

The DOI matches its Crossref record.
Bone morphogenetic protein 2-induced human dental pulp cell differentiation involves p38 mitogen-activated protein kinase-activated canonical WNT pathway
Open accessAbstract
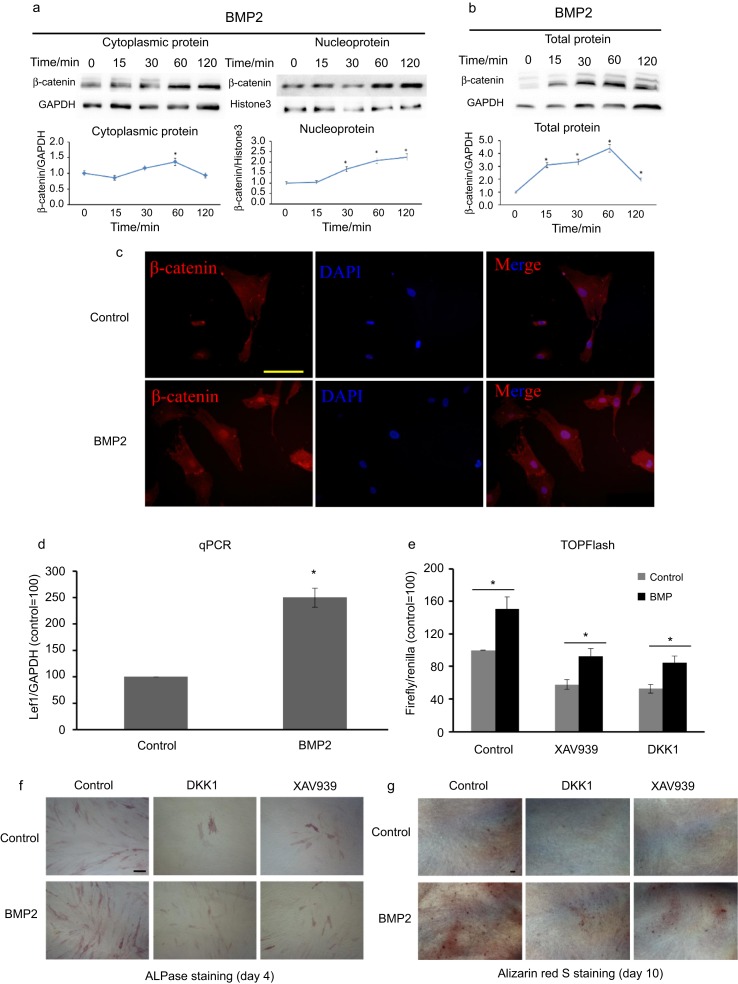
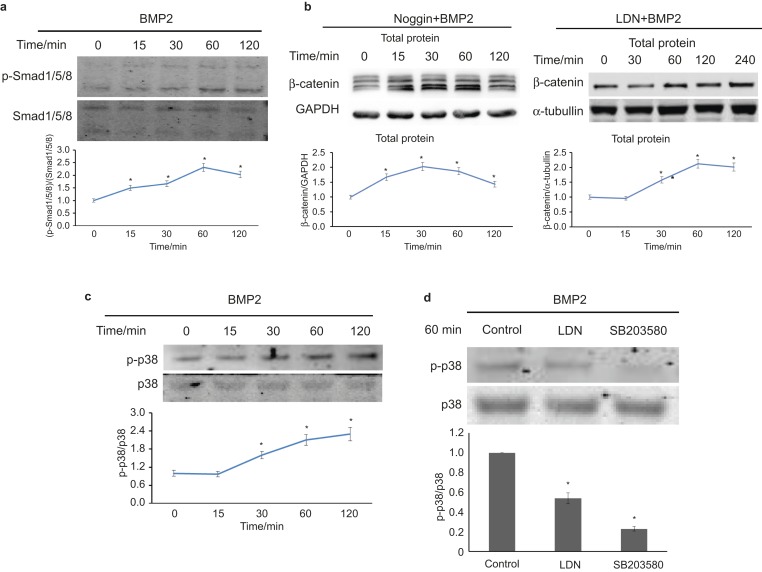
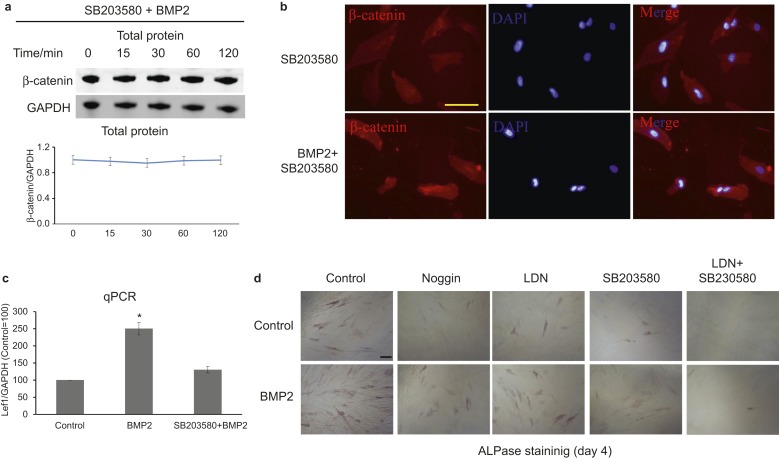
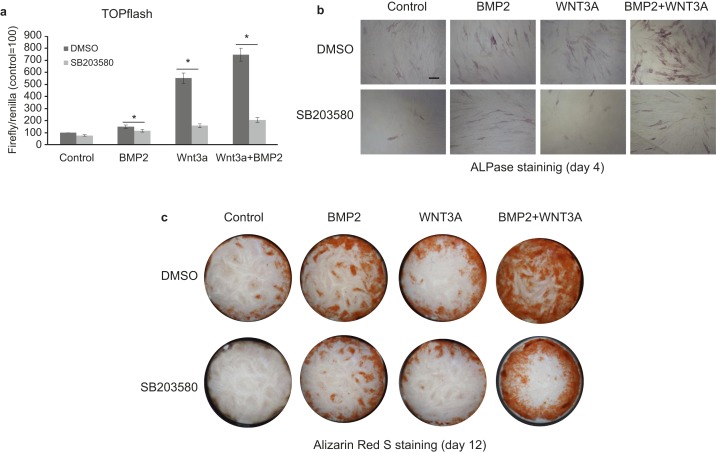
Both bone morphogenetic protein 2 (BMP2) and the wingless-type MMTV integration site (WNT)/β-catenin signalling pathway play important roles in odontoblast differentiation and dentinogenesis. Cross-talk between BMP2 and WNT/β-catenin in osteoblast differentiation and bone formation has been identified. However, the roles and mechanisms of the canonical WNT pathway in the regulation of BMP2 in dental pulp injury and repair remain largely unknown. Here, we demonstrate that BMP2 promotes the differentiation of human dental pulp cells (HDPCs) by activating WNT/β-catenin signalling, which is further mediated by p38 mitogen-activated protein kinase (MAPK) in vitro. BMP2 stimulation upregulated the expression of β-catenin in HDPCs, which was abolished by SB203580 but not by Noggin or LDN193189. Furthermore, BMP2 enhanced cell differentiation, which was not fully inhibited by Noggin or LDN193189. Instead, SB203580 partially blocked BMP2-induced β-catenin expression and cell differentiation. Taken together, these data suggest a possible mechanism by which the elevation of β-catenin resulting from BMP2 stimulation is mediated by the p38 MAPK pathway, which sheds light on the molecular mechanisms of BMP2-mediated pulp reparative dentin formation. Researchers have clarified the molecular interactions that underpin the formation and regeneration of dentin in human teeth. Dentin is the layer of calcified tissue directly beneath the surface enamel of a tooth. It is formed and sustained by the differentiation of cells in the tooth pulp that lies beneath the dentin layer. Chenglin Wang and co-workers at Sichuan University in China, with colleagues at Columbia University, New York, USA, studied human dental pulp cells in vitro. They demonstrated that bone morphogenetic protein 2 (BMP2) promotes the differentiation of pulp cells to form dentin by affecting signaling pathways known to be involved. Identifying the links between the growth factor BMP2, and β-catenin and p38, proteins in these pathways, will improve understanding of dentin formation and repair after injury.
Overview
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
The cited source says what the claim attributes to it.
In the citing paper
“Furthermore, multiple studies have provided evidence of the involvement of MAPK in modulating the activities of the Wnt/β-catenin pathway.”
From Multiple myeloma: signaling pathways and targeted therapy (2024) · cites this paper as [134]
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
No references could be resolved yet.
Research works printed but not linked: 56
- Mao JJ, Robey PG, Prockop DJ . Stem cells in the face: tooth regeneration and beyond. Cell Stem Cell 2012 ; 11 ( 3 ): 291 – 301 . · DOI
- Gronthos S, Mankani M, Brahim J et al . Postnatal human dental pulp stem cells (DPSCs) in vitro and in vivo. Proc Natl Acad Sci USA 2000 ; 97 ( 25 ): 13625 – 13630 . · DOI
- Mann LM, Lennon DP, Caplan AI . Cultured rat pulp cells have the potential to form bone, cartilage, and dentin in vivo //Davidovitch Z, Norton LA eds . Biological mechanisms of tooth movement and craniofacial adaptation . Boston: Harvard Society of the Advancement of Orthodontics, 1996 : 7 – 10 .
- Yildirim S, Fu SY, Kim K et al . Tooth regeneration: a revolution in stomatology and evolution in regenerative medicine. Int J Oral Sci 2011 ; 3 ( 3 ): 107 – 116 . · DOI
- Peng L, Ye L, Zhou XD . Mesenchymal stem cells and tooth engineering. Int J Oral Sci 2009 ; 1 ( 1 ): 6 – 12 . · DOI
- Sloan AJ, Smith AJ . Stem cells and the dental pulp: potential roles in dentine regeneration and repair. Oral Dis 2007 ; 13 ( 2 ): 151 – 157 . · DOI
- Smith AJ, Lesot H . Induction and regulation of crown dentinogenesis: embryonic events as a template for dental tissue repair? Crit Rev Oral Biol Med 2001 ; 12 ( 5 ): 425 – 437 . · DOI
- Saito T, Ogawa M, Hata Y et al . Acceleration effect of human recombinant bone morphogenetic protein-2 on differentiation of human pulp cells into odontoblasts. J Endod 2004 ; 30 ( 4 ): 205 – 208 . · DOI
- Qin W, Yang F, Deng R et al . Smad 1/5 is involved in bone morphogenetic protein-2-induced odontoblastic differentiation in human dental pulp cells. J Endod 2012 ; 38 ( 1 ): 66 – 71 . · DOI
- Li J, Huang X, Xu X et al . SMAD4-mediated WNT signaling controls the fate of cranial neural crest cells during tooth morphogenesis. Development 2011 ; 138 ( 10 ): 1977 – 1989 . · DOI
- Qin W, Liu P, Zhang R et al . JNK MAPK is involved in BMP2-induced odontoblastic differentiation of human dental pulp cells. Connect Tissue Res 2014 ; 55 ( 3 ): 217 – 224 . · DOI
- Nakashima M . Bone morphogenetic proteins in dentin regeneration for potential use in endodontic therapy. Cytokine Growth Factor Rev 2005 ; 16 ( 3 ): 369 – 376 . · DOI
- Chen D, Zhao M, Mundy GR . Bone morphogenetic proteins. Growth Factors 2004 ; 22 ( 4 ): 233 – 241 . · DOI
- Nakashima M, Reddi AH . The application of bone morphogenetic proteins to dental tissue engineering. Nat Biotechnol 2003 ; 21 ( 9 ): 1025 – 1032 . · DOI
- Gautschi OP, Frey SP, Zellweger R . Bone morphogenetic proteins in clinical applications. ANZ J Surg 2007 ; 77 ( 8 ): 626 – 631 . · DOI
- Bègue-Kirn C, Smith AJ, Loriot M et al . Comparative analysis of TGF beta s, BMPs, IGF1, msxs, fibronectin, osteonectin and bone sialoprotein gene expression during normal and in vitro-induced odontoblast differentiation. Int J Dev Biol 1994 ; 38 ( 3 ): 405 – 420 .
- Iohara K, Nakashima M, Ito M et al . Dentin regeneration by dental pulp stem cell therapy with recombinant human bone morphogenetic protein 2. J Dent Res 2004 ; 83 ( 8 ): 590 – 595 . · DOI
- Yang W, Harris MA, Cui Y et al . BMP2 is required for odontoblast differentiation and pulp vasculogenesis. J Dent Res 2012 ; 91 ( 1 ): 58 – 64 . · DOI
- Chen J, Lan Y, Baek JA et al . Wnt/beta-catenin signaling plays an essential role in activation of odontogenic mesenchyme during early tooth development. Dev Biol 2009 ; 334 ( 1 ): 174 – 185 . · DOI
- Tamura M, Nemoto E, Sato MM et al . Role of the Wnt signaling pathway in bone and tooth. Front Biosci: Elite Ed 2010 ; 2 : 1405 – 1413 . · DOI
- Mbalaviele G, Sheikh S, Stains JP et al . Beta-catenin and BMP2 synergize to promote osteoblast differentiation and new bone formation. J Cell Biochem 2005 ; 94 ( 2 ): 403 – 418 . · DOI
- Chen D, Harris MA, Rossini G et al . Bone morphogenetic protein 2 (BMP2) enhances BMP3, BMP4, and bone cell differentiation marker gene expression during the induction of mineralized bone matrix formation in cultures of fetal rat calvarial osteoblasts. Calcif Tissue Int 1997 ; 60 ( 3 ): 283 – 290 . · DOI
- Chen D, Ji X, Harris MA et al . Differential roles for bone morphogenetic protein (BMP) receptor type IB and IA in differentiation and specification of mesenchymal precursor cells to osteoblast and adipocyte lineages. J Cell Biol 1998 ; 142 ( 1 ): 295 – 305 . · DOI
- Zhao M, Harris SE, Horn D et al . Bone morphogenetic protein receptor signaling is necessary for normal murine postnatal bone formation. J Cell Biol 2002 ; 157 ( 6 ): 1049 – 1060 . · DOI
- Rawadi G, Vayssière B, Dunn F et al . BMP2 controls alkaline phosphatase expression and osteoblast mineralization by a Wnt autocrine loop. J Bone Miner Res 2003 ; 18 ( 10 ): 1842 – 1853 . · DOI
- Zhang M, Yan Y, Lim YB et al . BMP2 modulates beta-catenin signaling through stimulation of Lrp5 expression and inhibition of beta-TrCP expression in osteoblasts. J Cell Biochem 2009 ; 108 ( 4 ): 896 – 905 . · DOI
- Scheller EL, Chang J, Wang CY . Wnt/beta-catenin inhibits dental pulp stem cell differentiation. J Dent Res 2008 ; 87 ( 2 ): 126 – 130 . · DOI
- Silvério KG, Davidson KC, James RG et al . Wnt/β-catenin pathway regulates bone morphogenetic protein (BMP2)-mediated differentiation of dental follicle cells. J Periodont Res 2012 ; 47 ( 3 ): 309 – 319 . · DOI
- Hildesheim J, Salvador JM, Hollander MC et al . Casein kinase 2- and protein kinase A-regulated adenomatous polyposis coli and beta-catenin cellular localization is dependent on p38 MAPK. J Biol Chem 2005 ; 280 ( 17 ): 17221 – 17226 . · DOI
- Bikkavilli RK, Feigin ME, Malbon CC . G alpha o mediates WNT-JNK signaling through dishevelled 1 and 3, RhoA family members, and MEKK 1 and 4 in mammalian cells . J Cell Sci 2008 ; 121 ( Pt 2 ): 234 – 245 . · DOI
- Caverzasio J, Manen D . Essential role of Wnt3a-mediated activation of mitogen-activated protein kinase p38 for the stimulation of alkaline phosphatase activity and matrix mineralization in C3H10T1/2 mesenchymal cells. Endocrinology 2007 ; 148 ( 11 ): 5323 – 5330 . · DOI
- Keren A, Bengal E, Frank D . p38 MAP kinase regulates the expression of XMyf5 and affects distinct myogenic programs during Xenopus development. Dev Biol 2005 ; 288 ( 1 ): 73 – 86 . · DOI
- Bikkavilli RK, Feigin ME, Malbon CC . p38 mitogen-activated protein kinase regulates canonical Wnt-beta-catenin signaling by inactivation of GSK3beta . J Cell Sci 2008 ; 121 ( Pt 21 ): 3598 – 3607 . · DOI
- Chang J, Sonoyama W, Wang Z et al . Noncanonical Wnt-4 signaling enhances bone regeneration of mesenchymal stem cells in craniofacial defects through activation of p38 MAPK. J Biol Chem 2007 ; 282 ( 42 ): 30938 – 30948 . · DOI
- Jin EJ, Lee SY, Choi YA et al . BMP2-enhanced chondrogenesis involves p38 MAPK-mediated down-regulation of Wnt-7a pathway. Mol Cells 2006 ; 22 ( 3 ): 353 – 359 . · DOI
- Couble ML, Farges JC, Bleicher F et al . Odontoblast differentiation of human dental pulp cells in explant cultures. Calcif Tissue Int 2000 ; 66 ( 2 ): 129 – 138 . · DOI
- Han N, Zheng Y, Li R et al . β-catenin enhances odontoblastic differentiation of dental pulp cells through activation of Runx2. PLoS One 2014 ; 9 ( 2 ): e88890 . · DOI
- Nakashima M, Nagasawa H, Yamada Y et al . Regulatory role of transforming growth factor-beta, bone morphogenetic protein-2, and protein-4 on gene expression of extracellular matrix proteins and differentiation of dental pulp cells. Dev Biol 1994 ; 162 ( 1 ): 18 – 28 . · DOI
- Liu J, Jin T, Ritchie HH et al . In vitro differentiation and mineralization of human dental pulp cells induced by dentin extract. In Vitro Cell Dev Biol Anim 2005 ; 41 ( 7 ): 232 – 238 . · DOI
- Zhang W, Walboomers XF, Wolke JG et al . Differentiation ability of rat postnatal dental pulp cells in vitro. Tissue Eng 2005 ; 11 ( 3/4 ): 357 – 368 . · DOI
- Kido J, Ishida H, Nagata T et al . Effects of parathyroid hormone, 1,25-dihydroxyvitamin D3, and prostaglandin E2 on alkaline phosphatase activity in cultured dental pulp and gingiva cells of bovine calf. J Endod 1991 ; 17 ( 4 ): 161 – 164 . · DOI
- Handrigan GR, Richman JM . A network of Wnt, hedgehog and BMP signaling pathways regulates tooth replacement in snakes. Dev Biol 2010 ; 348 ( 1 ): 130 – 141 . · DOI
- Silvério KG, Davidson KC, James RG et al . Wnt/β-catenin pathway regulates bone morphogenetic protein (BMP2)-mediated differentiation of dental follicle cells. J Periodont Res 2012 ; 47 ( 3 ): 309 – 319 . · DOI
- Kamiya N, Ye L, Kobayashi T et al . BMP signaling negatively regulates bone mass through sclerostin by inhibiting the canonical Wnt pathway. Development 2008 ; 135 ( 22 ): 3801 – 3811 . · DOI
- Tang N, Song WX, Luo J et al . BMP9-induced osteogenic differentiation of mesenchymal progenitors requires functional canonical Wnt/beta-catenin signalling. J Cell Mol Med 2009 ; 13 ( 8B ): 2448 – 2464 . · DOI
- Nakashima A, Katagiri T, Tamura M . Cross-talk between Wnt and bone morphogenetic protein 2 (BMP2) signaling in differentiation pathway of C2C12 myoblasts. J Biol Chem 2005 ; 280 ( 45 ): 37660 – 37668 . · DOI
- Hill TP, Später D, Taketo MM et al . Canonical Wnt/beta-catenin signaling prevents osteoblasts from differentiating into chondrocytes. Dev Cell 2005 ; 8 ( 5 ): 727 – 738 . · DOI
- Bain G, Müller T, Wang X et al . Activated beta-catenin induces osteoblast differentiation of C3H10T1/2 cells and participates in BMP2 mediated signal transduction. Biochem Biophys Res Commun 2003 ; 301 ( 1 ): 84 – 91 . · DOI
- Semënov MV, Tamai K, Brott BK et al . Head inducer Dickkopf-1 is a ligand for Wnt coreceptor LRP6. Curr Biol 2001 ; 11 ( 12 ): 951 – 961 . · DOI · Paper page
- Mao B, Wu W, Li Y et al . LDL-receptor-related protein 6 is a receptor for Dickkopf proteins. Nature 2001 ; 411 ( 6835 ): 321 – 325 . · DOI
- Xiao YT, Xiang LX, Shao JZ . Bone morphogenetic protein. Biochem Biophys Res Commun 2007 ; 362 ( 3 ): 550 – 553 . · DOI
- Wu XB, Li Y, Schneider A et al . Impaired osteoblastic differentiation, reduced bone formation, and severe osteoporosis in noggin-overexpressing mice. J Clin Invest 2003 ; 112 ( 6 ): 924 – 934 . · DOI
- Devlin RD, Du Z, Pereira RC et al . Skeletal overexpression of noggin results in osteopenia and reduced bone formation. Endocrinology 2003 ; 144 ( 5 ): 1972 – 1978 . · DOI
- Hassel S, Schmitt S, Hartung A et al . Initiation of Smad-dependent and Smad-independent signaling via distinct BMP-receptor complexes . J Bone Joint Surg Am 2003 ; 85 ( Suppl 3 ): 44 – 51 . · DOI
- Rosen V . BMP2 signaling in bone development and repair. Cytokine Growth Factor Rev 2009 ; 20 ( 5/6 ): 475 – 480 . · DOI
- Su Y, Xie W, Wang C et al . JNK/P38 mitogen-activated protein kinase used for hepatocyte growth factor-induced proliferation, differentiation, and migration in human dental papilla cells. J Endod 2012 ; 38 ( 9 ): 1207 – 1213 . · DOI
Cited by
Sorted by citations
Multiple myeloma: signaling pathways and targeted therapy
Lu, Q., Yang, D., Li, H., Niu, T., & Tong, A. (2024) · Molecular biomedicine · doi:10.1186/s43556-024-00188-w · Cited by 90
Self-citation
Metadata
- Authors
- Yang, J., Ye, L., Hui, T.-Q., Yang, D.-M., Huang, D.-M., Zhou, X.-D., Mao, J. J., & Wang, C.-L.
- Affiliations
- Sichuan University (CN)
- Columbia University Irving Medical Center (US)
- Venue
- International Journal of Oral Science
- Published
- 2015-06
- Volume
- 7
- Issue
- 2
- Pages
- 95-102
- ISSN
- 1674-2818 (ISSN-L)
- 2049-3169
- PMC
- PMC4817555
- OpenAlex
- W2408014337
- Cited by
- 68
- References
- 0
- Citations by year
- 2026: 5 · 2025: 5 · 2024: 6 · 2023: 7 · 2022: 4 · 2021: 9 · 2020: 7 · 2019: 5 · 2018: 5 · 2017: 7 · 2016: 7 · 2015: 1
- FWCI
- 2.90
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Licence
- Locations
- International Journal of Oral Science (publishedVersion, cc-by-nc-sa)
- PubMed Central (publishedVersion, cc-by-nc-sa)
- PubMed (publishedVersion)
- Funders
- National Natural Science Foundation of China (813220170, 81070801, 81200759)
- Education Department of Sichuan Province (13TD0038)
- Sichuan Province Science and Technology Support Program
- Topics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Wnt/β-catenin signaling in development and cancer
- Health Sciences › Dentistry › Oral Surgery › Endodontics and Root Canal Treatments
- Health Sciences › Dentistry › General Dentistry › dental development and anomalies
- Keywords
- BMP-2, Wnt/β-catenin signaling, p38 MAPK, human dental pulp cells, odontoblast differentiation, dentin formation, pulp repair, β-catenin, SB203580, noggin, LDN-193189
- MeSH terms
- Cell Differentiation, Dental Pulp, Humans, MAP Kinase Signaling System, Wnt Proteins, beta Catenin, Bone Morphogenetic Protein 2
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
