

The DOI matches its Crossref record; 98 of the 102 references it cites were found in a registry or an index; none of the 90 sources its claims cite is checked for support yet.
Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils
Open accessAbstract
Cyanobacteria are among the most ancient of evolutionary lineages, oxygenic photosynthesizers that may have originated before 3.0 Ga, as evidenced by free oxygen levels. Throughout the P recambrian, cyanobacteria were one of the most important drivers of biological innovations, strongly impacting early Earth's environments. At the end of the A rchean E on, they were responsible for the rapid oxygenation of Earth's atmosphere during an episode referred to as the G reat O xidation E vent (GOE). However, little is known about the origin and diversity of early cyanobacterial taxa, due to: (1) the scarceness of P recambrian fossil deposits; (2) limited characteristics for the identification of taxa; and (3) the poor preservation of ancient microfossils. Previous studies based on 16 S r RNA have suggested that the origin of multicellularity within cyanobacteria might have been associated with the GOE. However, single‐gene analyses have limitations, particularly for deep branches. We reconstructed the evolutionary history of cyanobacteria using genome scale data and re‐evaluated the P recambrian fossil record to get more precise calibrations for a relaxed clock analysis. For the phylogenomic reconstructions, we identified 756 conserved gene sequences in 65 cyanobacterial taxa, of which eight genomes have been sequenced in this study. Character state reconstructions based on maximum likelihood and Bayesian phylogenetic inference confirm previous findings, of an ancient multicellular cyanobacterial lineage ancestral to the majority of modern cyanobacteria. Relaxed clock analyses provide firm support for an origin of cyanobacteria in the A rchean and a transition to multicellularity before the GOE. It is likely that multicellularity had a greater impact on cyanobacterial fitness and thus abundance, than previously assumed. Multicellularity, as a major evolutionary innovation, forming a novel unit for selection to act upon, may have served to overcome evolutionary constraints and enabled diversification of the variety of morphotypes seen in cyanobacteria today.
Overview
AI snapshot
Written from the paper’s full text.
TL;DR
Genome-scale phylogenomics and relaxed molecular clock analyses of 65 cyanobacterial taxa support an Archean origin of cyanobacteria and an origin of multicellularity before the Great Oxidation Event, with multicellularity later lost and occasionally regained. The authors argue this early multicellularity may have increased cyanobacterial abundance and oxygen production, contributing to the GOE.
Key findings
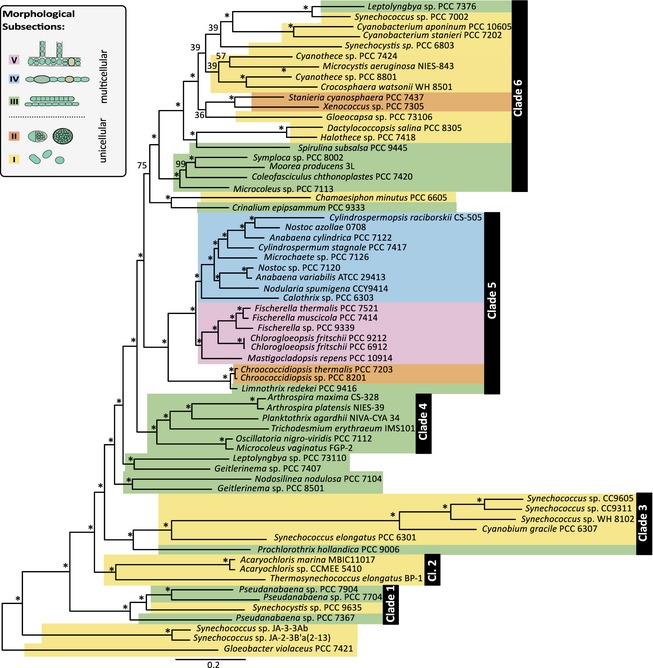
- The phylogenomic tree, based on 756 conserved proteins (197,761 amino acid sites) from 65 cyanobacterial taxa, recovered six major clades with full bootstrap support; 100% maximum likelihood bootstrap support was inferred for 57 of 64 branches, compared with 24 of 64 branches in the 16S/23S rRNA tree.
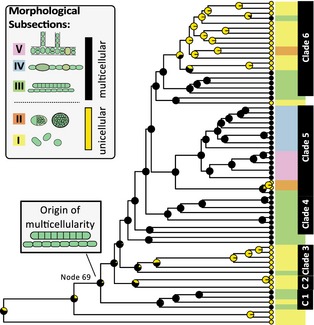
- Ancestral character state reconstruction inferred a very early transition to multicellularity at node/branch 69; multicellularity was subsequently lost at least five times and regained on one, possibly two, branches leading to *Leptolyngbya* sp. PCC 7376 and *Spirulina subsalsa* PCC 9445, so the majority of modern cyanobacteria are descendants of an ancient multicellular lineage.
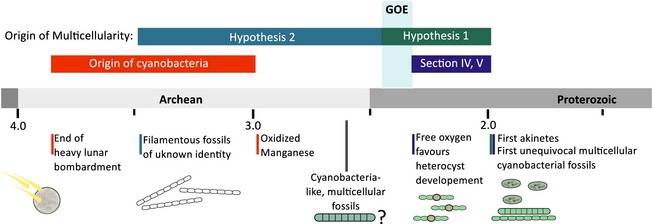
- Relaxed clock analyses, irrespective of prior assumptions for node 69, estimated that multicellularity originated before the GOE; cyanobacteria originated in the Archean/mid-Archean long before the GOE, and the majority of modern clades 2–6 evolved after the GOE.
- Comparisons of modern cyanobacterial cell sizes to Precambrian microfossils support the inferred presence of multicellular cyanobacteria before the GOE, but the fossil record does not provide evidence for multicellular taxa among the earliest unequivocal fossil assemblages at 3.33–3.45 Ga.
Methods
- Taxon sampling and phylogenomics: 65 cyanobacterial taxa were analyzed, including 27 unicellular (sections I–II) and 38 multicellular (sections III–V) taxa; eight additional cyanobacterial genomes were sequenced. A total of 756 highly conserved proteins were identified, aligned, and concatenated into a 197,761-amino-acid supermatrix; maximum likelihood trees were reconstructed with RAxML using the LG + Γ model and 1000 bootstrap resamplings, alongside a concatenated 16S/23S rRNA tree.
- Ancestral character state reconstruction: maximum likelihood methods in the R ape package and Bayesian inference in BayesTraits were used; MCMC analyses ran for 1,010,000 iterations with a 10,000 burn-in, estimating transition rates q01 (to multicellularity) and q10 (to unicellularity).
- Divergence time estimation: relaxed clocks with lognormal rate distribution were applied in MCMCTREE/PAML, using three calibrations—origin of Cyanobacteria, origin of sections IV and V capable of cellular differentiation, and origin of multicellularity at node 69. Two hypotheses were tested: multicellularity after the GOE (H1) versus before the GOE (H2); four MCMC analyses ran for 10 million generations, sampling every 100 generations with 50% burn-in.
Limitations
- Stated: deep divergences are limited by the lack of evolutionary information retained in molecular data over long timescales, weaknesses in phylogenetic models, paucity of calibration points, potential misassignment of calibrations, and the likelihood that fossil ages poorly approximate clade ages; posterior node age estimates had large 95% confidence intervals that prevented precise dating.
- Stated: the Precambrian fossil record is patchy at best; the earliest unequivocal fossil assemblages at 3.33–3.45 Ga do not provide evidence for multicellular cyanobacteria, and filament diameters in older fossils are described as “more probabilistic than deterministic” evidence for cyanobacteria.
- Evident from the text: the analyses depend on debated fossil interpretations and geochemical inferences for calibration, use only uniform prior distributions, and showed that user-specified priors can differ from effective priors, although the authors judged the age ranges similar enough to accept.
Model-written summary. Check it against the paper before relying on it.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
59 Not checked yet · 29 Own result · 22 Own interpretation · 11 No basis given · 3 Own method
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Relaxed clock analyses provide firm support for an origin of cyanobacteria in the Archean and a transition to multicellularity before the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- The authors state this as an assumption: The divergence of the Gloeobacter lineage from the stem lineage leading to all other extant cyanobacteria occurred between 3.85 and 2.918 Ga (analyses A, C) or between 3.85 and 2.45 Ga (analyses B, D).
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Relaxed clock analyses provide firm support for an origin of cyanobacteria in the Archean and a transition to multicellularity before the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- The authors state this as an assumption: The most recent common ancestor of subsections IV and V cyanobacteria originated after the GOE but before 1.957 Ga.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Results of all analyses suggest a very early transition to multicellularity at ‘node/branch 69’ (Fig. 3; Fig. S3; Table S3).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Changing the widths of the uniform distribution in several runs supported an early transition to multicellularity even further (Fig. S3, online Supporting Information).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Assuming that Gloeobacter groups closest to a eubacterial outgroup, as previously suggested based on ribosomal (Schirrmeister et al. 2011b), and phylogenomic data (Blank and Sanchez‐Baracaldo 2010; Shih et al. 2013), Synechococcus isolated from hot springs are the first group to split from the rest of Cyanobacteria, followed by an early branching ‘Clade 1’ of unicellular and multicellular cyan”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
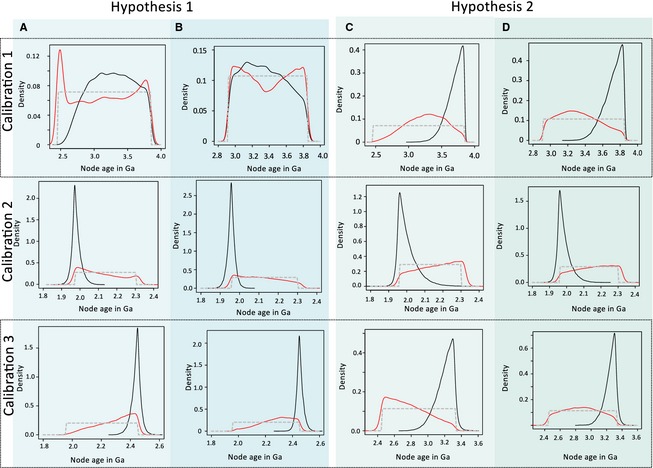
“Our analyses run without molecular data showed that our originally uniform priors (Fig. 4; dashed curve) resulted in non‐uniform effective priors (Fig. 4; red curve).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“For character state reconstructions using an asymmetrical rate model, the estimated rates were q01 = 0.5768 (standard error = 0.3147) and q10 = 0.8254 (standard error = 0.2205), where q01 defines the transition to multicellularity and q01 the loss of multicellularity.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Six distinct clades could be reconstructed with full support.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Phylogenomic analyses using a supermatrix
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“In all analyses, the posterior probabilities of the origin of multicellularity (calibration 3; Fig. 4) support an age close to the maximum of the prior age calibration.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The posterior age estimates for the origin of multicellularity (calibration 3) are in all cases shifted towards the older bound of the effective priors.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Several forms of genera appear polyphyletic, such as Synechococcus, Geitlerinema and Pseudanabaena.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The majority of branches in this phylogeny are well supported.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Phylogenomic analyses using a supermatrix
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“In all analyses, subsections IV and V capable of cellular differentiation (calibration 2; Fig. 4) have a higher probability of origination close to the minimum age range of our specified prior calibration (1.9–2.1 Ga).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- The authors state this as an assumption: The most recent common ancestor of subsections IV and V cyanobacteria originated after the GOE but before 1.957 Ga.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Phylogenomic results show increased tree support compared to single‐gene analyses and confirm previous suggestions of early multicellularity in cyanobacteria (Schirrmeister et al. 2013).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Differentiated cyanobacteria belonging to subsections IV and V are the only groups where morphological and genomic data congruently suggest a monophyletic origin.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Phylogenomic analyses using a supermatrix
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Phylogenomic results show increased tree support compared to single‐gene analyses and confirm previous suggestions of early multicellularity in cyanobacteria (Schirrmeister et al. 2013).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“However, if this node was not used for calibration, a younger age is estimated (0.8–1.6 Ga; Fig. S4).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Monophyly of cyanobacteria forming heterocysts and akinetes is confirmed in this study.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of terminal cell differentiation (calibration 2)
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Phylogenomic data fully support monophyly of subsections IV and V cyanobacteria capable of cellular differentiation.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Clades 1–6 (this study) can be directly compared to clades (A–C, E, F) reconstructed by Shih et al. (2013).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“a younger age is estimated (0.8–1.6 Ga; Fig. S4).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“In comparison with the previous analyses based on 16S rRNA data (Schirrmeister et al. 2013), confidence intervals are smaller in general, particularly those of deep node ages.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
What the sources say
- Not checked yetcites Schirrmeister et al. 2013
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
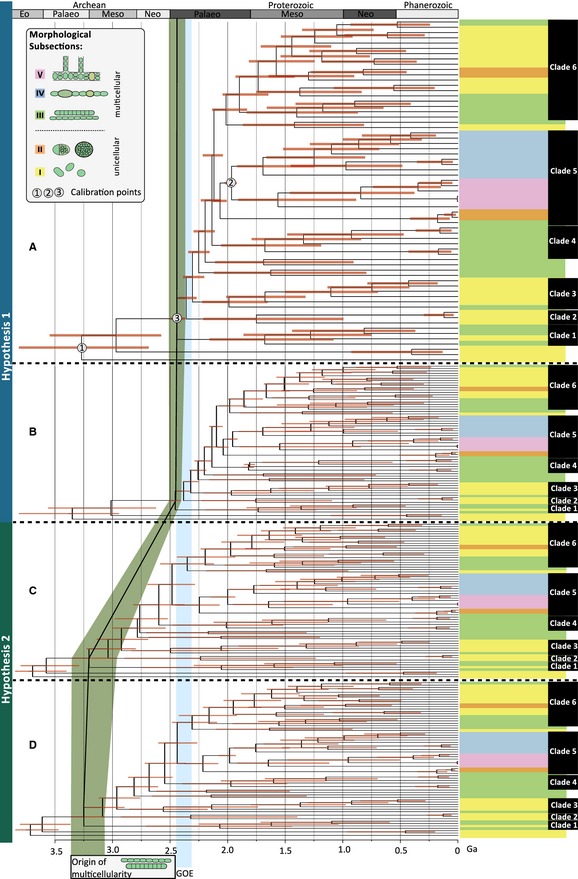
“Nevertheless, all analyses, irrespective of the prior assumptions applied for ‘node 69’, point to an origin of multicellularity in cyanobacteria before the GOE (Fig. 5).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Different widths for the calibration of the root (A, C vs. B, D in Fig. 5) did not affect age estimates for node 69”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“whereas in Hypothesis 1 a calibration of the root between 3.85 and 2.958 resulted in a mean estimate of 235 million years older age for node 69 with wider posterior probability distribution.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Posterior node age estimates show large 95% confidence intervals, which prevents a precise dating of divergence events.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The majority of modern cyanobacterial clades (clades 2–6) have evolved after the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“our results agree with the previous estimates of an origin of marine picocyanobacteria around the end of the Mesoproterozoic (Sanchez‐Baracaldo et al. 2014), although confidence intervals are too broad to specify dates, further.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
What the sources say
- Not checked yetcites Sanchez‐Baracaldo et al. 2014
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“At the end of the Archean Eon, they were responsible for the rapid oxygenation of Earth's atmosphere during an episode referred to as the Great Oxidation Event (GOE).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Bekker et al. 2004
- Not checked yetcites Anbar et al. 2007
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Furthermore, 2.0 Ga fossilized resting cells (present in subsections IV and V), termed ‘Archaeoellipsoides’, resemble akinetes of modern subsection IV cyanobacterial genus Anabaena (Amard and Bertrand‐Sarfati 1997).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Amard and Bertrand‐Sarfati 1997
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Fossil cyanobacteria from almost all subsections have been found in Mesoproterozoic deposits (Schopf and Blacic 1971; Horodyski and Donaldson 1980; Butterfield 2000).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Schopf and Blacic 1971
- Not checked yetcites Horodyski and Donaldson 1980
- Not checked yetcites Butterfield 2000
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“In heterotrophic prokaryotes, metabolic rates have been found to increase superlinearly with body mass (DeLong et al. 2010).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites DeLong et al. 2010
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Cyanobacteria belonging to subsections I and III have been identified in the early Proterozoic including the 1.8 Ga Duck Creek Dolomite in Australia (Knoll et al. 1988) and 1.9 Ga Belcher Supergroup in Canada (Hofmann 1976).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Knoll et al. 1988
- Not checked yetcites Hofmann 1976
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Unfortunately, attempts to resolve the early evolutionary history of life using molecular phylogenetic approaches has reached contradictory conclusions due to a lack of data and weaknesses in methodology (Schirrmeister et al. 2013; Shih and Matzke 2013).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Schirrmeister et al. 2013
- Not checked yetcites Shih and Matzke 2013
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The diversity of cyanobacterial taxa soon after the GOE indicates an origin of cyanobacterial ancestors some time in the Archean.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“However, single‐gene analyses have limitations, particularly for deep branches.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Schirrmeister et al. 2013
- Not checked yetcites Shih and Matzke 2013
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“During the early Proterozoic, 2.5–2.3 Ga, atmospheric oxygen levels accumulated rapidly during an episode coined the Great Oxidation Event (GOE; Bekker et al. 2004; Anbar et al. 2007) as a result of cyanobacterial activity leading to great changes to the Earth system (Van Kranendonk et al. 2012), subsequently allowing for the evolutionary emergence of complex life as we know it.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Bekker et al. 2004
- Not checked yetcites Anbar et al. 2007
- Not checked yetcites Van Kranendonk et al. 2012
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“It is likely that multicellularity had a greater impact on cyanobacterial fitness and thus abundance, than previously assumed.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“This variety in shapes allows for a fairly reliable identification of cyanobacterial relatives in the fossil record compared to other prokaryotes.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Additionally, Warnock et al. (2012, 2015) pointed out that programs for molecular clock analyses will truncate prior calibrations so that prior age distributions agree with the occurrences of divergence events in the phylogeny.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
What the sources say
- Not checked yetcites Warnock et al. 2012
- Not checked yetcites Warnock et al. 2015
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Therefore, the joint (effective) calibration priors may differ substantially from the user‐specified priors.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
What the sources say
- Not checked yetcites Warnock et al. 2012
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Filament diameters of these fossils are more probabilistic than deterministic as evidence for the presence of cyanobacteria.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > The evolution of multicellularity – testing two hypotheses (calibration 3)
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Fossil resting cells, so called akinetes, only present in cyanobacteria capable of heterocyst formation (subsections IV and V; Fig. 1) have been described from c. 2.1 Ga Franceville Group, Gabon (Amard and Bertrand‐Sarfati 1997; Sergeev 2009).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of terminal cell differentiation (calibration 2)
What the sources say
- Not checked yetcites Amard and Bertrand‐Sarfati 1997
- Not checked yetcites Sergeev 2009
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Hence, the majority of modern cyanobacteria are descendants of an ancient multicellular lineage.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“The upper limit represents the latest ending of the Late Heavy Bombardment, based on estimates for the end of the strong meteorite bombardment of the moon (Stöffler and Ryder 2001; Chapman et al. 2007).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
What the sources say
- Not checked yetcites Stöffler and Ryder 2001
- Not checked yetcites Chapman et al. 2007
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Divergence time results are strongly affected by parameter choice if non‐uniform prior calibration densities, such as lognormal, are employed (Warnock et al. 2012, 2015); therefore, only uniform distributions were applied in this study.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
What the sources say
- Not checked yetcites Warnock et al. 2012
- Not checked yetcites Warnock et al. 2015
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Based on U–Pb zircon ages, rocks containing these Mo signatures were formed at a minimum of 2.940 Ga ± 0.022 Gyr (Hegner et al. 1984).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
What the sources say
- Not checked yetcites Hegner et al. 1984
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Filamentous fossils from the 3.42–3.35 Ga found in the Strelley Pool Formation, Australia (Wacey et al. 2011; Sugitani et al. 2013), Barberton Greenstone Belt, South Africa (Walsh 1992; Westall et al. 2001; Westall et al. 2006), and possibly earlier (Awramik et al. 1988; Schopf and Kudryavtsev 2009) evidence the presence of multicellular prokaryotes.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > The evolution of multicellularity – testing two hypotheses (calibration 3)
What the sources say
- Not checked yetcites Wacey et al. 2011
- Not checked yetcites Sugitani et al. 2013
- Not checked yetcites Walsh 1992
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Carbon isotope analyses from rocks of similar age, such as Mushandike, Zimbabwe, and Steep Rock, Canada, further support an early presence of oxygen as a result of oxygenic photosynthesis (Nisbet et al. 2007; Nisbet and Nisbet 2008).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
What the sources say
- Not checked yetcites Nisbet et al. 2007
- Not checked yetcites Nisbet and Nisbet 2008
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“While an occurrence of larger tubes (10–20 μm) has been observed in 3.4 Ga deposits from Western Australia, these show few characteristics to link them to modern prokaryotic taxa.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Geochemical evidence, based on Mo and Fe isotopes, supports an early evolution of oxygenic photosynthesis (Nisbet and Fowler 2011).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Nisbet and Fowler 2011
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Modern cyanobacteria exhibit a wide range of cell sizes which, on average, exceeds sizes found among most prokaryotes (<2 μm; Castenholz 2001).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Castenholz 2001
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“their results are based on merely two subunits of one enzyme (c. 986 amino acids).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Shih and Matzke (2013)
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“In c. 2.0 Ma deposits from Western Australia, filaments of large size (63 μm in width) have been found and classified as Oscillatoriopsis majuscule (Knoll et al. 1988).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Knoll et al. 1988
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“over time it will become more likely that sequences saturate, which is a problem particularly for nucleotide sequences and deep branches (Xia et al. 2003).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Xia et al. 2003
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“The first larger, well‐preserved, multicellular morphotypes with cell widths of up to 28 μm can be observed in the 2.6 Ga Transvaal Group (Altermann and Schopf 1995).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Altermann and Schopf 1995
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“This has some significance for the interpretation of filamentous fossils as cyanobacteria based on their morphology, including those described from a range of sites at 2.0 Ga (Knoll et al. 1988; Lanier 1989; Amard and Bertrand‐Sarfati 1997) and potentially from the 2.6 Ga Transvaal Supergroup (Altermann and Schopf 1995) or even older (Awramik et al. 1988; Schopf and Kudryavtsev 2009).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Knoll et al. 1988
- Not checked yetcites Lanier 1989
- Not checked yetcites Amard and Bertrand‐Sarfati 1997
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“Often, sizes of unicellular taxa exceed those of fossilized filaments, as observed in deposits, such as Dismal Lake, Gunflint Chert, Belcher Supergroup and Barberton Supergroup (Hofmann 1976; Horodyski and Donaldson 1980; Lanier 1989; Walsh 1992).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Hofmann 1976
- Not checked yetcites Horodyski and Donaldson 1980
- Not checked yetcites Lanier 1989
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Fossils of such sizes resemble modern filamentous cyanobacterial sizes observed in the form of genera Lyngbya, Oscillatoria and Trichodesmium (Castenholz 2001).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Castenholz 2001
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“However, these results were based on a minimal data set of 16S ribosomal RNA sequences (1077–1090 nucleotide sites).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Therefore, the chances are high that phylogenetic information may have been lost due to multiple substitutions at the same nucleotide site (saturation).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“the reconstructed phylogenies depict the evolution of an enzyme and may result in strongly misleading inferences for species evolution.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“In early Archean deposits, such as in South Africa (3.33–3.46 Ga), fossil filament sizes do not exceed 5 μm (Walsh 1992; Westall et al. 2001).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Walsh 1992
- Not checked yetcites Westall et al. 2001
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“In modern mat communities, multicellular cyanobacteria, such as Oscillatoria and Phormidium, move vertically to position themselves in optimal light (Stal 1995).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Stal 1995
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
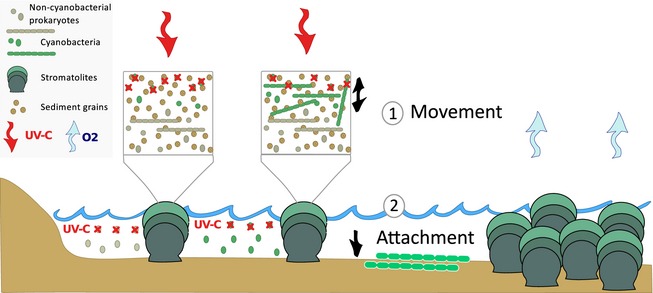
“Therefore, potential advantages of multicellularity such as: (1) movement and (2) improved substrate attachment in combination with potential increases in metabolic rates could have been the trigger for evolutionary success of cyanobacteria at the end of the Archean initiating the oxygenation of Earth.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
In the paper
“Cellular differentiation in Cyanobacteria, for example, can only evolve in a multicellular setting (Rossetti et al. 2010).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Rossetti et al. 2010
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Larger surface area of filamentous bacteria increases contact to the substrate which could have resulted in improved attachment (Young 2006).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Young 2006
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Furthermore, multicellularity may have been advantageous during initial substrate attachment at the beginning of mat formation (Fig. 6).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“During cyanobacterial evolution, UV radiation must have been a strong selective pressure resulting in several cyanobacterial taxa, today, that have developed a capability to protect themselves from UV‐A and UV‐B using pigments, such as scytonemin and shinorine (Sinha and Häder 2008; Balskus and Walsh 2010; Calteau et al. 2014; Rastogi et al. 2014).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Sinha and Häder 2008
- Not checked yetcites Balskus and Walsh 2010
- Not checked yetcites Calteau et al. 2014
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Improved attachment of filamentous cyanobacteria at the end of the Archean could have increased mat formation and consequently success of cyanobacterial taxa associated with those microbial communities.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Prior to the GOE, before an ozone shield was established, additional ultraviolet (UV) radiation between 200 and 300 nm (UV‐C) would have had lethal effects on organisms (Kasting and Catling 2003).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Kasting and Catling 2003
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The ability to move within the microbial mat, a characteristic that has been described for multicellular cyanobacteria, could have been of great advantage to avoid lethal radiation.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“Filamentous cyanobacteria of the genus Oscillatoria have been associated with initial substrate colonization during mat formation (Stal et al. 1985).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Stal et al. 1985
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“It has been shown that Fe (II) inhibits growth in Synechococcus cultures (Swanner et al. 2015).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Swanner et al. 2015
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“An observed delay in oxygen accumulation until the GOE could have been associated not only with oxygen sinks that remove oxygen, but possibly also with decreased evolutionary success of early Cyanobacteria.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Conclusion
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
In the paper
“As we have already observed, metabolic rates seem to increase superlinearly with size in heterotrophic bacteria (DeLong et al. 2010).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites DeLong et al. 2010
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- Probably not a substantial claim. 20
- It may state two separate claims as one. 34
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“An evolutionary model assuming equal transition rates resulted in rates of 0.7575 (standard deviation = 0.1978).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“‘Clade 6’ comprises the majority of the subsections I to III cyanobacteria (except marine picocyanobacteria, hot spring Synechococcus and early‐branching multicellular taxa) and is well supported in the phylogenomic tree, but not resolved in the ribosomal tree (BS: 41%).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“For the cyanobacterial stem lineage (calibration 1; Fig. 4), posterior age estimates were almost uniformly distributed in Hypothesis 1 and shifted towards an origin of cyanobacteria prior 3.5 Ga for Hypothesis 2.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Across the phylogeny, multicellularity is subsequently lost at least five times and regained on one, possibly two, branch leading to Leptolyngbya sp. PCC 7376 and Spirulina subsalsa PCC 9445.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“While 100% maximum likelihood bootstrap (BS) values supported just 24 of 64 branches of the ribosomal tree, 100% bootstrap support was inferred for 57 of 64 branches of the genomic tree.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Comparison of phylogenetic reconstructions based on genome and ribosomal data
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“In this study, the use of an impressively large data set (197 766 amino acid sites) helped to overcome the limitations previous analyses might have had, not only substantially improving the statistical support across cyanobacterial phylogeny in comparison with single‐gene analyses, but also corroborating the hypotheses of an early origin of multicellularity in Cyanobacteria (Schirrmeister et al. 2”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Schirrmeister et al. 2011b, 2013
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Our results show that multicellularity evolved very early among cyanobacteria and divergence time estimations (Fig. 5) confirm previous suggestions of an origin of multicellularity prior to the GOE, independently of whether the 2.0 Ga fossil akinete calibration is used.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“In addition to their ecological variety, cyanobacteria exhibit impressive morphological diversity, particularly for prokaryotes. On this basis, cyanobacteria have been classified and divided into five subsections (Rippka et al. 1979; Castenholz 2001).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Rippka et al. 1979
- Not checked yetcites Castenholz 2001
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The transition to multicellularity with its increase in overall size could have had a similar effect in cyanobacteria.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“These hypotheses, however, ignore the possibility of evolutionary innovations that could have influenced fitness and, hence, abundance of cyanobacteria.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Multicellularity, as a major evolutionary innovation, forming a novel unit for selection to act upon, may have served to overcome evolutionary constraints and enabled diversification of the variety of morphotypes seen in cyanobacteria today.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Difficulties in obtaining accurate age estimates for such deep speciation events may include: (1) the lack of evolutionary information retained in molecular data over such long timescales; (2) weaknesses in the phylogenetic model to correctly infer evolutionary processes that took place over such long time periods; and (3) the paucity of calibration points for divergence time estimation.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Further difficulties of calibrations involve: (1) the potential for their misassignment to clades; and (2) the likelihood that the age of the calibrating fossils is a poor approximation of their clade age.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Although the limiting factor on precision in divergence time studies is invariably the uncertainty associated with the fossil calibrations (dos Reis and Yang 2013), in terms of the degree to which fossil minima approximate the true time of divergence, much of the uncertainty associated with phylogeny and divergence time estimation can be diminished by employing genome scale data (dos Reis et al. 2”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites dos Reis and Yang 2013
- Not checked yetcites dos Reis et al. 2012
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Although many multicellular fossil remains from the Archean and Proterozoic (Altermann and Schopf 1995; Schopf 2006) have been interpreted as cyanobacteria, the overall fossil record is patchy at best and provides only glimpses into the history of these early prokaryotes.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Altermann and Schopf 1995
- Not checked yetcites Schopf 2006
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“The appearance of cyanobacterial fossils attributed to subsections IV and V cyanobacteria occurs after the GOE, supporting the hypothesis that heterocyst formation evolved after the increase in atmospheric oxygen to allow for nitrogen fixation, spatially separated from photosynthesis (Tomitani et al. 2006).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Tomitani et al. 2006
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“bacteria in subsections IV and V have the ability to form differentiated cells, such as metabolically specialized heterocysts for nitrogen fixation and resting cells, so called akinetes (Flores and Herrero 2010).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Flores and Herrero 2010
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
None of the sources cited for this claim have been checked yet.
In the paper
“Taxa belonging to subsection V are the only cyanobacteria that grow multiseriate filaments (varying cell width) and in several planes exhibit ‘true’ branching, not to be confused with ‘false’ branching (Rippka et al. 1979; Gugger and Hoffmann 2004).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Rippka et al. 1979
- Not checked yetcites Gugger and Hoffmann 2004
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Cyanobacteria are among the most ancient of evolutionary lineages, oxygenic photosynthesizers that may have originated before 3.0 Ga, as evidenced by free oxygen levels.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Abstract
What the sources say
- Not checked yetcites Crowe et al. 2013
- Not checked yetcites Lyons et al. 2014
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“Age ranges of specified and effective priors were similar, however, and could be accepted for the divergence time analyses.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“For all analyses, accepted changes to the chains had values of approximately 30% at the time of convergence.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
In the paper
“Based on Sm‐Nd isotopes, two kerogen‐rich shale samples of the Franceville Group were dated 2.099 Ga ± 115 Myr to 2.036 Ga ± 79 Myr, which suggests a conservative minimum constrain for the tree calibration of 1.957 Ga (Bros et al. 1992).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of terminal cell differentiation (calibration 2)
What the sources say
- Not checked yetcites Bros et al. 1992
hedgedcorrelationaln = 2- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“For analyses B and D, the lower limit on the age of crown Cyanobacteria is based on the estimated beginning of the GOE (Bekker et al. 2004).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
What the sources say
- Not checked yetcites Bekker et al. 2004
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“All MCMC runs exhibited evidence of sufficient mixing.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim.
None of the sources cited for this claim have been checked yet.
In the paper
“These fossil akinetes, classified as Archaeoellipsoides, have been reported from various intervals through the Proterozoic (Horodyski and Donaldson 1980; Golubic et al. 1995; Srivastava 2005); however, the microfossils of the Franceville Group are the earliest of these occurrences.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of terminal cell differentiation (calibration 2)
What the sources say
- Not checked yetcites Horodyski and Donaldson 1980
- Not checked yetcites Golubic et al. 1995
- Not checked yetcites Srivastava 2005
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“The lower limit on the age of crown Cyanobacteria in analyses A and C is based on Mo isotope evidence for oxygen production from the Sinqeni Fm., Pongola Supergroup, South Africa, indicating indirectly the presence of manganese oxidation, a process that would require abundant free oxygen (Planavsky et al. 2014).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
What the sources say
- Not checked yetcites Planavsky et al. 2014
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Applying 16S rRNA sequence data and a set of different calibration assumptions, a previous study by Schirrmeister et al. (2013) estimated divergence times that pointed towards an origin of cyanobacteria in the Archean Eon, with multicellularity more likely originating before the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Schirrmeister et al. (2013)
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. It may state two separate claims as one.
In the paper
“Previous hypotheses have argued for an origin of Cyanobacteria shortly before the GOE (Kirschvink and Kopp 2008), followed by a rapid accumulation of oxygen as observed during the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Kirschvink and Kopp 2008
plaindirect- Asserted: fails — The authors may not put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The authors may not put it forward as true. The paper’s conclusions may not depend on it. It may state two separate claims as one.
In the paper
“More than 2.83‐Gyr‐old reef systems from Mushandike, Zimbabwe, and Steep Rock, Canada, seem to have been formed in oxic waters and support the hypotheses of Archean oxygen oases that were based on the absence of mass‐independent sulphur fractionation (Ohmoto et al. 2006).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Ohmoto et al. 2006
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“it comprises merely 1400 nucleotide sites with only half of them susceptible to change in phylum Cyanobacteria.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Additionally, calibrations of tip clades have been claimed to be unsuitable for the accurate estimation of deep divergence events (Duchene et al. 2014).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Duchene et al. 2014
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
None of the sources cited for this claim have been checked yet.
In the paper
“Alternatively, several studies have found evidence of free oxygen and, thus, inferred the presence of cyanobacteria, hundreds of millions of years prior to the GOE, possibly as early as 3.0 Ga (Nisbet et al. 2007; Nisbet and Nisbet 2008; Crowe et al. 2013; Lyons et al. 2014).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Nisbet et al. 2007
- Not checked yetcites Nisbet and Nisbet 2008
- Not checked yetcites Crowe et al. 2013
hedgedcorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
In the paper
“Another study by Shih and Matzke (2013) recovered a much more recent origin of living cyanobacterial taxa concluding that an ancient cyanobacterial stem lineage must be responsible for late Archean oxygen levels.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Shih and Matzke (2013)
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Isotopes from organic carbon in these rocks, additionally, point towards cyanobacterial RuBisCO I activity in those deposits and support an origin of cyanobacteria in the Archean (Nisbet et al. 2007; Nisbet and Fowler 2011).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
What the sources say
- Not checked yetcites Nisbet et al. 2007
- Not checked yetcites Nisbet and Fowler 2011
plaincorrelational- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“The ATPase subunits resulted from an ancient duplication event, which occurred before the last common ancestor of all living taxa and has therefore been used in the past to reconstruct the Tree of Life (Iwabe et al. 1989).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
What the sources say
- Not checked yetcites Iwabe et al. 1989
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The assumptions that: (1) simple filamentous cyanobacterial taxa were present in 2.0‐Gyr‐old deposits; and (2) cyanobacteria were responsible for the accumulation of oxygen during the Archean, indicates an existence of multicellular cyanobacteria before the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
It may state two separate claims as one.
- The authors state this as an assumption: Simple filamentous cyanobacterial taxa were present in 2.0-Gyr-old deposits.
- The authors state this as an assumption: Cyanobacteria were responsible for the accumulation of oxygen during the Archean.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Microfossils from Proterozoic and Archean deposits comprise multicellular forms, such as septate and non‐septate filaments, and unicellular remains, such as spheres and rods.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We suggest that the origin of multicellularity was a major transition in the history of cyanobacteria, forming new units to be subject to selection, and offering the potential to increase cyanobacterial abundance, consequently initiating the GOE.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgeddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Furthermore, experiments have demonstrated the movement of filamentous cyanobacteria to avoid UV light, where prevention of movement resulted in UV‐induced inhibition of photosynthesis (Kruschel and Castenholz 1998).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Kruschel and Castenholz 1998
boosteddirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“In Archean environments, Fe (II) toxicity could have prohibited oxygenic photosynthesis and subsequently allowed for only little oxygen production.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“The delay in the accumulation of free oxygen until the GOE has been explained by a strongly reducing atmosphere where initially produced oxygen was captured by oxygen sinks, such as reduced volcanic gases (Catling and Claire 2005).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
What the sources say
- Not checked yetcites Catling and Claire 2005
plaindirect- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Furthermore, multicellularity could have provided novel possibilities for cyanobacterial diversification and adaptation to new oxygenated habitats.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“As the only biological source of oxygen during the early Precambrian, cyanobacterial fitness and ecological success should have had a profound impact on the amount of free net oxygen in Earth's ocean and atmosphere.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Comparisons of modern cyanobacterial taxa to Precambrian microfossils support the inferred presence of multicellular cyanobacteria before the GOE, but the fossil record does not provide evidence for multicellular taxa among the earliest unequivocal fossil assemblages at 3.33–3.45 Ga.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Conclusion
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Multicellularity provides selective advantage during early Earth history including: (1) movement within microbial mats to avoid lethal UV‐C dosages; and (2) improved attachment to surfaces during initial mat formation that may have substantially increased the success of cyanobacterial‐dominated mat communities and enabled adaptation to novel habitats.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Conclusion
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: unclear — It is unclear why the paper says it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Similarly, increased sizes of multicellular cyanobacteria may have resulted in higher metabolic rates, hence, higher photosynthetic activity and increased net oxygen production.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds. It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Additionally, multicellular growth may have provided competitive advantages that resulted in a higher growth success (Fig. 6).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Benefits of cyanobacterial multicellularity and its potential consequences for the GOE
hedgedconditional- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Cyanobacteria originated in the mid‐Archean, long before the GOE, with multicellular taxa evolving towards the end of the Archean.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Conclusion
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
The authors state this as an assumption.
The divergence of the Gloeobacter lineage from the stem lineage leading to all other extant cyanobacteria occurred between 3.85 and 2.918 Ga (analyses A, C) or between 3.85 and 2.45 Ga (analyses B, D).
“The divergence of Gloeobacter lineage from the stem lineage leading to the all other extant cyanobacterial species was assumed to have occurred some time between 3.85 and 2.918 Ga (Table 1, analyses A, C) or 3.85 and 2.45 Ga (Table 1, analyses B, D), with each time point being equally likely (uniform prior distribution).”
The authors state this as an assumption.
The most recent common ancestor of subsections IV and V cyanobacteria originated after the GOE but before 1.957 Ga.
“we assumed that the most recent common ancestor of subsections IV and V cyanobacteria must have originated after the GOE, but prior to 1.957 Ga.”
The authors state this as an assumption.
The end of the Late Heavy Bombardment at 3.85 Ga can be taken as a similar age for Earth.
“Given that the heavy lunar bombardment is estimated to have ended at 3.85 Ga, a similar age may be assumed for Earth given the proximity of the moon.”
The authors state this as an assumption.
Simple filamentous cyanobacterial taxa were present in 2.0-Gyr-old deposits.
“The assumptions that: (1) simple filamentous cyanobacterial taxa were present in 2.0‐Gyr‐old deposits; and (2) cyanobacteria were responsible for the accumulation of oxygen during the Archean, indicates an existence of multicellular cyanobacteria before the GOE.”
The authors state this as an assumption.
Cyanobacteria were responsible for the accumulation of oxygen during the Archean.
“The assumptions that: (1) simple filamentous cyanobacterial taxa were present in 2.0‐Gyr‐old deposits; and (2) cyanobacteria were responsible for the accumulation of oxygen during the Archean, indicates an existence of multicellular cyanobacteria before the GOE.”
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
The cited source says what the claim attributes to it.
In the citing paper
“For example, cyanobacteria probably evolved [e.g., (3)] during this period”
From The Archean atmosphere (2020) · cites this paper as [3]
The cited source says what the claim attributes to it.
In the citing paper
“While some argue that oxygenic photosynthesis evolved only 50 to 100 Ma before the GOE (115), most studies suggest an earlier Paleoarchean or Mesoarchean age [e.g., (3, 118, 119)].”
From The Archean atmosphere (2020) · cites this paper as [3]
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
Each contradiction between two passages listed here was confirmed by an independent check.
Rated major: it would touch a result — a value a result rests on, reported and recomputed p-values on opposite sides of the significance level, two passages that conflict with no sign which is right, or a cited work retracted before this paper was published.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of terminal cell differentiation (calibration 2)
“We assumed a uniform prior calibration density between 1.957 and 2.45 Ga with 5% prior probability that posterior estimates may lie outside this interval (soft bounds).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Divergence time estimation and calibration
“| A, C | Section IV and V | Uniform (sb) | 1.957 | 2.32 | 1.957 | 2.32 |”
Rated major: it would touch a result — a value a result rests on, reported and recomputed p-values on opposite sides of the significance level, two passages that conflict with no sign which is right, or a cited work retracted before this paper was published.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Restricting the origin of cyanobacteria (calibration 1)
“The divergence of Gloeobacter lineage from the stem lineage leading to the all other extant cyanobacterial species was assumed to have occurred some time between 3.85 and 2.918 Ga (Table 1, analyses A, C) or 3.85 and 2.45 Ga (Table 1, analyses B, D)”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Divergence time estimation and calibration
“| A, C | Root | Uniform (hb) | 2.45 | 3.85 | 2.45 | 3.85 |”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Improved data set to reconstruct the evolutionary history of Cyanobacteria
“an impressively large data set (197 766 amino acid sites)”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Phylogenomic analyses using a supermatrix
“the resultant 197 761 amino acid‐rich supermatrix”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Taxon sampling
“and five multicellular strains belonging to the filamentous cyanobacteria without cellular differentiation”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Taxon sampling
“(1) Geitlerinema sp. PCC 8501; (2) Leptolyngbya sp. PCC 73110; (3) Limnothrix redekei PCC 9416; (4) Pseudanabaena sp. PCC 7704 and PCC 7904; and (5) Symploca sp. PCC 8002)”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
“a narrower root calibration (3.85–2.958 Ga)”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Divergence time estimation and calibration
“| B, D | Root | Uniform (hb) | 2.918 | 3.85 | 2.918 | 3.85 |”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Ancestral character state reconstruction
“where q01 defines the transition to multicellularity and q01 the loss of multicellularity.”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > Ancestral character state reconstruction
“q01 describes the transition to multicellularity and q10 the transition to unicellularity.”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Discussion > Comparison of cyanobacterial cell sizes to Precambrian microfossils
“In c. 2.0 Ma deposits from Western Australia, filaments of large size (63 μm in width) have been found and classified as Oscillatoriopsis majuscule (Knoll et al. 1988).”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > The evolution of multicellularity – testing two hypotheses (calibration 3)
“Deposits of similar age from the Duck Creek Dolomite in Western Australia (c. 2.0 Ga) contain several fossils similar to the multicellular cyanobacterial genus Lyngbya, named Oscillatoriopsis (Knoll et al. 1988).”
Rated minor: it would not touch a result — a value no result rests on, a p-value that stays on the same side of the significance level, or a conflict that is clerical, resolved elsewhere in the paper, or outside its own findings.
In the paper
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Material and methods > The evolution of multicellularity – testing two hypotheses (calibration 3)
“Hypothesis 1: Multicellularity originated in cyanobacteria before the Great Oxidation Event (GOE)”
§ Cyanobacteria and the Great Oxidation Event: evidence from genes and fossils > Results > Divergence time estimation
“an origin of multicellularity after the GOE as an adaptation to newly formed (oxygenated) habitats (Hypothesis 1); or (2) an origin of multicellularity before the GOE”
Citations
Cites
1 retracted
Westall, F., de Ronde, C. E. J., Southam, G., Grassineau, N. V., Colas, M., Cockell, C. S., & Lammer, H. (2006) · Philosophical Transactions of the Royal Society B Biological Sciences · doi:10.1098/rstb.2006.1896 · Cited by 203
RetractedMAFFT Multiple Sequence Alignment Software Version 7: Improvements in Performance and Usability
Katoh, K., & Standley, D. M. (2013) · Molecular Biology and Evolution · doi:10.1093/molbev/mst010 · Cited by 46,209
BLAST+: architecture and applications
Camacho, C., Coulouris, G., Avagyan, V., Ma, N., Papadopoulos, J., Bealer, K., & Madden, T. L. (2009) · BMC Bioinformatics · doi:10.1186/1471-2105-10-421 · Cited by 22,074
Prokka: rapid prokaryotic genome annotation
Seemann, T. (2014) · Bioinformatics · doi:10.1093/bioinformatics/btu153 · Cited by 18,937
PAML 4: Phylogenetic Analysis by Maximum Likelihood
Yang, Z. (2007) · Molecular Biology and Evolution · doi:10.1093/molbev/msm088 · Cited by 13,879
APE: analyses of phylogenetics and evolution in R language
Paradis, E., Claude, J., & Strimmer, K. (2004) · Bioinformatics · doi:10.1093/bioinformatics/btg412 · Cited by 11,335
Velvet: Algorithms for de novo short read assembly using de Bruijn graphsPreprint
Zerbino, D. R., & Birney, E. (2008) · Genome Research · doi:10.1101/gr.074492.107 · Cited by 9,587
EMBOSS: the European molecular biology open software suite.
Rice, P., Longden, I., & Bleasby, A. (2000) · Trends in Genetics · doi:10.1016/s0168-9525(00)02024-2 · Cited by 9,466
Generic Assignments, Strain Histories and Properties of Pure Cultures of Cyanobacteria
Rippka, R., Stanier, R. Y., Deruelles, J., Herdman, M., & Waterbury, J. B. (1979) · Microbiology · doi:10.1099/00221287-111-1-1 · Cited by 7,606
Relaxed Phylogenetics and Dating with Confidence
Drummond, A. J., Ho, S. Y. W., Phillips, M. J., & Rambaut, A. (2006) · PLoS Biology · doi:10.1371/journal.pbio.0040088 · Cited by 6,463
Cited by
Sorted by citations
Huisman, J., Codd, G. A., Paerl, H. W., Ibelings, B. W., Verspagen, J. M. H., & Visser, P. (2018) · Nature Reviews Microbiology · doi:10.1038/s41579-018-0040-1 · Cited by 2,935
Catling, D. C., & Zahnle, K. J. (2020) · Science Advances · doi:10.1126/sciadv.aax1420 · Cited by 568
Early photosynthetic eukaryotes inhabited low-salinity habitats
Sánchez‐Baracaldo, P., Raven, J. A., Pisani, D., & Knoll, A. H. (2017) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1620089114 · Cited by 332
On the origin of oxygenic photosynthesis and Cyanobacteria
Sánchez‐Baracaldo, P., & Cardona, T. (2019) · New Phytologist · doi:10.1111/nph.16249 · Cited by 290
“Furthermore, the standard heterodimeric photosystems, a defining 87 trait of crown group Cyanobacteria (Figure 3), evolved towards the late Archean (Blank & 88 Sánchez-Baracaldo, 2010; Schirrmeister et al., 2015) or early Paleoproterozoic (Shih et al., 89 2016).”
BackgroundMethodInfluentialCyanobacteria and biogeochemical cycles through Earth history
Sánchez-Baracaldo, P., Bianchini, G., Wilson, J. D., & Knoll, A. H. (2022) · Trends in Microbiology · doi:10.1016/j.tim.2021.05.008 · Cited by 279
Metadata
- Authors
- Schirrmeister, B. E., Gugger, M., & Donoghue, P. C. J.
- Affiliations
- University of Bristol (GB)
- Institut Pasteur (FR)
- Venue
- Palaeontology
- Publisher
- Wiley
- Published
- 2015-06-23
- Volume
- 58
- Issue
- 5
- Pages
- 769-785
- ISSN
- 0031-0239 (ISSN-L)
- 1475-4983
- PMC
- PMC4755140
- OpenAlex
- W1831957949
- Semantic Scholar
- 6e03cd37924a78a193bde6f1580e42699eee46c3
- Cited by
- 304
- References
- 102
- Citations by year
- 2026: 24 · 2025: 29 · 2024: 54 · 2023: 31 · 2022: 30 · 2021: 25 · 2020: 21 · 2019: 32 · 2018: 28 · 2017: 18 · 2016: 8 · 2015: 4
- FWCI
- 8.40
- Type
- journal article
- Language
- en
- Update notices
- correction (2015-08-14)
- Open access
- hybrid
- doi.org
- Licence
- Locations
- Palaeontology (publishedVersion, cc-by)
- Europe PMC (PubMed Central) (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- Explore Bristol Research (publishedVersion, cc-by)
- HAL (submittedVersion, cc-by)
- Bristol Research (University of Bristol) (submittedVersion, cc-by)
- Funders
- Biotechnology and Biological Sciences Research Council (BB/J00538X/1)
- European Commission (FP7 - PEOPLE - 2012 - IEF) (PIEF-GA-2012-330849)
- Swiss National Science Foundation (PBZHP3_147232)
- Topics
- Life Sciences › Agricultural and Biological Sciences › Ecology, Evolution, Behavior and Systematics › Protist diversity and phylogeny
- Physical Sciences › Earth and Planetary Sciences › Paleontology › Paleontology and Stratigraphy of Fossils
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Photosynthetic Processes and Mechanisms
- Keywords
- cyanobacteria, Great Oxidation Event, multicellularity, cyanobacterial evolution, Archean, phylogenomics, character reconstruction, cyanobacterial genome, cyanobacterial diversity
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
A language model drew the claims from the paper on 2026-10-08, under version 3 of the claim definition (model deepseek-v4.1-flash, prompt extract-v3).
A second model labelled each claim on 2026-10-08 (model jev-1.13-20260917, definition revision gold-guideline-v0.2).
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
