

The DOI matches its Crossref record; 1 of the 1 references it cites were found in a registry or an index.
Rifampin resistance and its fitness cost in Riemerella anatipestifer
Open accessAbstract
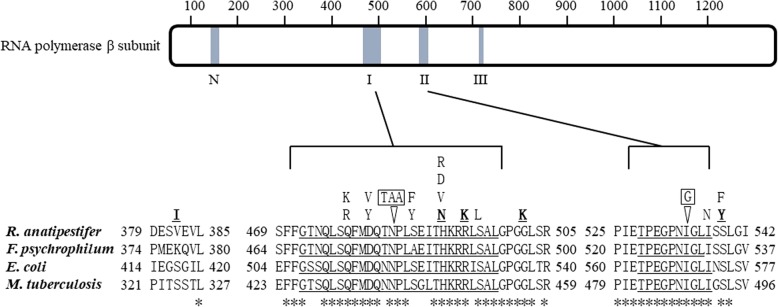
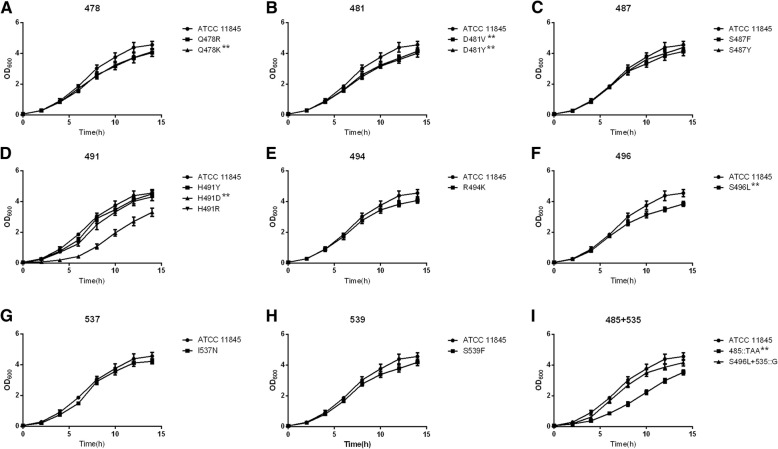
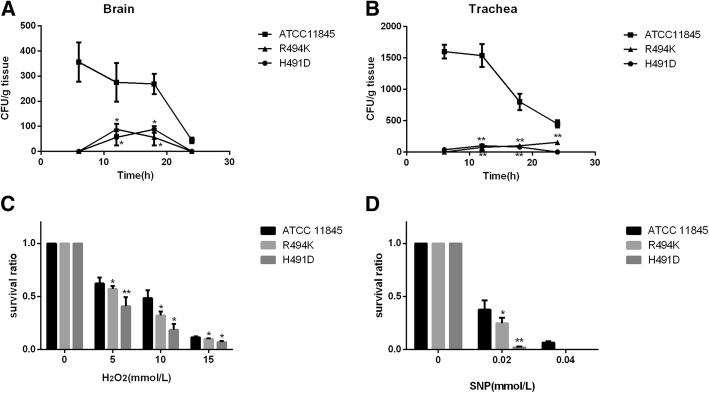
Riemerella anatipestifer ( R. anatipestifer ) is one of the most important poultry pathogens worldwide, with associated infections causing significant economic losses. Rifampin Resistance is an important mechanism of drug resistance. However, there is no information about rpoB mutations conferring rifampin resistance and its fitness cost in Riemerella anatipestifer . Comparative analysis of 18 R.anatipestifer rpoB sequences and the determination of rifampin minimum inhibitory concentrations showed that five point mutations, V382I, H491N, G502K, R494K and S539Y, were related to rifampin resistance. Five overexpression strains were constructed using site-directed mutagenesis to validate these sites. To investigate the origin and fitness costs of the rpoB mutations, 15 types of rpoB mutations were isolated from R. anatipestifer ATCC 11845 by using spontaneous mutation in which R494K was identical to the type of mutation detected in the isolates. The mutation frequency of the rpoB gene was calculated to be 10 − 8 . A total of 98.8% (247/250) of the obtained mutants were located in cluster I of the rifampin resistance-determining region of the rpoB gene. With the exception of D481Y, I537N and S539F, the rifampin minimum inhibitory concentrations of the remaining mutants were at least 64 μg/mL. The growth performance and competitive experiments of the mutant strains in vitro showed that H491D and 485::TAA exhibit growth delay and severely impaired fitness. Finally, the colonization abilities and sensitivities of the R494K and H491D mutants were investigated. The sensitivity of the two mutants to hydrogen peroxide (H 2 O 2) and sodium nitroprusside (SNP) increased compared to the parental strain. The number of live colonies colonized by the two mutants in the duckling brain and trachea were lower than that of the parental strain within 24 h. Mutations of rpoB gene in R. anatipestifer mediate rifampin resistance and result in fitness costs. And different single mutations confer different levels of fitness costs. Our study provides, to our knowledge, the first estimates of the fitness cost associated with the R. anatipestifer rifampin resistance in vitro and in vivo .
Overview
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
The check wasn’t confident either way, so it gives no verdict — never disputed.
In the citing paper
“Recently there has been evidence that a big role in phenotypic delay may be played by chromosome segregation in quickly dividing cells [21,58].”
From Efficient, robust, and versatile fluctuation data analysis using MLE MUtation Rate calculator (mlemur) (2023) · cites this paper as [58]
Experimental — accuracy not yet measured
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
Structural Mechanism for Rifampicin Inhibition of Bacterial RNA Polymerase
Campbell, E. A., Korzheva, N., Mustaev, A., Murakami, K., Nair, S., Goldfarb, A., & Darst, S. A. (2001) · Cell · doi:10.1016/s0092-8674(01)00286-0 · Cited by 1,556 · cited 1×
“It can only block transcription initiation and did not inhibit the extension process [6].”
Background
Research works printed but not linked: 38
- Ruiz JA, Sandhu TS. Riemerella anatipestifer infection. In: Swayne DE, Glisson JR, McDougald LR, Nolan LK, Suarez DL, Nair VL, editors. Diseases of poultry. 13th ed. Hoboken: John Wiley & Sons, Inc.; 2013. p. 823–8.
- Tan Y, Hu Z, Zhao Y, Cai X, Luo C, Zou C, Liu X. The beginning of the rpoB gene in addition to the rifampin resistance determination region might be needed for identifying rifampin/rifabutin cross-resistance in multidrug-resistant Mycobacterium tuberculosis isolates from southern China. J Clin Microbiol. 2012;50(1):81–5. https://doi.org/10.1128/JCM05092-11 . · DOI
- Jin DJ, Gross CA. Mapping and sequencing of mutations in the Escherichia coli rpoB gene that lead to rifampicin resistance. J Mol Biol. 1988;202(1):45–58. https://doi.org/10.1016/0022-2836(88)90517-7 . · DOI
- Landick R, Stewart J, Lee DN. Amino acid changes in conserved regions of the beta-subunit of Escherichia coli RNA polymerase alter transcription pausing and termination. Genes Dev. 1990;4(9):1623. https://doi.org/10.1101/gad.4.9.1623 . · DOI
- Heep M, Brandstatter B, Rieger U, Lehn N, Richter E, Rusch-Gerdes S, Niemann S. Frequency of rpoB mutations inside and outside the cluster I region in rifampin-resistant clinical Mycobacterium tuberculosis isolates. J Clin Microbiol. 2001;39(1):107–10. https://doi.org/10.1128/JCM.39.1.107-110.2001 . · DOI
- Borukhov S, Nudler E. RNA polymerase holoenzyme: structure, function and biological implications. Curr Opin Microbiol. 2003;6(2):93–100. https://doi.org/10.1016/S1369-5274(03)00036-5 . · DOI
- Pang Y, Lu J, Wang Y, Song Y, Wang S, Zhao Y. Study of the rifampin monoresistance mechanism in Mycobacterium tuberculosis. Antimicrob Agents Chemother. 2013;57(2):893–900. https://doi.org/10.1128/AAC.01024-12 . · DOI
- Andersson DI, Levin BR. The biological cost of antibiotic resistance. Curr Opin Microbiol. 1999;2(5):489–93. https://doi.org/10.1016/S1369-5274(99)00005-3 . · DOI
- Billington OJ, Mchugh TD, Gillespie SH. Physiological cost of rifampin resistance induced in vitro in Mycobacterium tuberculosis. Antimicrob Agents Chemother. 1999;43(8):1866–9. · DOI
- Sander P, Springer B, Prammananan T, Sturmfels A, Kappler M, Pletschette M, Bottger EC. Fitness cost of chromosomal drug resistance-conferring mutations. Antimicrob Agents Chemother. 2002;46(5):1204–11. https://doi.org/10.1128/AAC.46.5.1204-1211.2002 . · DOI
- Colicchio R, Pagliuca C, Pastore G, Cicatiello AG, Pagliarulo C, Tala A, Scaglione E, Sammartino JC, Bucci C, Alifano P, et al. Fitness cost of rifampin resistance in Neisseria meningitidis: In vitro study of mechanisms associated with rpoB H553Y mutation. Antimicrob Agents Chemother. 2015;59(12):7637–49. https://doi.org/10.1128/AAC.01746-15 . · DOI
- Huang L, Yuan H, Liu MF, Zhao XX, Wang MS, Jia RY, Chen S, Sun KF, Yang Q, Wu Y, et al. Type B chloramphenicol acetyltransferases are responsible for chloramphenicol resistance in Riemerella anatipestifer, China. Front Microbiol. 2017;8:297. https://doi.org/10.3389/fmicb.2017.00297 . · DOI
- Luo HY, Liu MF, Wang MS, Zhao XX, Jia RY, Chen S, Sun KF, Yang Q, Wu Y, Chen XY, et al. A novel resistance gene, lnu(H), conferring resistance to lincosamides in Riemerella anatipestifer CH-2. Int J Antimicrob Agents. 2017;51(1):136–9. https://doi.org/10.1016/j.ijantimicag.2017.08.022 . · DOI
- Zhang X, Wang MS, Liu MF, Zhu DK, Biville F, Jia RY, Chen S, Sun KF, Yang Q, Wu Y, et al. Contribution of RaeB, a putative RND-type transporter to aminoglycoside and detergent resistance in Riemerella anatipestifer. Front Microbiol. 2017;8:2435. https://doi.org/10.3389/fmicb.2017.02435 . · DOI
- Zhong CY, Cheng AC, Wang MS, Zhu DK, Luo QH, Zhong CD, Li L, Duan Z. Antibiotic susceptibility of Riemerella anatipestifer field isolates. Avian Dis. 2009;53:601–7 https://www.jstor.org/stable/25599169 . · DOI
- Klein JL, Brown TJ, French GL. Rifampin resistance in Mycobacterium kansasii is associated with rpoB mutations. Antimicrob Agents Chemother. 2001;45(11):3056–8. https://doi.org/10.1128/AAC.45.11.3056-3058.2001 . · DOI
- Dabbs ER, Yazawa K, Tanaka Y, Mikami Y, Miyaji M, Andersen SJ, Morisaki N, Iwasaki S, Shida O, Takagi H. Rifampicin inactivation by Bacillus species. J Antibiot. 1995;48(8):815–9. · DOI
- Imai T, Watanabe K, Mikami Y, Yazawa K, Ando A, Nagata Y, Morisaki N, Hashimoto Y, Furihata K, Dabbs ER. Identification and characterization of a new intermediate in the ribosylative inactivation pathway of rifampin by Mycobacterium smegmatis. Microb Drug Resist. 1999;5(4):259–64. https://doi.org/10.1089/mdr.1999.5.259 . · DOI
- Combrink KD, Denton DA, Harran S, Ma Z, Chapo K, Yan D, Bonventre E, Roche ED, Doyle TB, Robertson GT. New C25 carbamate rifamycin derivatives are resistant to inactivation by ADP-ribosyl transferases. Bioorg Med Chem Lett. 2007;17(2):522–6. https://doi.org/10.1016/j.bmcl.2006.10.016 . · DOI
- Artsimovitch I, Vassylyeva MN, Svetlov D, Svetlov V, Perederina A, Igarashi N, Matsugaki N, Wakatsuki S, Tahirov TH, Vassylyev DG. Allosteric modulation of the RNA polymerase catalytic reaction is an essential component of transcription control by rifamycins. Cell. 2005;122(3):351–63. https://doi.org/10.1016/j.cell.2005.07.014 . · DOI
- Cavusoglu C, Karacaderici Y, Bilgic A. In-vitro activity of rifabutin against rifampicin-resistant Mycobacterium tuberculosis isolates with known rpoB mutations. Clin Microbiol Infect. 2004;10(7):662–5. https://doi.org/10.1111/j.1469-0691.2004.00917.x . · DOI
- Figueiredo R, Ramos DF, Moiteiro C, Medeiros MA, Curto MJM, Menezes JCD, Pando RH, Silva PEA, Costa MDC. Pharmacophore insights into rpoB gene mutations in Mycobacterium tuberculosis rifampicin resistant isolates. Eur J Med Chem. 2012;47(1):186–93. https://doi.org/10.1016/j.ejmech.2011.10.041 . · DOI
- Brandis G, Pietsch F, Alemayehu R, Hughes D. Comprehensive phenotypic characterization of rifampicin resistance mutations in Salmonella provides insight into the evolution of resistance in Mycobacterium tuberculosis. J Antimicrob Chemother. 2014;70(3):680–5. https://doi.org/10.1093/jac/dku434 . · DOI
- Vigliotta G, Tredici SM, Damiano F, Montinaro MR, Pulimeno R, Di SR, Rita MD, GG V, Alifano P. Natural merodiploidy involving duplicated rpoB alleles affects secondary metabolism in a producer actinomycete. Mol Microbiol. 2005;55(2):396–412. https://doi.org/10.1111/j.1365-2958.2004.04406.x . · DOI
- Vogwill T, Kojadinovic M, MacLean RC. Epistasis between antibiotic resistance mutations and genetic background shape the fitness effect of resistance across species of Pseudomonas. Proc R Soc B. 2016;283(1830):20160151. https://doi.org/10.1098/rspb.2016.0151 . · DOI
- Gifford DR, Toll-Riera M, MacLean RC. Environmental variation alters the fitness effects of rifampicin resistance mutations in Pseudomonas aeruginosa. Evolution. 2016;70(3):725–30. https://doi.org/10.1111/evo.12958. · DOI
- Mejia YX, Mao H, Forde NR, Bustamante C. Thermal probing of E.coli RNA polymerase off-pathway mechanisms. J Mol Biol. 2008;382(3):628–37. https://doi.org/10.1016/j.jmb.2008.06.079 . · DOI
- Nicholson WL, Park R. Anaerobic growth of Bacillus subtilis alters the spectrum of spontaneous mutations in the rpoB gene leading to rifampicin resistance. FEMS Microbiol Lett. 2015;362(24):fnv213. https://doi.org/10.1093/femsle/fnv213 . · DOI
- Fajardocavazos P, Leehan JD, Nicholson WL. Alterations in the Spectrum of spontaneous rifampicin-resistance mutations in the Bacillus subtilis rpoB gene after cultivation in the human spaceflight environment. Front Microbiol. 2018;9. https://doi.org/10.3389/fmicb.2018.00192 . · DOI
- Gliniewicz K, Wildung M, Orfe LH, Wiens GD, Cain KD, Lahmers KK, Snekvik KR, Call DR. Potential mechanisms of attenuation for rifampicin-passaged strains of Flavobacterium psychrophilum. BMC Microbiol. 2015;15(1):179. https://doi.org/10.1186/s12866-015-0518-1 . · DOI
- Gagneux S, Long CD, Small PM, Van T, Schoolnik GK. The competitive cost of antibiotic resistance in Mycobacterium tuberculosis. Science. 2006;312(5782):1944–6. https://doi.org/10.1126/science.1124410 . · DOI · Paper page
- Qi Q, Preston GM, MacLean RC. Linking system-wide impacts of RNA polymerase mutations to the fitness cost of rifampin resistance in Pseudomonas aeruginosa. MBio. 2014;5(6):e01562–14. https://doi.org/10.1128/mBio.01562-14 . · DOI
- Pérezvarela M, Corral J, Vallejo JA, Rumbofeal S, Bou G, Aranda J, Barbé J. Mutants in the β-subunit of the RNA polymerase impairing the surface-associated motility and virulence of Acinetobacter baumannii. Infect Immun. 2017;85(8):e00327–17. https://doi.org/10.1128/IAI.00327-17 . · DOI
- Meenakshi S, Munavar MH. Suppression of capsule expression in Deltalon strains of Escherichia coli by two novel rpoB mutations in concert with HNS: possible role for DNA bending at rcsA promoter. Microbiologyopen. 2015;4(5):712–29. https://doi.org/10.1002/mbo3.268 . · DOI
- Talà A, Monaco C, Nagorska K, Exley RM, Corbett A, Zychlinsky A, Alifano P, Tang CM. Glutamate utilization promotes meningococcal survival in vivo through avoidance of the neutrophil oxidative burst. Mol Microbiol. 2011;81(5):1330–42. https://doi.org/10.1111/j.1365-2958.2011.07766.x . · DOI
- Liu M, Wang M, Zhu D, Wang M, Jia R, Chen S, Sun K, Yang Q, Wu Y, Chen X, et al. Investigation of TbfA in Riemerella anatipestifer using plasmid-based methods for gene over-expression and knockdown. Sci Rep. 2016;6:37159. https://doi.org/10.1038/srep37159 . · DOI
- CLSI. Performance Standards for Antimicrobial Disk and Dilution Susceptibility Tests for Bacteria Isolated From Animals; Approved Standard—Fourth Edition. CLSI document VET01-A4. Wayne: Clinical and Laboratory Standards Institute; 2013.
- Liu M, Zhang L, Huang L, Biville F, Zhu D, Wang M, Jia R, Chen S, Sun K, Yang Q, et al. Use of natural transformation to establish an easy knockout method in Riemerella anatipestifer. Appl Environ Microbiol. 2017;83(9):e00127–17. https://doi.org/10.1128/AEM.00127-17 . · DOI
Cited by
Łazowski, K. (2023) · Mutation Research - Fundamental and Molecular Mechanisms of Mutagenesis · doi:10.1016/j.mrfmmm.2023.111816 · Cited by 9
Metadata
- Authors
- Sun, J., Zhu, D., Xu, J., Jia, R., Chen, S., Liu, M., Zhao, X., Yang, Q., Wu, Y., Zhang, S., Liu, Y., Zhang, L., Yu, Y., You, Y., Wang, M., & Cheng, A.
- Affiliations
- Sichuan Agricultural University (CN)
- Corresponding author
- Wang, Mingshu
- Cheng, Anchun
- ORCID
- Venue
- BMC Microbiology
- Published
- 2019-05-23
- Volume
- 19
- Issue
- 1
- Pages
- 107-107
- ISSN
- 1471-2180 (ISSN-L)
- PMC
- PMC6533769
- OpenAlex
- W2947557968
- Cited by
- 17
- References
- 1
- Citations by year
- 2025: 3 · 2024: 2 · 2023: 5 · 2022: 1 · 2021: 3 · 2020: 3
- FWCI
- 0.61
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Locations
- BMC Microbiology (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion, cc-by-sa)
- Funders
- National Key Research and Development Program of China (2017YFD050080)
- Agriculture Research System of China (CARS-42-17)
- International S&T Cooperation Program of Sichuan Province (2017HH0026)
- Special Fund for Key Laboratory of Animal Disease and Human Health of Sichuan Province (2016JPT0004)
- Science and Technology Innovation Program of Guizhou Academy of Agricultural Science ([2017]03)
- Topics
- Health Sciences › Medicine › Microbiology (medical) › Antibiotic Resistance in Bacteria
- Life Sciences › Immunology and Microbiology › Microbiology › Microbial infections and disease research
- Health Sciences › Medicine › Infectious Diseases › Antimicrobial Resistance in Staphylococcus
- Keywords
- resistance, Riemerella anatipestifer, rpoB mutations, fitness cost, drug resistance, minimum inhibitory concentration, spontaneous mutation, competitive fitness, colonization ability, hydrogen peroxide sensitivity, poultry pathogens
- MeSH terms
- Animals, Bacterial Proteins, Brain, Ducks, Hydrogen Peroxide, Microbial Sensitivity Tests, Nitroprusside, Rifampin, DNA-Directed RNA Polymerases, Trachea, Point Mutation, Drug Resistance, Bacterial, Riemerella
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
Data sources
Bibliographic data: Semantic Scholar, OpenAlex, Crossref.
Contains information from the Semantic Scholar Academic Graph Datasets, made available under the ODC Attribution License (ODC-BY 1.0).
Semantic Scholar’s data is described in: Kinney, R., et al. (2023). The Semantic Scholar Open Data Platform. arXiv:2301.10140.
