

The DOI matches its Crossref record; 57 of the 58 references it cites were found in a registry or an index.
Cereal Domestication and Evolution of Branching: Evidence for Soft Selection in the Tb1 Orthologue of Pearl Millet (Pennisetum glaucum [L.] R. Br.)
Open accessAbstract
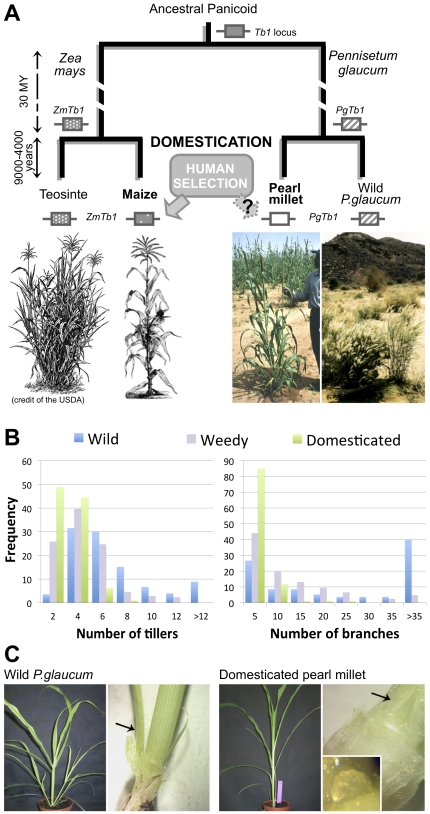
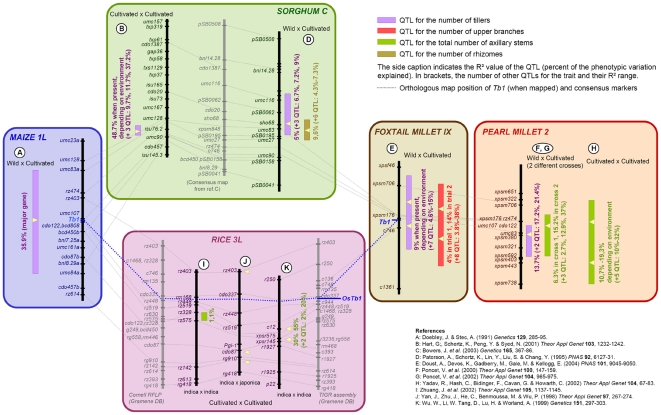
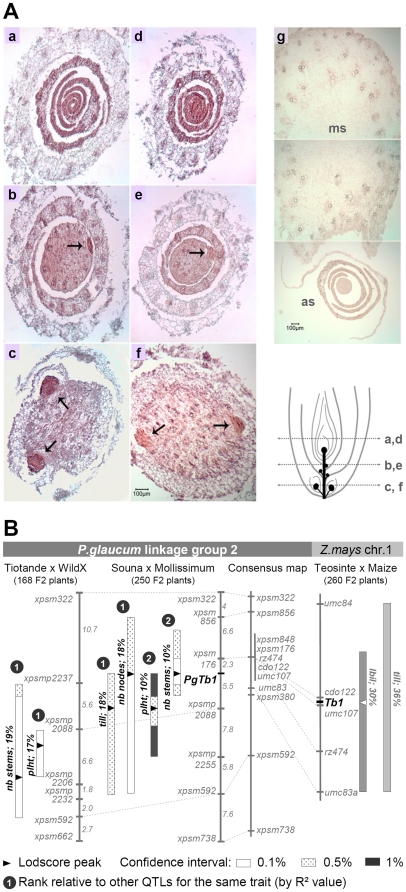
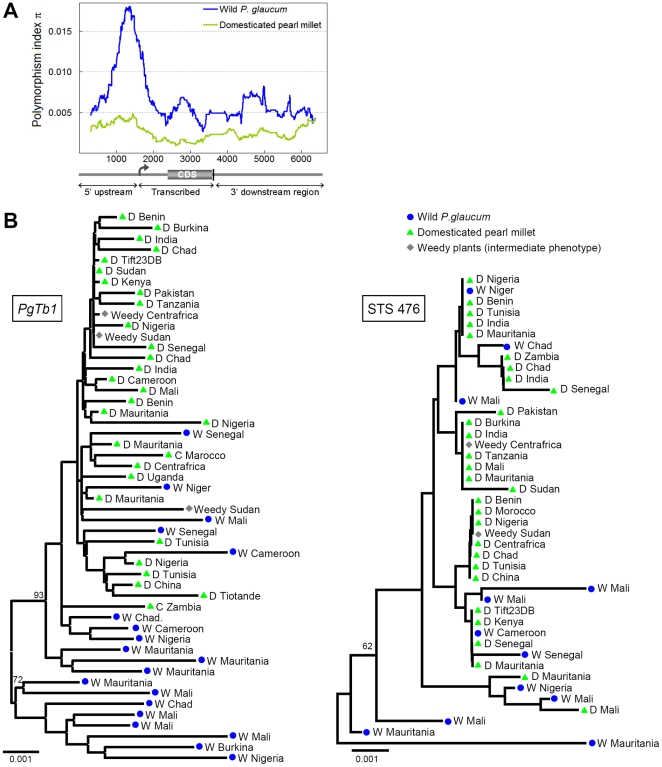
BACKGROUND: During the Neolithic revolution, early farmers altered plant development to domesticate crops. Similar traits were often selected independently in different wild species; yet the genetic basis of this parallel phenotypic evolution remains elusive. Plant architecture ranks among these target traits composing the domestication syndrome. We focused on the reduction of branching which occurred in several cereals, an adaptation known to rely on the major gene Teosinte-branched1 (Tb1) in maize. We investigate the role of the Tb1 orthologue (Pgtb1) in the domestication of pearl millet (Pennisetum glaucum), an African outcrossing cereal. METHODOLOGY/PRINCIPAL FINDINGS: Gene cloning, expression profiling, QTL mapping and molecular evolution analysis were combined in a comparative approach between pearl millet and maize. Our results in pearl millet support a role for PgTb1 in domestication despite important differences in the genetic basis of branching adaptation in that species compared to maize (e.g. weaker effects of PgTb1). Genetic maps suggest this pattern to be consistent in other cereals with reduced branching (e.g. sorghum, foxtail millet). Moreover, although the adaptive sites underlying domestication were not formerly identified, signatures of selection pointed to putative regulatory regions upstream of both Tb1 orthologues in maize and pearl millet. However, the signature of human selection in the pearl millet Tb1 is much weaker in pearl millet than in maize. CONCLUSIONS/SIGNIFICANCE: Our results suggest that some level of parallel evolution involved at least regions directly upstream of Tb1 for the domestication of pearl millet and maize. This was unanticipated given the multigenic basis of domestication traits and the divergence of wild progenitor species for over 30 million years prior to human selection. We also hypothesized that regular introgression of domestic pearl millet phenotypes by genes from the wild gene pool could explain why the selective sweep in pearl millet is softer than in maize.
Overview
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
The source backs part of the claim, not all of it — or backs it for a different population, condition or comparison.
In the citing paper
“This analysis indicates that nucleotide changes important for the reduced branching of pearl millet occurred within the promoter region of the TB1 gene (Remigereau et al., 2011).”
From Shaping plant architecture (2015) · cites this paper as Remigereau et al., 2011
Experimental — accuracy not yet measuredThe source backs part of the claim, not all of it — or backs it for a different population, condition or comparison.
In the citing paper
“Interestingly, comparative QTL mapping revealed that also in pearl millet, TB1 was the molecular target of domestication (Remigereau et al., 2011).”
From Shaping plant architecture (2015) · cites this paper as Remigereau et al., 2011
Experimental — accuracy not yet measuredThe cited source says what the claim attributes to it.
In the citing paper
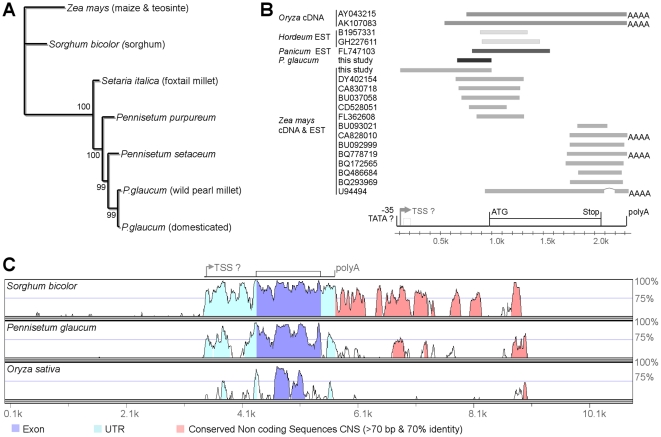
“Polymorphism analyses comparing cultivated pearl millet with the wild form Pennisetum glaucum showed that the nucleotide diversity of the TB1 gene dramatically dropped in a region upstream of the transcription start site.”
From Shaping plant architecture (2015) · cites this paper as Remigereau et al., 2011
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
Statistical method for testing the neutral mutation hypothesis by DNA polymorphism.
Tajima, F. (1989) · Genetics · doi:10.1093/genetics/123.3.585 · Cited by 14,056
DnaSP, DNA polymorphism analyses by the coalescent and other methods
Rozas, J., Sánchez-DelBarrio, J. C., Messeguer, X., & Rozas, R. (2003) · Bioinformatics · doi:10.1093/bioinformatics/btg359 · Cited by 6,133
Statistical tests of neutrality of mutations.
Fu, Y., & Li, W. (1993) · Genetics · doi:10.1093/genetics/133.3.693 · Cited by 4,067
MEGA: A biologist-centric software for evolutionary analysis of DNA and protein sequences
Kumar, S., Nei, M., Dudley, J. T., & Tamura, K. (2008) · Briefings in Bioinformatics · doi:10.1093/bib/bbn017 · Cited by 3,511
VISTA: computational tools for comparative genomics
Frazer, K. A., Pachter, L. S., Poliakov, A., Rubin, E. M., & Dubchak, I. L. (2004) · Nucleic Acids Research · doi:10.1093/nar/gkh458 · Cited by 2,821
Generating samples under a Wright–Fisher neutral model of genetic variation
Hudson, R. R. (2002) · Bioinformatics · doi:10.1093/bioinformatics/18.2.337 · Cited by 2,389
The Molecular Genetics of Crop Domestication
Doebley, J., Gaut, B. S., & Smith, B. D. (2006) · Cell · doi:10.1016/j.cell.2006.12.006 · Cited by 2,033
A Test of Neutral Molecular Evolution Based on Nucleotide Data
Hudson, R. R., Kreitman, M., & Aguadé, M. (1987) · Genetics · doi:10.1093/genetics/116.1.153 · Cited by 1,759
The evolution of apical dominance in maize
Doebley, J., Stec, A., & Hubbard, L. (1997) · Nature · doi:10.1038/386485a0 · Cited by 1,552
The nature of selection during plant domestication
Purugganan, M. D., & Fuller, D. Q. (2009) · Nature · doi:10.1038/nature07895 · Cited by 1,085
Research works printed but not linked: 1
- J Doebley, 1999, The structure of teosinte-branched one: a progress report., Maize Genetics Cooperation Newsletter, 73, 82
Cited by
Evolution of crop species: genetics of domestication and diversification
Meyer, R. S., & Purugganan, M. D. (2013) · Nature Reviews Genetics · doi:10.1038/nrg3605 · Cited by 1,231
A Bountiful Harvest: Genomic Insights into Crop Domestication Phenotypes
Olsen, K. M., & Wendel, J. F. (2013) · Annual Review of Plant Biology · doi:10.1146/annurev-arplant-050312-120048 · Cited by 403
Evolutionary Insights into the Nature of Plant Domestication
Purugganan, M. D. (2019) · Current Biology · doi:10.1016/j.cub.2019.05.053 · Cited by 374
Teichmann, T., & Muhr, M. (2015) · Frontiers in Plant Science · doi:10.3389/fpls.2015.00233 · Cited by 228
“Interestingly, comparative QTL mapping revealed that also in pearl millet, TB1 was the molecular target of domestication (Remigereau et al., 2011).”
BackgroundInfluentialMolecular mechanisms involved in convergent crop domestication
Lenser, T., & Theißen, G. (2013) · Trends in Plant Science · doi:10.1016/j.tplants.2013.08.007 · Cited by 195
Glémin, S., & Ronfort, J. (2012) · Evolution · doi:10.1111/j.1558-5646.2012.01778.x · Cited by 162
Guan, J., Koch, K. E., Suzuki, M., Wu, S., Latshaw, S. P., Petruff, T. A., Goulet, C., Klee, H. J., & McCarty, D. R. (2012) · PLANT PHYSIOLOGY · doi:10.1104/pp.112.204503 · Cited by 159
Diversity, expansion, and evolutionary novelty of plant DNA-binding transcription factor families
Lehti‐Shiu, M. D., Panchy, N. L., Wang, P., Uygun, S., & Shiu, S. (2016) · Biochimica et Biophysica Acta (BBA) - Gene Regulatory Mechanisms · doi:10.1016/j.bbagrm.2016.08.005 · Cited by 121
Dong, Z., Li, W., Unger‐Wallace, E., Yang, J., Vollbrecht, E., & Chuck, G. S. (2017) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1714960114 · Cited by 116
Dawson, I. K., Powell, W., Hendre, P. S., Bančič, J., Hickey, J. M., Kindt, R., Hoad, S. P., Hale, I. L., & Jamnadass, R. (2019) · New Phytologist · doi:10.1111/nph.15895 · Cited by 111
Exploration of Genetic and Genomic Resources for Abiotic and Biotic Stress Tolerance in Pearl Millet
Shivhare, R., & Lata, C. (2017) · Frontiers in Plant Science · doi:10.3389/fpls.2016.02069 · Cited by 106
Pearl millet response to drought: A review
Shrestha, N., Hu, H., Shrestha, K., & Doust, A. N. (2023) · Frontiers in Plant Science · doi:10.3389/fpls.2023.1059574 · Cited by 106
Genomics of sorghum local adaptation to a parasitic plant
Bellis, E. S., Kelly, E. A., Lorts, C. M., Gao, H., DeLeo, V. L., Rouhan, G., Budden, A., Bhaskara, G. B., Hu, Z., Muscarella, R., et al. (2020) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1908707117 · Cited by 103
Orphan Crops and their Wild Relatives in the Genomic Era
Ye, C., & Fan, L. (2020) · Molecular Plant · doi:10.1016/j.molp.2020.12.013 · Cited by 98
Alam, O., & Purugganan, M. D. (2024) · The Plant Cell · doi:10.1093/plcell/koae013 · Cited by 91
Casting light on the architecture of crop yield
Murchie, E. H., & Burgess, A. J. (2022) · Crop and Environment · doi:10.1016/j.crope.2022.03.009 · Cited by 74
Similar traits, different genes? Examining convergent evolution in related weedy rice populations
Thurber, C. S., Jia, M. H., Jia, Y., & Caicedo, A. L. (2012) · Molecular Ecology · doi:10.1111/mec.12147 · Cited by 69
Evolutionary trajectories of duplicated FT homologues and their roles in soybean domestication
Wu, F., Sedivy, E. J., Price, W. B., Haider, W., & Hanzawa, Y. (2017) · The Plant Journal · doi:10.1111/tpj.13521 · Cited by 62
Evolutionary insights into plant breeding
Turner, S., Mabry, M. E., Beissinger, T. M., Ross‐Ibarra, J., & Pires, J. C. (2020) · Current Opinion in Plant Biology · doi:10.1016/j.pbi.2020.03.003 · Cited by 56
Genomic footprints of sorghum domestication and breeding selection for multiple end uses
Wu, X., Liu, Y., Luo, H., Shang, L., Leng, C.-Y., Liu, Z., Li, Z., Lu, X., Cai, H., Hao, H., et al. (2022) · Molecular Plant · doi:10.1016/j.molp.2022.01.002 · Cited by 52
The role of pangenomics in orphan crop improvement
Hu, H., Zhao, J., Thomas, W. J. W., Batley, J., & Edwards, D. (2025) · Nature Communications · doi:10.1038/s41467-024-55260-4 · Cited by 53
Evidence for Selection on Gene Expression in Cultivated Rice (Oryza sativa)
House, M., Griswold, C. K., & LUKENS, L. N. (2014) · Molecular Biology and Evolution · doi:10.1093/molbev/msu110 · Cited by 38
MATING SYSTEM, HALDANE'S SIEVE, AND THE DOMESTICATION PROCESS
Ronfort, J., & Glémin, S. (2012) · Evolution · doi:10.1111/evo.12025 · Cited by 37
Parallelism and convergence in post-domestication adaptation in cereal grasses
Woodhouse, M. R., & Hufford, M. B. (2019) · Philosophical Transactions of the Royal Society B Biological Sciences · doi:10.1098/rstb.2018.0245 · Cited by 30
Identification of candidate genes for dissecting complex branch number trait in chickpea
Bajaj, D., Upadhyaya, H. D., Das, S., Kumar, V., Gowda, C. L. L., Sharma, S., Tyagi, A. K., & Parida, S. K. (2016) · Plant Science · doi:10.1016/j.plantsci.2016.01.004 · Cited by 29
A transposon in tb1 drove maize domestication
Tsiantis, M. (2011) · Nature Genetics · doi:10.1038/ng.986 · Cited by 23
Evolutionary dynamics of cycle length in pearl millet: the role of farmer’s practices and gene flow
Lakis, G., Ousmane, A. M., Sanoussi, D., Habibou, A., Badamassi, M., Lamy, F., Jika, A. K. N., Sidikou, R., Adam, T., Sarr, A., et al. (2011) · Genetica · doi:10.1007/s10709-012-9633-1 · Cited by 22
Self-citationIdentifying and Classifying Shared Selective Sweeps from Multilocus Data
Harris, A. M., & DeGiorgio, M. (2020) · Genetics · doi:10.1534/genetics.120.303137 · Cited by 21
A deep-time landscape of plant cis-regulatory sequence evolution
Amundson, K., Hendelman, A., Ciren, D., Yang, H., de Neve, A. E., Tal, S., Sulema, A., Jackson, D. P., Bartlett, M. E., Lippman, Z. B., et al. (2026) · Science · doi:10.1126/science.adt8983 · Cited by 22
Evolution of Neutral and Flowering Genes along Pearl Millet (Pennisetum glaucum) Domestication
Lakis, G., Navascués, M., Rekima, S., Simon, M., Remigereau, M., Leveugle, M., Takvorian, N., Lamy, F., Depaulis, F., & Robert, T. (2012) · PLoS ONE · doi:10.1371/journal.pone.0036642 · Cited by 17
Self-citationPrakash, N. R., Chhabra, R., Zunjare, R. U., Muthusamy, V., & Hossain, F. (2020) · 3 Biotech · doi:10.1007/s13205-020-2052-6 · Cited by 16
Description of the Family, Vegetative Morphology and Anatomy
Kellogg, E. A. (2015) · Springer eBooks · doi:10.1007/978-3-319-15332-2_1 · Cited by 13
Hard versus soft selective sweeps during domestication and improvement in soybean
Zhong, L., Zhu, Y., & Olsen, K. M. (2022) · Molecular Ecology · doi:10.1111/mec.16454 · Cited by 12
Zhong, L., Yang, Q., Yan, X., Yu, C., Liu, S., Zhang, X., & Zhu, Y. (2017) · Molecular Ecology · doi:10.1111/mec.14209 · Cited by 12
Dussert, Y., Remigereau, M., Fontaine, M. C., Snirc, A., Lakis, G., Stoeckel, S., Langin, T., Sarr, A., & Robert, T. (2012) · Molecular Ecology · doi:10.1111/mec.12139 · Cited by 11
Self-citationMolecular and Genomic Tools Provide Insights on Crop Domestication and Evolution
Geleta, M., & Ortiz, R. O. (2015) · Advances in agronomy · doi:10.1016/bs.agron.2015.09.005 · Cited by 11
Accelerating crop domestication through genome editing for sustainable agriculture
Pattnaik, D., Avinash, S. P., Panda, S., Bansal, K. C., Chakraborti, M., Kar, M. K., Baig, M. J., & Molla, K. A. (2023) · Journal of Plant Biochemistry and Biotechnology · doi:10.1007/s13562-023-00837-1 · Cited by 10
Plant domestication revisited: Genomic insights into origins, mechanisms, and convergent evolution
Cao, Y., Yan, J., Ross‐Ibarra, J., & Yang, N. (2025) · iScience · doi:10.1016/j.isci.2025.114062 · Cited by 7
Omics-driven utilization of wild relatives for empowering pre-breeding in pearl millet
Kapoor, C., Anamika, Sankar, S. M., Singh, S. P., Singh, N., & Kumar, S. (2024) · Planta · doi:10.1007/s00425-024-04423-0 · Cited by 3
Liu, T., Liu, X., He, J., Dong, K., Zhang, L., Li, Y., Ren, R., & Yang, T. (2024) · Theoretical and Applied Genetics · doi:10.1007/s00122-023-04524-6 · Cited by 2
Past, present and future of local crop evolution
Canales, N. A., Ryan, P., Jackson, A. C., Le-Hong, P., Borrell, J. S., Davis, A. P., & Gutaker, R. M. (2026) · Plants People Planet · doi:10.1002/ppp3.70172 · Cited by 1
Odonkor, S. E. (2015) · Cited by 1
Muhr, M. (2016) · eDiss (Georg-August-Universität Göttingen) · doi:10.53846/goediss-5648 · Cited by 1
Goron, T. L. (2017) · The Atrium (University of Guelph)
Kumar, S., Kumari, R., & Sharma, V. (2020) · Revista de Fomento Social · doi:10.16943/ptinsa/2020/154986
Kellogg, E. A. (2015) · Springer eBooks · doi:10.1007/978-3-319-15332-2_12
Dharbaranyam, B., Sakthivel, K., & Venkataraman, G. (2024) · CABI eBooks · doi:10.1079/9781800623033.0010
Asselin, S. R. (2019) · Mspace (University of Manitoba)
Dynamique évolutive de la durée du cycle de mil : effet des flux de gènes et des pratiques paysannes
Lakis, G. (2012) · theses.fr (ABES) · doi:10.70675/878c9526zfe52z48a1zadddzdc99144edf46
Self-citation
Metadata
- Authors
- Remigereau, M.-S., Lakis, G., Rekima, S., Leveugle, M., Fontaine, M. C., Langin, T., Sarr, A., & Robert, T.
- Affiliations
- Université Paris-Sud (FR)
- Corresponding author
- Robert, Thierry
- Venue
- PLoS ONE
- Publisher
- Public Library of Science (PLoS)
- Published
- 2011-07-22
- Volume
- 6
- Issue
- 7
- Pages
- e22404
- ISSN
- 1932-6203 (ISSN-L)
- PMC
- PMC3142148
- OpenAlex
- W2094310327
- Cited by
- 48
- References
- 58
- Citations by year
- 2026: 2 · 2025: 2 · 2024: 4 · 2023: 2 · 2022: 3 · 2020: 5 · 2019: 3 · 2018: 1 · 2017: 5 · 2016: 4 · 2015: 5 · 2014: 1 · 2013: 3 · 2012: 6
- FWCI
- 2.39
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Locations
- PLoS ONE (publishedVersion, cc-by)
- Europe PMC (PubMed Central) (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- HAL (submittedVersion, cc-by-nc-nd)
- DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion)
- Figshare (submittedVersion, cc-by)
- Funders
- Agence Nationale de la Recherche (ANR-06-BDIV-0003)
- Centre National de la Recherche Scientifique
- Topics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Genetics › Genetic Mapping and Diversity in Plants and Animals
- Life Sciences › Agricultural and Biological Sciences › Plant Science › Plant Genetic and Mutation Studies
- Life Sciences › Agricultural and Biological Sciences › Plant Science › Plant Molecular Biology Research
- Keywords
- pearl millet, TEOSINTE BRANCHED1, plant domestication, plant architecture, parallel evolution, soft selection, selective sweeps, domestication syndrome, maize, gene regulatory regions, introgression, QTL mapping, molecular evolution
- MeSH terms
- Edible Grain, Chromosome Mapping, Cloning, Molecular, Hybridization, Genetic, Plant Proteins, Polymorphism, Genetic, Selection, Genetic, Sequence Homology, Nucleic Acid, Gene Expression Regulation, Plant, Evolution, Molecular, Pennisetum, Quantitative Trait Loci, Genetic Loci
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
Data sources
Bibliographic data: Semantic Scholar, OpenAlex, Crossref.
Contains information from the Semantic Scholar Academic Graph Datasets, made available under the ODC Attribution License (ODC-BY 1.0).
Semantic Scholar’s data is described in: Kinney, R., et al. (2023). The Semantic Scholar Open Data Platform. arXiv:2301.10140.
