

The DOI matches its Crossref record; 3 of the 3 references it cites were found in a registry or an index.
Structure and evolutionary history of a large family of NLR proteins in the zebrafish
Published version of a preprint
Abstract
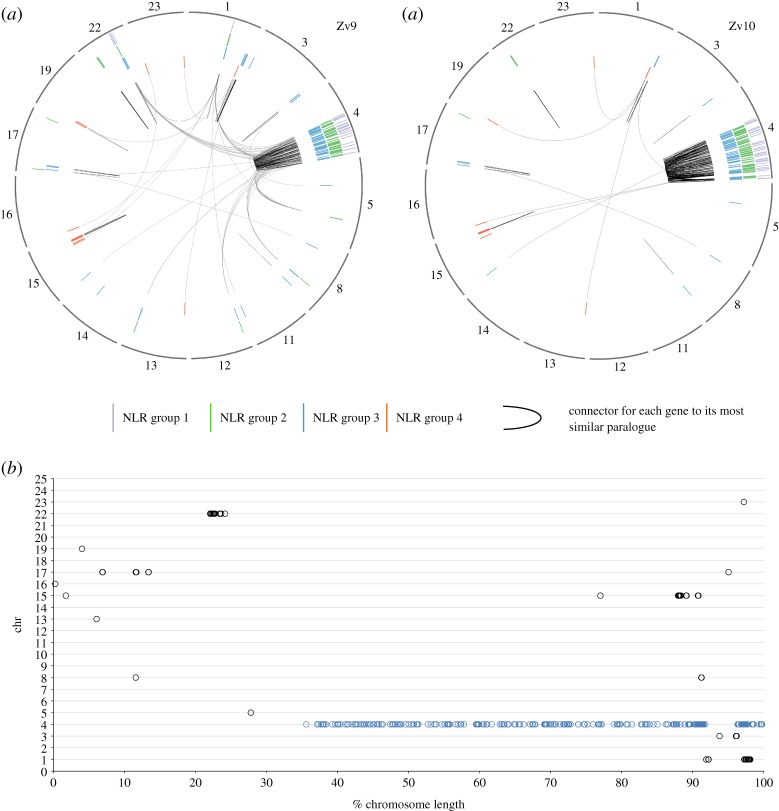
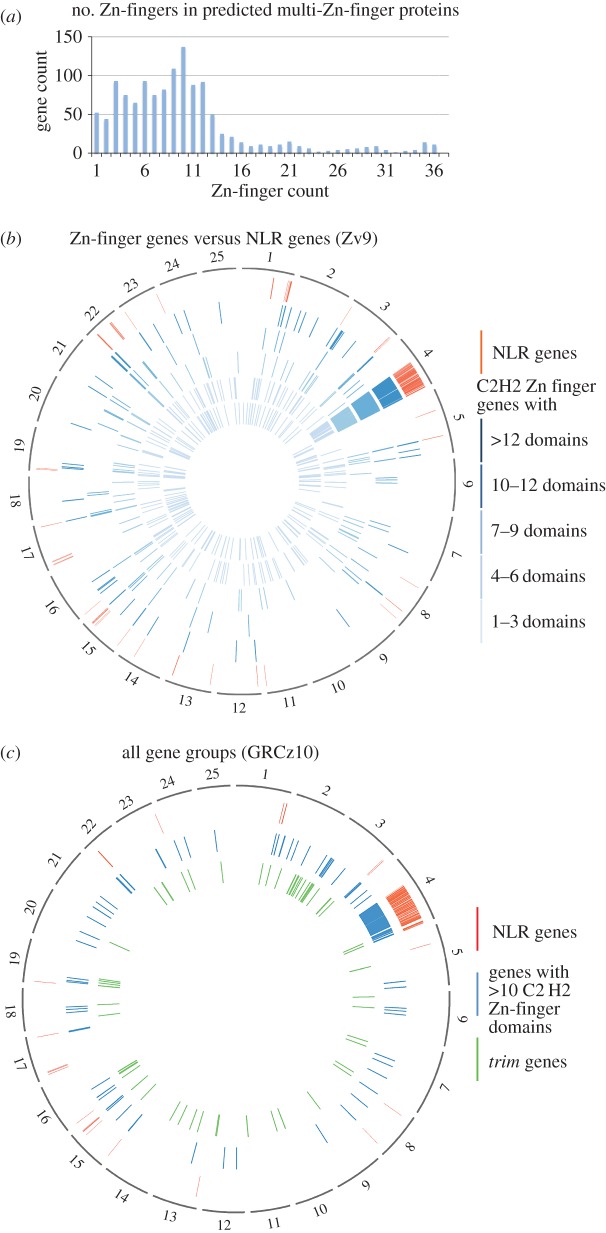
Multicellular eukaryotes have evolved a range of mechanisms for immune recognition. A widespread family involved in innate immunity are the NACHT-domain and leucine-rich-repeat-containing (NLR) proteins. Mammals have small numbers of NLR proteins, whereas in some species, mostly those without adaptive immune systems, NLRs have expanded into very large families. We describe a family of nearly 400 NLR proteins encoded in the zebrafish genome. The proteins share a defining overall structure, which arose in fishes after a fusion of the core NLR domains with a B30.2 domain, but can be subdivided into four groups based on their NACHT domains. Gene conversion acting differentially on the NACHT and B30.2 domains has shaped the family and created the groups. Evidence of positive selection in the B30.2 domain indicates that this domain rather than the leucine-rich repeats acts as the pathogen recognition module. In an unusual chromosomal organization, the majority of the genes are located on one chromosome arm, interspersed with other large multigene families, including a new family encoding zinc-finger proteins. The NLR-B30.2 proteins represent a new family with diversity in the specific recognition module that is present in fishes in spite of the parallel existence of an adaptive immune system.
Overview
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Integrity signals
Registry
Cites
Statistics
Figures
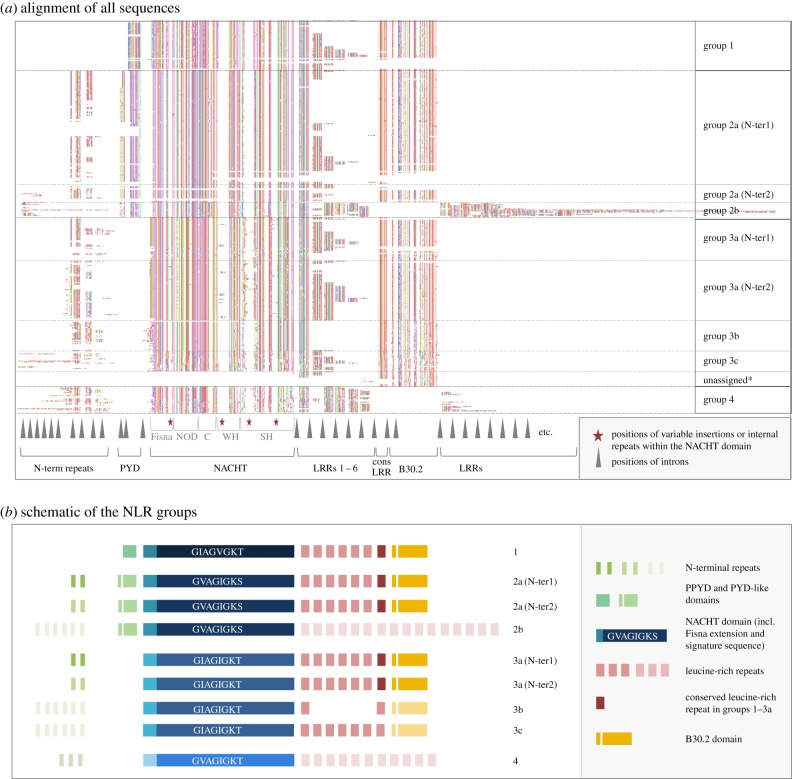
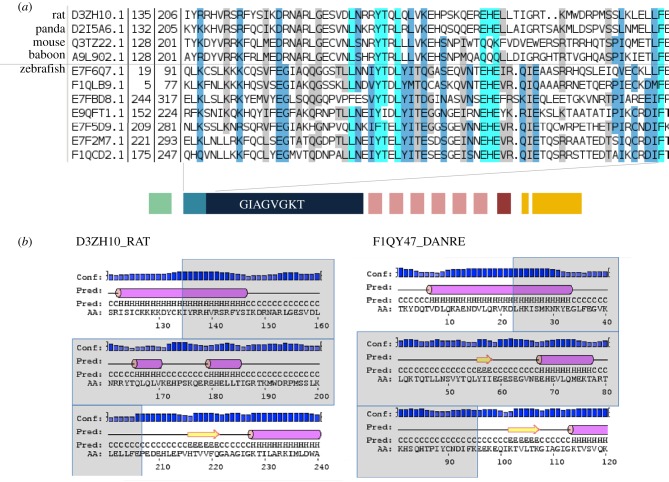
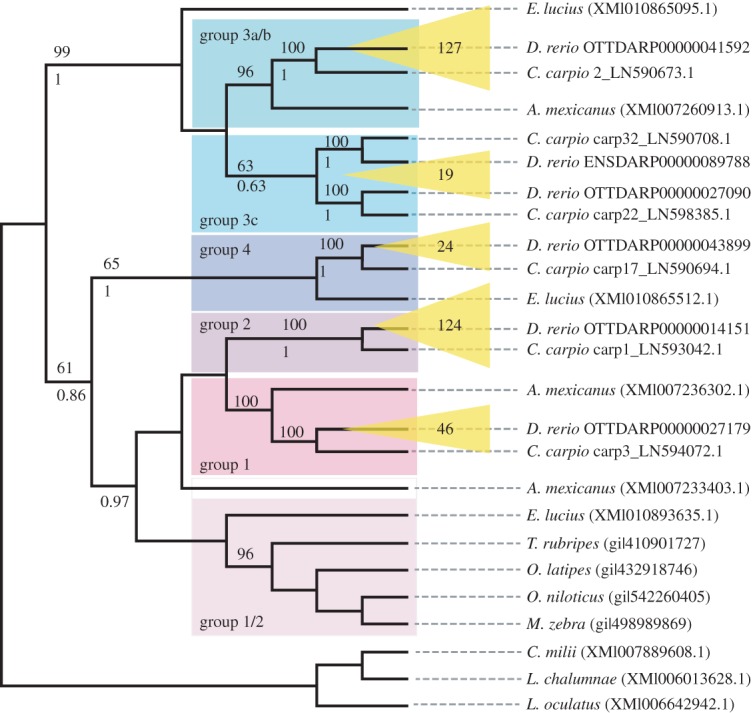
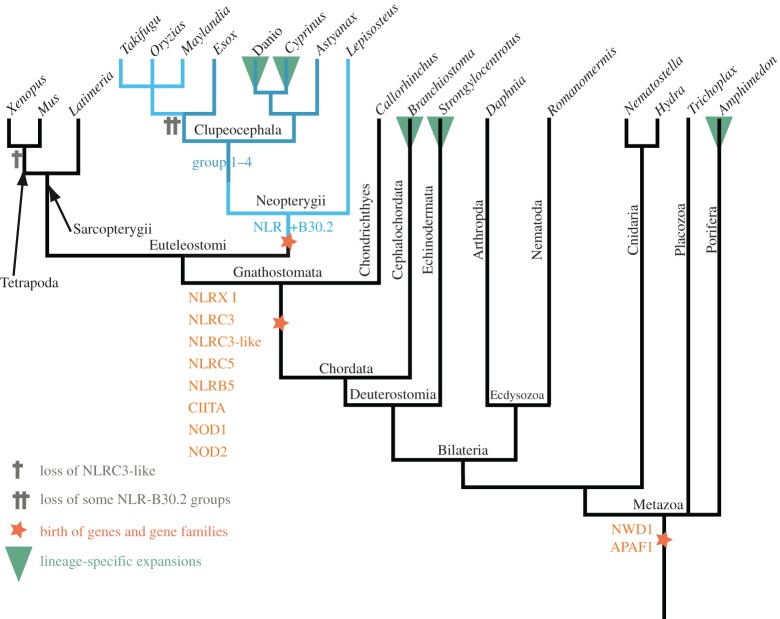
Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
In the citing paper
“In previous versions of this genome assembly (i.e. Zv6) the NLR genes were more or less collapsed.”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
In the citing paper
“As a further complicating repeat-issue they occur interspersed with Zn-finger genes and arranged irregularly.”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
In the citing paper
“The repeated nature of this huge genomic architecture makes it difficult to be confident that all the genes have been properly assembled and annotated, even with manual annotation and curation (76).”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
In the citing paper
“The specific organization of the NLR and Zn-finger genes is likely the result of multiple different local duplications.”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
In the citing paper
“However, zebrafish assembly GRCz10 was created with substantial efforts in BAC and fosmid clones to close gaps, which enabled researchers to show that 159 of the 368 identified NLR genes are present as TRs on the long arm of chromosome 4 (76).”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
In the citing paper
“However, zebrafish assembly GRCz10 was created with substantial efforts in BAC and fosmid clones to close gaps, which enabled researchers to show that 159 of the 368 identified NLR genes are present as TRs on the long arm of chromosome 4 (76).”
From Tandem repeats lead to sequence assembly errors and impose multi-level challenges for genome and protein databases (2019) · cites this paper as [76]
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
RAxML-VI-HPC: maximum likelihood-based phylogenetic analyses with thousands of taxa and mixed models
Stamatakis, A. (2006) · Bioinformatics · doi:10.1093/bioinformatics/btl446 · Cited by 15,582
The zebrafish reference genome sequence and its relationship to the human genome.
Howe, K., Clark, M. D., Torroja, C. F., Torrance, J., Berthelot, C., Muffato, M., Collins, J. E., Humphray, S., McLaren, K., Matthews, L., et al. (2013) · Nature · doi:10.1038/nature12111 · Cited by 5,100
Self-citationTLRs, NLRs and RLRs: a trinity of pathogen sensors that co-operate in innate immunity
Creagh, E. M., & O’Neill, L. A. J. (2006) · Trends in Immunology · doi:10.1016/j.it.2006.06.003 · Cited by 762
Research works printed but not linked: 59
- 10.1016/S0968-0004(00)01577-2 · DOI
- 10.1371/journal.pone.0002119 · DOI
- 10.1016/j.immuni.2008.02.005 · DOI
- 10.1177/09680519050110060301 · DOI
- 10.1189/jlb.1205758 · DOI
- 10.1186/gb-2007-8-11-r251 · DOI · Paper page
- 10.1038/ni.1985 · DOI
- 10.1016/j.coi.2011.12.006 · DOI
- 10.1371/journal.pone.0066859 · DOI
- 10.1016/j.dci.2014.02.014 · DOI
- 10.1016/j.dci.2014.03.025 · DOI
- 10.1186/1471-2148-8-42 · DOI
- 10.1186/1741-7007-7-7 · DOI
- 10.1101/gr.7.5.541 · DOI
- 10.1073/pnas.1303541110 · DOI
- 10.1093/molbev/mst174 · DOI
- 10.1016/j.ydbio.2006.08.048 · DOI
- 10.1186/s13742-015-0052-y · DOI
- 10.1023/A:1013776323077 · DOI
- 10.1016/j.dci.2011.08.010 · DOI
- 10.18632/oncotarget.1850 · DOI
- 10.1101/gr.069674.107 · DOI
- 10.1186/gb-2002-3-2-research0008 · DOI
- 10.1098/rspb.2012.1108 · DOI
- 10.1073/pnas.0802432105 · DOI
- 10.1073/pnas.1314540110 · DOI
- Hamada M, 2012, The complex NOD-like receptor repertoire of the coral Acropora digitifera includes novel domain combinations, Mol. Biol. Evol., 30
- 10.1186/1471-2148-8-225 · DOI
- 10.1016/j.imlet.2005.11.022 · DOI
- 10.1146/annurev.bi.58.070189.002453 · DOI
- 10.1007/s002510050593 · DOI
- 10.1084/jem.164.6.2083 · DOI
- 10.1016/j.molcel.2006.11.009 · DOI
- 10.1007/s10709-009-9355-1 · DOI
- 10.1534/genetics.166.3.1553 · DOI
- 10.1038/nature02343 · DOI
- 10.1146/annurev.biochem.74.082803.133347 · DOI
- 10.1016/j.cell.2006.02.015 · DOI
- 10.1093/intimm/dxp017 · DOI
- 10.1016/S0145-305X(03)00103-4 · DOI
- 10.1371/journal.pone.0040701 · DOI
- 10.1534/genetics.114.169284 · DOI
- 10.1038/ng.3280 · DOI
- 10.1007/s00335-015-9583-x · DOI
- 10.1016/S0091-679X(04)77012-0 · DOI
- Sievers F, 2011, Fast, scalable generation of high-quality protein multiple sequence alignments using Clustal Omega, Mol. Syst. Biol., 7, 1, 10.1038/msb.2011.75 · DOI
- 10.1186/1471-2105-5-113 · DOI
- 10.1093/bioinformatics/btu642 · DOI
- 10.1093/bioinformatics/btp348 · DOI
- 10.1093/bioinformatics/btr088 · DOI
- 10.1186/1471-2105-8-460 · DOI
- 10.1093/bioinformatics/btu544 · DOI
- 10.1093/nar/gkp335 · DOI · Paper page
- 10.1093/bioinformatics/btg1080 · DOI · Paper page
- 10.1016/S1672-0229(10)60008-3 · DOI
- 10.1016/S0168-9525(00)02024-2 · DOI · Paper page
- 10.1016/j.bbrc.2012.02.101 · DOI
- Tange O, 2011, Gnu parallel: the command-line power tool
- 10.1109/MCSE.2007.53 · DOI
Cited by
Sorted by citations
Tørresen, O. K., Star, B., Mier, P., Andrade-Navarro, M. A., Bateman, A., Jarnot, P., Gruca, A., Grynberg, M., Kajava, A. V., Promponas, V. J., et al. (2019) · Nucleic Acids Research · doi:10.1093/nar/gkz841 · Cited by 347
Metadata
- Authors
- Howe, K., Schiffer, P. H., Zielinski, J., Wiehe, T., Laird, G. K., Marioni, J. C., Soylemez, O., Kondrashov, F., & Leptin, M.
- Affiliations
- Wellcome Trust Sanger Institute, Cambridge, UK
- Institut für Genetik, Universität zu Köln, Köln, Germany
- Bioinformatics and Genomics Programme, Centre for Genomic Regulation (CRG) 88 Dr. Aiguader, 08003 Barcelona, Spain
- ORCID
- Venue
- Open Biology
- Publisher
- The Royal Society
- Published
- 2016-04
- Volume
- 6
- Issue
- 4
- Pages
- 160009
- ISSN
- 2046-2441
- PMC
- PMC4852459
- Cited by
- 137
- References
- 3
- Language
- en
- Funders
- AGAUR program (2014 SGR 0974)
- Wellcome Trust
- National Human Genome Research Institute (HG002659)
- MINECO (Sev-2012-0208)
- European Research Council (335980_EinME)
- EMBL
- Deutsche Forschungsgemeinschaft (SFB 670 “Zellautonome Immunität”, SFB 680 "Molecular basis of evolutionary innovatio, SPP1819)
- Howard Hughes Medical Institute (55007424)
- Volkswagen Foundation
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
How to cite
Cite CoChat for the checks on this page, and the paper for its own findings.
- This page
- CoChat. (2026). Citation check: Structure and evolutionary history of a large family of NLR proteins in the zebrafish. https://app.cochat.ai/papers/10.1098/rsob.160009
- The paper
- Howe, K., Schiffer, P. H., Zielinski, J., Wiehe, T., Laird, G. K., Marioni, J. C., Soylemez, O., Kondrashov, F., & Leptin, M. (2016). Structure and evolutionary history of a large family of NLR proteins in the zebrafish. Open Biology. https://doi.org/10.1098/rsob.160009
