Cited by 213Gut microbiota and healthDiet, Metabolism, and DiseaseAdipokines, Inflammation, and Metabolic Diseases

The DOI matches its Crossref record; 65 of the 66 references it cites were found in a registry or an index.

Dietary fat and gut microbiota interactions determine diet-induced obesity in mice

Open access

Abstract

Objective Gut microbiota may promote positive energy balance; however, germfree mice can be either resistant or susceptible to diet-induced obesity (DIO) depending on the type of dietary intervention. We here sought to identify the dietary constituents that determine the susceptibility to body fat accretion in germfree (GF) mice. Methods GF and specific pathogen free (SPF) male C57BL/6N mice were fed high-fat diets either based on lard or palm oil for 4 wks. Mice were metabolically characterized at the end of the feeding trial. FT-ICR-MS and UPLC-TOF-MS were used for cecal as well as hepatic metabolite profiling and cecal bile acids quantification, respectively. Hepatic gene expression was examined by qRT-PCR and cecal gut microbiota of SPF mice was analyzed by high-throughput 16S rRNA gene sequencing. Results GF mice, but not SPF mice, were completely DIO resistant when fed a cholesterol-rich lard-based high-fat diet, whereas on a cholesterol-free palm oil-based high-fat diet, DIO was independent of gut microbiota. In GF lard-fed mice, DIO resistance was conveyed by increased energy expenditure, preferential carbohydrate oxidation, and increased fecal fat and energy excretion. Cecal metabolite profiling revealed a shift in bile acid and steroid metabolites in these lean mice, with a significant rise in 17β-estradiol, which is known to stimulate energy expenditure and interfere with bile acid metabolism. Decreased cecal bile acid levels were associated with decreased hepatic expression of genes involved in bile acid synthesis. These metabolic adaptations were largely attenuated in GF mice fed the palm-oil based high-fat diet. We propose that an interaction of gut microbiota and cholesterol metabolism is essential for fat accretion in normal SPF mice fed cholesterol-rich lard as the main dietary fat source. This is supported by a positive correlation between bile acid levels and specific bacteria of the order Clostridiales (phylum Firmicutes ) as a characteristic feature of normal SPF mice fed lard. Conclusions In conclusion, our study identified dietary cholesterol as a candidate ingredient affecting the crosstalk between gut microbiota and host metabolism.

Overview

The claims and statistics of this paper haven’t been checked yet.

Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.

A few free checks a day · papers already verified open instantly · results are public

Integrity signals

Registry

Crossref · 10.1016/j.molmet.2016.10.001

Cites

65 of 65 references verified0 citation errors · 0 not checkable

Statistics

Figures

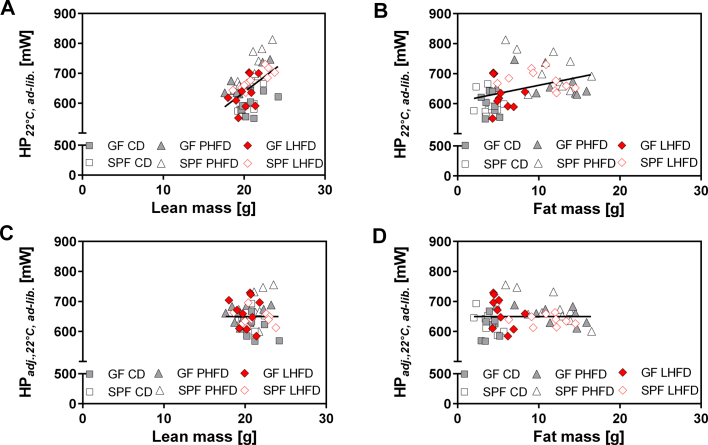
Figure S2 Dependency of daily energy expenditure on body composition. Correlation between daily energy expenditure (HP22 °C, ad-lib.) and lean mass (A) or fat mass (B) following 4 wks of feeding CD, PHFD, or LHFD. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of diet and microbiota status due to small sample size. (A) r2 = 0.26, p < 0.001; (B) r2 = 0.14, p < 0.01. There was no further dependency between daily energy expenditure and lean mass (C) or fat mass (D) after adjusting daily energy expenditure for body composition (HPadj.,22 °C, ad-lib.) by ANCOVA. (C) r2 < 0.001, p = ns; (D) r2 < 0.001, p = ns. adj.: adjusted; ad-lib.: ad-libitum; HP: heat production.
Figure S2 Dependency of daily energy expenditure on body composition. Correlation between daily energy expenditure (HP22 °C, ad-lib.) and lean mass (A) or fat mass (B) following 4 wks of feeding CD, PHFD, or LHFD. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of diet and microbiota status due to small sample size. (A) r2 = 0.26, p < 0.001; (B) r2 = 0.14, p < 0.01. There was no further dependency between daily energy expenditure and lean mass (C) or fat mass (D) after adjusting daily energy expenditure for body composition (HPadj.,22 °C, ad-lib.) by ANCOVA. (C) r2 < 0.001, p = ns; (D) r2 < 0.001, p = ns. adj.: adjusted; ad-lib.: ad-libitum; HP: heat production.CC BY-NC-ND · PubMed Central
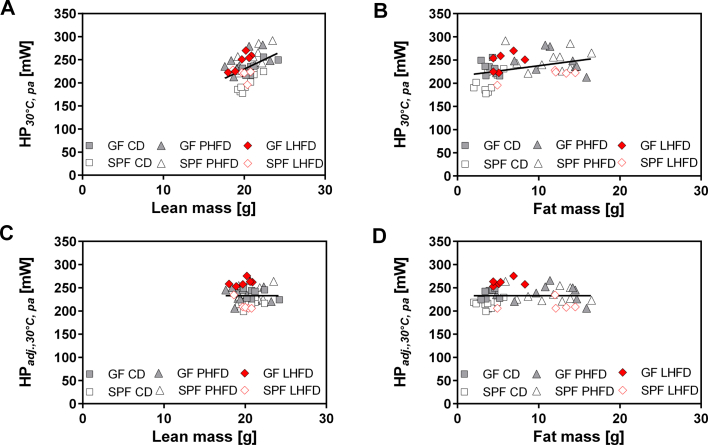
Figure S3 Dependency of basal metabolic rate on body composition. Correlation between basal metabolic rate (HP30 °C, pa) and lean mass (A) or fat mass (B) following 4 wks of feeding CD, PHFD or LHFD. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 5; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 6. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of diet and microbiota status due to small sample size. (A) r2 = 0.19, p < 0.01; (B) r2 = 0.14, p < 0.01. There was no further dependency between basal metabolic rate and lean mass (C) or fat mass (D) after adjusting basal metabolic rate for body composition (HPadj.,30 °C, pa) by ANCOVA. (C) r2 < 0.001, p = ns; (D) r2 < 0.001, p = ns. adj.: adjusted; HP: heat production; pa: post-absorptive.
Figure S3 Dependency of basal metabolic rate on body composition. Correlation between basal metabolic rate (HP30 °C, pa) and lean mass (A) or fat mass (B) following 4 wks of feeding CD, PHFD or LHFD. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 5; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 6. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of diet and microbiota status due to small sample size. (A) r2 = 0.19, p < 0.01; (B) r2 = 0.14, p < 0.01. There was no further dependency between basal metabolic rate and lean mass (C) or fat mass (D) after adjusting basal metabolic rate for body composition (HPadj.,30 °C, pa) by ANCOVA. (C) r2 < 0.001, p = ns; (D) r2 < 0.001, p = ns. adj.: adjusted; HP: heat production; pa: post-absorptive.CC BY-NC-ND · PubMed Central
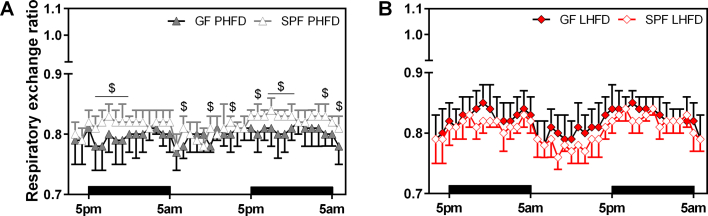
Figure S4 Respiratory exchange ratio of GF mice exposed to PHFD is below that of SPF counterparts and LHFD-FED mice. Comparison of respiratory exchange ratio between GF and SPF mice fed LHFD (p = ns) or PHFD, respectively. $ GF PHFD vs. SPF PHFD: p < 0.05. Black bars above the x-axis indicate nocturnal phases. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Data are shown as means ± sd.
Figure S4 Respiratory exchange ratio of GF mice exposed to PHFD is below that of SPF counterparts and LHFD-FED mice. Comparison of respiratory exchange ratio between GF and SPF mice fed LHFD (p = ns) or PHFD, respectively. $ GF PHFD vs. SPF PHFD: p < 0.05. Black bars above the x-axis indicate nocturnal phases. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Data are shown as means ± sd.CC BY-NC-ND · PubMed Central
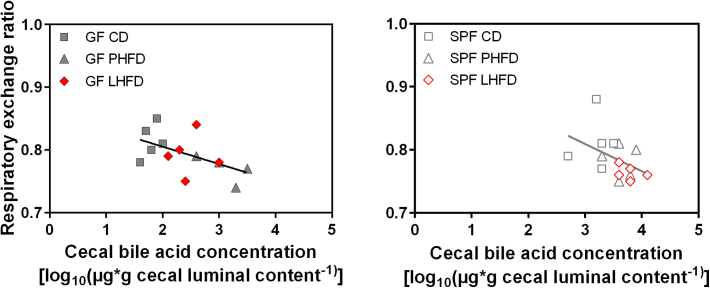
Figure S5 Increased cecal bile acid concentration points to an increased fat oxidation in GF mice. Correlation between cecal bile acid concentration and respiratory exchange ratio measured during basal metabolic rate recordings and represented as the mean of fasted animals following 4 wks of feeding CD, PHFD or LHFD. SPF CD: n = 5; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 5; GF PHFD: n = 4; GF LHFD: n = 5. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of the diet. GF: r2 = 0.26, p < 0.05; SPF: r2 = 0.22, p = ns.
Figure S5 Increased cecal bile acid concentration points to an increased fat oxidation in GF mice. Correlation between cecal bile acid concentration and respiratory exchange ratio measured during basal metabolic rate recordings and represented as the mean of fasted animals following 4 wks of feeding CD, PHFD or LHFD. SPF CD: n = 5; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 5; GF PHFD: n = 4; GF LHFD: n = 5. Linear regression of GF or SPF C57BL/6N mice was calculated irrespective of the diet. GF: r2 = 0.26, p < 0.05; SPF: r2 = 0.22, p = ns.CC BY-NC-ND · PubMed Central
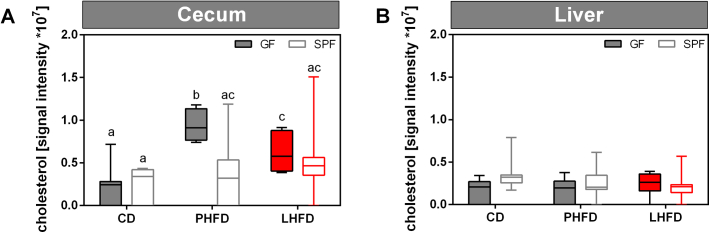
Figure S6 Cecal but not hepatic cholesterol levels are increased in GF mice due to PHFD feeding. (A) Signal intensities of cecal cholesterol measured by ESI-FT-ICR/MS. (B) Signal intensities of hepatic cholesterol measured by ESI-FT-ICR/MS. SPF CD: n = 10 (A)/11 (B); SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 10; GF PHFD: n = 10; GF LHFD: n = 10. Different superscript letters indicate significant differences (p < 0.05).
Figure S6 Cecal but not hepatic cholesterol levels are increased in GF mice due to PHFD feeding. (A) Signal intensities of cecal cholesterol measured by ESI-FT-ICR/MS. (B) Signal intensities of hepatic cholesterol measured by ESI-FT-ICR/MS. SPF CD: n = 10 (A)/11 (B); SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 10; GF PHFD: n = 10; GF LHFD: n = 10. Different superscript letters indicate significant differences (p < 0.05).CC BY-NC-ND · PubMed Central
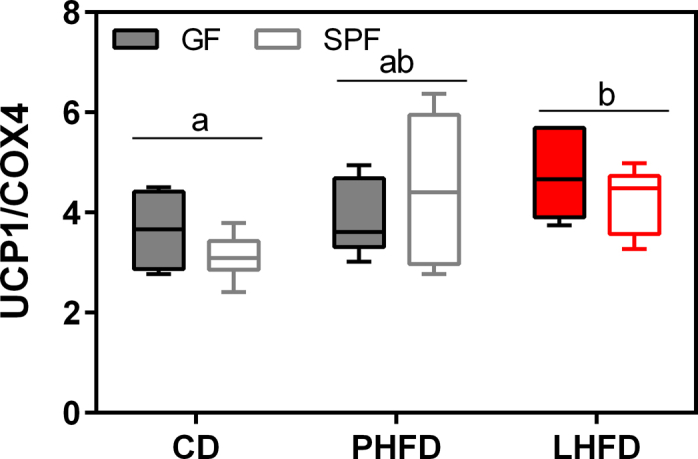
Figure S7 UCP1 protein levels in interscapular brown adipose tissue are altered by diet but not by gut microbiota. SPF CD: n = 7; SPF PHFD: n = 6; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 6. Heat dissipation of interscapular brown adipose tissue is reflected by uncoupling protein 1 (UCP1) protein levels analyzed in the fasted state of mice. Different superscript letters indicate significant diet effects (p < 0.05).
Figure S7 UCP1 protein levels in interscapular brown adipose tissue are altered by diet but not by gut microbiota. SPF CD: n = 7; SPF PHFD: n = 6; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 6. Heat dissipation of interscapular brown adipose tissue is reflected by uncoupling protein 1 (UCP1) protein levels analyzed in the fasted state of mice. Different superscript letters indicate significant diet effects (p < 0.05).CC BY-NC-ND · PubMed Central
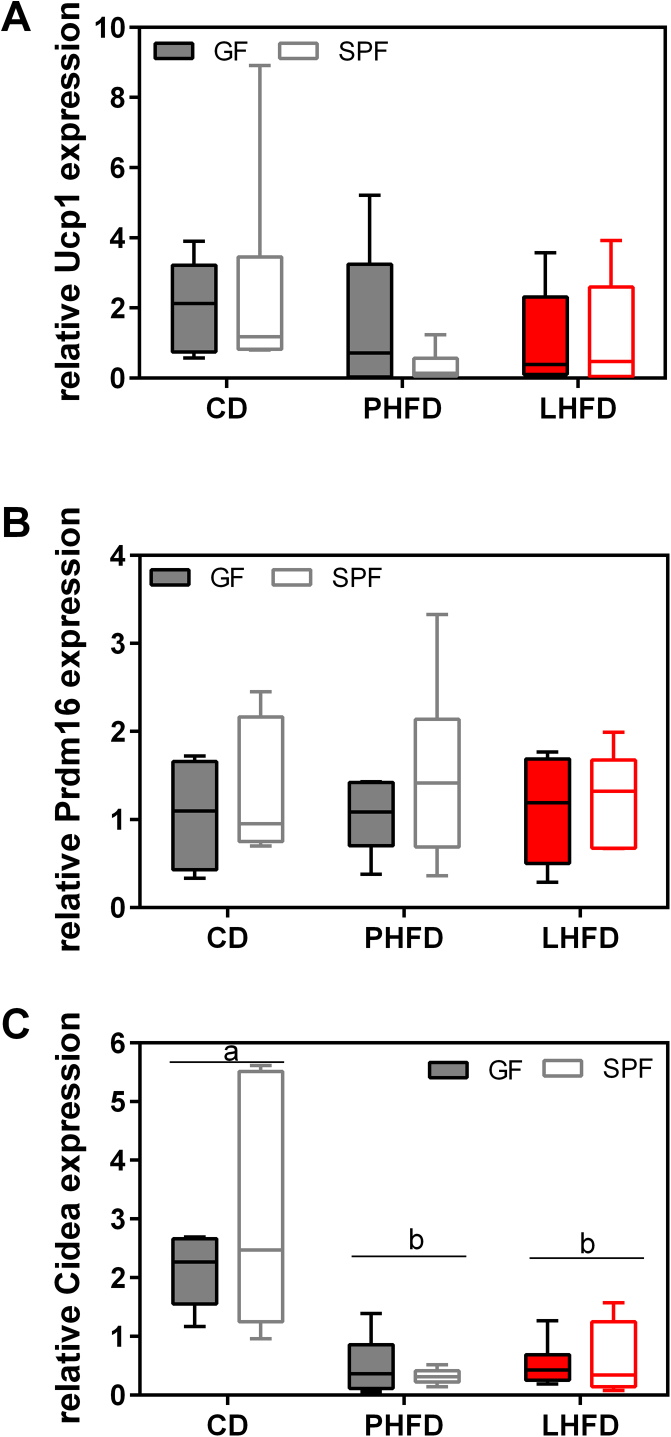
Figure S8 Browning of inguinal white adipose tissue does not explain the lean phenotype of LHFD-FED GF mice. (A) Relative gene expression levels of uncoupling protein 1 (Ucp1), (B) cell death inducing DFFA-like effector (Cidea), and (C) PR domain containing 16 (Prdm16). Data were normalized to the mean mRNA concentration of the three reference genes: transcription factor II B (Tf2b), beta-glucuronidase (Gusb), and beta-actin (Actb). SPF CD: n = 6; SPF PHFD: n = 6; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 6. Gene expression was analyzed in the fasted state of mice. Different superscript letters indicate significant diet effects (p < 0.05).
Figure S8 Browning of inguinal white adipose tissue does not explain the lean phenotype of LHFD-FED GF mice. (A) Relative gene expression levels of uncoupling protein 1 (Ucp1), (B) cell death inducing DFFA-like effector (Cidea), and (C) PR domain containing 16 (Prdm16). Data were normalized to the mean mRNA concentration of the three reference genes: transcription factor II B (Tf2b), beta-glucuronidase (Gusb), and beta-actin (Actb). SPF CD: n = 6; SPF PHFD: n = 6; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 6. Gene expression was analyzed in the fasted state of mice. Different superscript letters indicate significant diet effects (p < 0.05).CC BY-NC-ND · PubMed Central
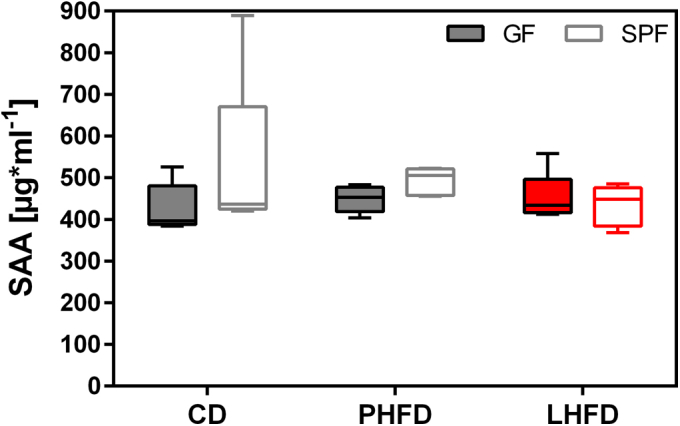
Figure S9 HFD-feeding is not accompanied with acute inflammation. Plasma S-amyloid A levels were measured in the fed state of mice following dissection. SPF CD: n = 5; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 5; GF PHFD: n = 5; GF LHFD: n = 7. p = ns.
Figure S9 HFD-feeding is not accompanied with acute inflammation. Plasma S-amyloid A levels were measured in the fed state of mice following dissection. SPF CD: n = 5; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 5; GF PHFD: n = 5; GF LHFD: n = 7. p = ns.CC BY-NC-ND · PubMed Central
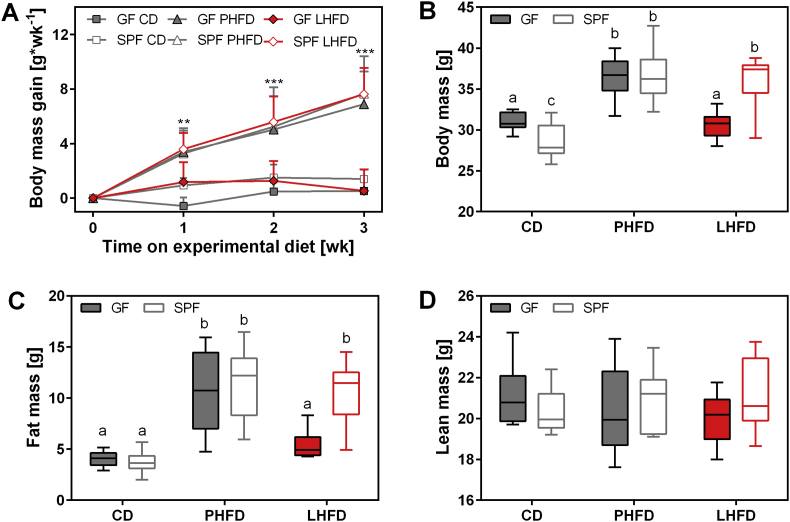
Figure 1 Dietary fat from lard precludes the development of diet-induced obesity in GF mice. (A) Body mass gain during the first 3 wks of experimental feeding. **p < 0.01 and ***p < 0.001 for GF LHFD, GF CD, and SPF CD relative to GF PHFD, SPF PHFD, and SPF LHFD. (B) Body mass, (C) fat mass, and (D) lean mass (p = ns) at the end of the feeding trial (4 wks). Different superscript letters indicate significant statistical differences (p < 0.05). SPF CD: n = 10; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 11; GF LHFD: n = 11.
Figure 1 Dietary fat from lard precludes the development of diet-induced obesity in GF mice. (A) Body mass gain during the first 3 wks of experimental feeding. **p < 0.01 and ***p < 0.001 for GF LHFD, GF CD, and SPF CD relative to GF PHFD, SPF PHFD, and SPF LHFD. (B) Body mass, (C) fat mass, and (D) lean mass (p = ns) at the end of the feeding trial (4 wks). Different superscript letters indicate significant statistical differences (p < 0.05). SPF CD: n = 10; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 11; GF LHFD: n = 11.CC BY-NC-ND · PubMed Central
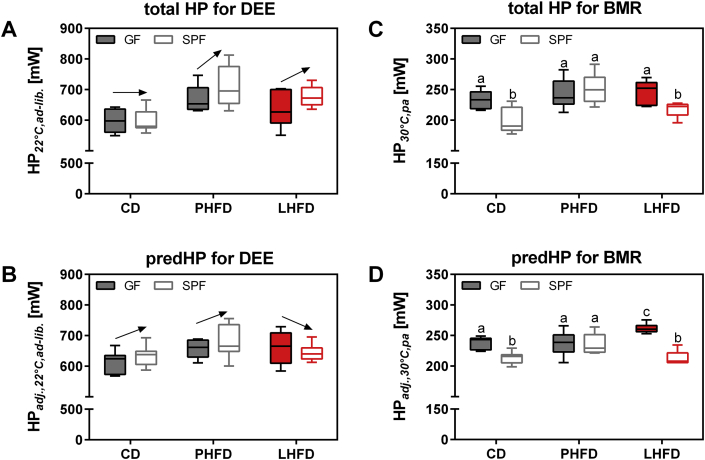
Figure 2 Basal metabolic rate is highest in LHFD-FED GF mice and contributes to increased daily energy expenditure. (A, C) Total and (B, D) predicted heat production of C57BL/6N mice fed ad libitum at ambient temperature (22 °C) (A, B) and fasted at thermoneutrality (30 °C) representing basal metabolism (C, D). Arrows indicate trends in total (A) and predicted (B) daily energy expenditure within dietary groups of GF and SPF mice. Different superscript letters indicate significant statistical differences (p < 0.05). SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10 (A, B)/5 (C, D); GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10 (A, B)/6 (C, D). Data were adjusted according to lean and fat mass over all C57BL/6N mice: HPadj., 22 °C,ad-lib. [mW] = 76.5196 + 7.4048 * fat mass + 24.9719 * lean mass (adjusted r2 = 0.49, p < 0.001). HPadj., 30 °C,pa [mW] = −18.851 + 3.2664 * fat mass + 11.072 * lean mass (adjusted r2 = 0.44, p < 0.001). adj.: adjusted; BMR: basal metabolic rate; DEE: daily energy expenditure; HP: heat production; pa: post-absorptive.
Figure 2 Basal metabolic rate is highest in LHFD-FED GF mice and contributes to increased daily energy expenditure. (A, C) Total and (B, D) predicted heat production of C57BL/6N mice fed ad libitum at ambient temperature (22 °C) (A, B) and fasted at thermoneutrality (30 °C) representing basal metabolism (C, D). Arrows indicate trends in total (A) and predicted (B) daily energy expenditure within dietary groups of GF and SPF mice. Different superscript letters indicate significant statistical differences (p < 0.05). SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10 (A, B)/5 (C, D); GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10 (A, B)/6 (C, D). Data were adjusted according to lean and fat mass over all C57BL/6N mice: HPadj., 22 °C,ad-lib. [mW] = 76.5196 + 7.4048 * fat mass + 24.9719 * lean mass (adjusted r2 = 0.49, p < 0.001). HPadj., 30 °C,pa [mW] = −18.851 + 3.2664 * fat mass + 11.072 * lean mass (adjusted r2 = 0.44, p < 0.001). adj.: adjusted; BMR: basal metabolic rate; DEE: daily energy expenditure; HP: heat production; pa: post-absorptive.CC BY-NC-ND · PubMed Central
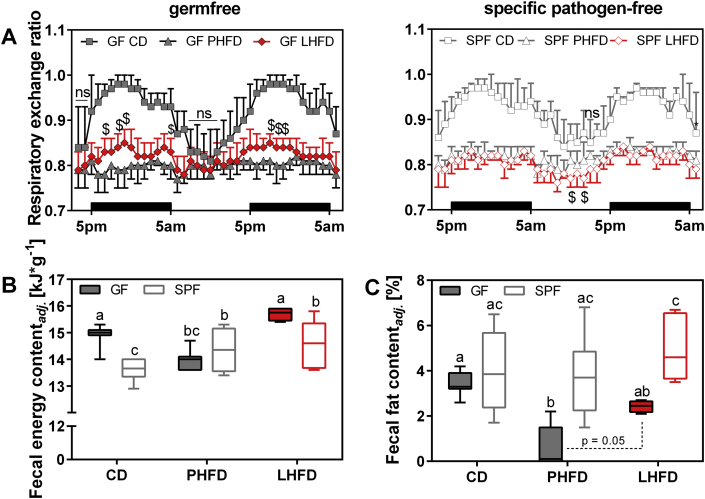
Figure 3 Lean GF mice are characterized by higher respiratory exchange ratio and energy loss in feces. (A) Respiratory exchange ratio in GF and SPF mice fed CD, PHFD, and LHFD. Left: $ GF PHFD vs. GF LHFD: p < 0.05; right: $ SPF PHFD vs. SPF LHFD: p < 0.05. CD-fed GF mice were different to HFD-fed mice at all time points unless otherwise labeled with ns. Different superscript letters indicate significant statistical differences (p < 0.05). Black bars above the x-axis indicate nocturnal phases. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Data are shown as means ± sd. (B) Fecal energy and (C) fat excretion in GF and SPF C57BL/6N mice (housed in groups) during the first and the last week of feeding. Data were adjusted for feces production as well as dietary energy or fat intake, respectively. SPF CD: n = 6; SPF PHFD: n = 6; SPF LHFD: n = 6; GF CD: n = 7; GF PHFD: n = 7; GF LHFD: n = 4. Linear regressions used for adjustment including both GF and SPF mice: Fecal energy contentadj. [kJ*g−1] = 13.0443 + 0.0273 * dietary energy intake − 0.8356 * feces production (adjusted r2 = 0.32, p < 0.001). Fecal fat contentadj. [%] = −0.0723 + 0.0261 * dietary fat intake − 0.3704 * feces production (adjusted r2 = 0.52, p < 0.001). ns: not significant.
Figure 3 Lean GF mice are characterized by higher respiratory exchange ratio and energy loss in feces. (A) Respiratory exchange ratio in GF and SPF mice fed CD, PHFD, and LHFD. Left: $ GF PHFD vs. GF LHFD: p < 0.05; right: $ SPF PHFD vs. SPF LHFD: p < 0.05. CD-fed GF mice were different to HFD-fed mice at all time points unless otherwise labeled with ns. Different superscript letters indicate significant statistical differences (p < 0.05). Black bars above the x-axis indicate nocturnal phases. SPF CD: n = 9; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 8; GF PHFD: n = 9; GF LHFD: n = 10. Data are shown as means ± sd. (B) Fecal energy and (C) fat excretion in GF and SPF C57BL/6N mice (housed in groups) during the first and the last week of feeding. Data were adjusted for feces production as well as dietary energy or fat intake, respectively. SPF CD: n = 6; SPF PHFD: n = 6; SPF LHFD: n = 6; GF CD: n = 7; GF PHFD: n = 7; GF LHFD: n = 4. Linear regressions used for adjustment including both GF and SPF mice: Fecal energy contentadj. [kJ*g−1] = 13.0443 + 0.0273 * dietary energy intake − 0.8356 * feces production (adjusted r2 = 0.32, p < 0.001). Fecal fat contentadj. [%] = −0.0723 + 0.0261 * dietary fat intake − 0.3704 * feces production (adjusted r2 = 0.52, p < 0.001). ns: not significant.CC BY-NC-ND · PubMed Central
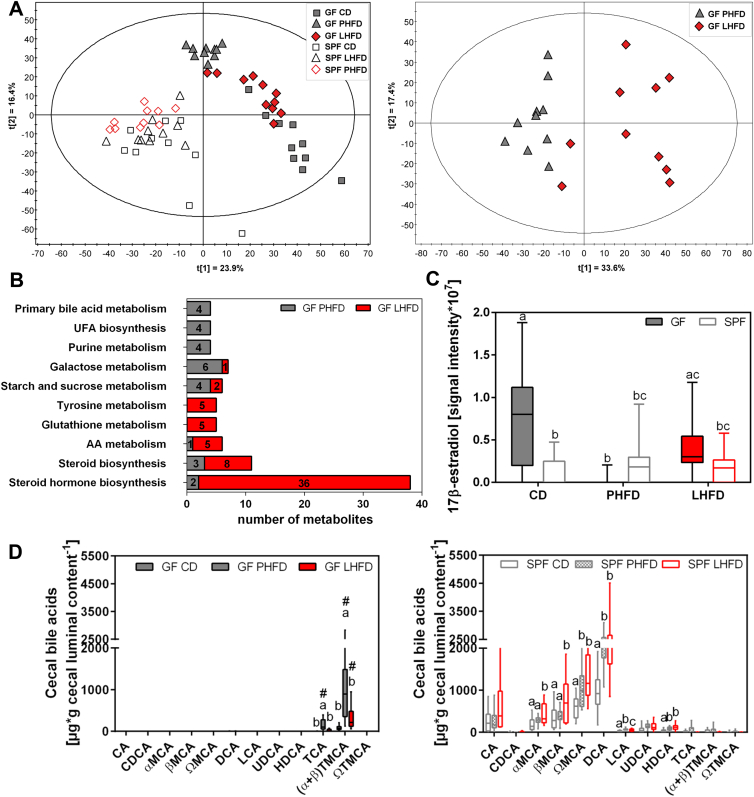
Figure 4 Cholesterol-derived metabolites are altered between lean and obese mice. (A) Metabolite data were visualized by PCA, taking into account annotated mass signals for all SPF and GF mice on CD, LHFD, and PHFD (left) or GF LHFD and PHFD mice alone (right). (B) Output of KEGG metabolic pathway analysis, performed with MetaboAnalyst (top ten) showing the number of metabolites significantly increased in GF mice fed LHFD (red bars) or PHFD (grey bars), but not in SPF counterparts (p < 0.05; Welch's t-test). AA: arachidonic acid; UFA: unsaturated fatty acid. (C) Signal intensity of cecal 17β-estradiol. Different superscript letters indicate significant statistical differences (p < 0.05). (D) Cecal bile acid concentrations in GF and SPF C57BL/6N mice using UPLC-MS. Different superscript letters indicate significant differences within a certain bile acid and among GF or SPF mice, respectively (p < 0.05). # GF vs. SPF: p < 0.05. CA: cholic acid; CDCA: chenodeoxycholic acid; MCA: muricholic acid; DCA: deoxycholic acid; LCA: lithocholic acid; UDCA: ursodeoxycholic acid; HDCA: hyodeoxycholic acid; T: taurine-conjugated species. SPF CD: n = 10; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 10; GF PHFD: n = 10; GF LHFD: n = 10.
Figure 4 Cholesterol-derived metabolites are altered between lean and obese mice. (A) Metabolite data were visualized by PCA, taking into account annotated mass signals for all SPF and GF mice on CD, LHFD, and PHFD (left) or GF LHFD and PHFD mice alone (right). (B) Output of KEGG metabolic pathway analysis, performed with MetaboAnalyst (top ten) showing the number of metabolites significantly increased in GF mice fed LHFD (red bars) or PHFD (grey bars), but not in SPF counterparts (p < 0.05; Welch's t-test). AA: arachidonic acid; UFA: unsaturated fatty acid. (C) Signal intensity of cecal 17β-estradiol. Different superscript letters indicate significant statistical differences (p < 0.05). (D) Cecal bile acid concentrations in GF and SPF C57BL/6N mice using UPLC-MS. Different superscript letters indicate significant differences within a certain bile acid and among GF or SPF mice, respectively (p < 0.05). # GF vs. SPF: p < 0.05. CA: cholic acid; CDCA: chenodeoxycholic acid; MCA: muricholic acid; DCA: deoxycholic acid; LCA: lithocholic acid; UDCA: ursodeoxycholic acid; HDCA: hyodeoxycholic acid; T: taurine-conjugated species. SPF CD: n = 10; SPF PHFD: n = 10; SPF LHFD: n = 10; GF CD: n = 10; GF PHFD: n = 10; GF LHFD: n = 10.CC BY-NC-ND · PubMed Central
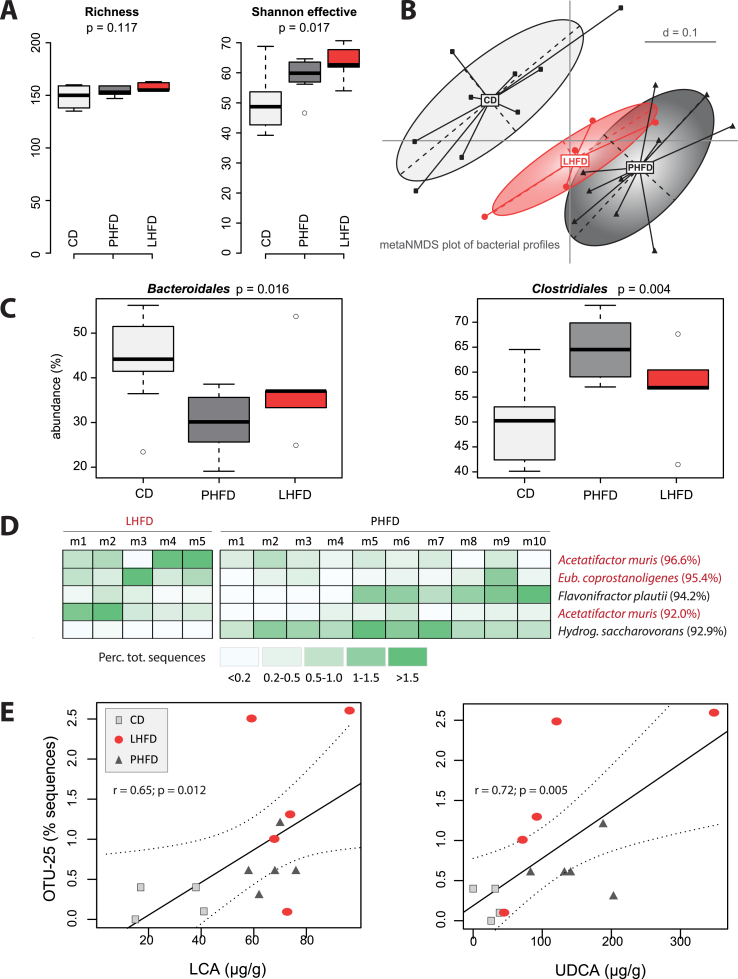
Figure 5 Specific dominant gut bacteria are affected by dietary fat source. Metagenomic DNA isolated from fecal samples (n = 24) was used for amplification of the V3/V4 region of 16S rRNA genes and subsequent sequencing using the Illumina technology. Sequences were analyzed using in-house developed pipelines as described in detail in the methods section. (A) Alpha-diversity analysis. (B) Multidimensional scaling showing differences in diversity between samples (beta-diversity) based on general UniFrac distances. (C) Box plots showing relative sequence abundance of taxonomic groups that were significantly different between mice fed the CD or HFD. (D) Phylotype analysis shown as heatmap of OTU abundances which were significantly different between the two HFD. The identity of OTUs was obtained using EzTaxon based on sequences of approximately 380 bp [64]. Best hits are shown with corresponding sequences similarity. (E) Pearson correlation analysis of Acetatifactor sp. against cecal bile acid concentrations.
Figure 5 Specific dominant gut bacteria are affected by dietary fat source. Metagenomic DNA isolated from fecal samples (n = 24) was used for amplification of the V3/V4 region of 16S rRNA genes and subsequent sequencing using the Illumina technology. Sequences were analyzed using in-house developed pipelines as described in detail in the methods section. (A) Alpha-diversity analysis. (B) Multidimensional scaling showing differences in diversity between samples (beta-diversity) based on general UniFrac distances. (C) Box plots showing relative sequence abundance of taxonomic groups that were significantly different between mice fed the CD or HFD. (D) Phylotype analysis shown as heatmap of OTU abundances which were significantly different between the two HFD. The identity of OTUs was obtained using EzTaxon based on sequences of approximately 380 bp [64]. Best hits are shown with corresponding sequences similarity. (E) Pearson correlation analysis of Acetatifactor sp. against cecal bile acid concentrations.CC BY-NC-ND · PubMed Central
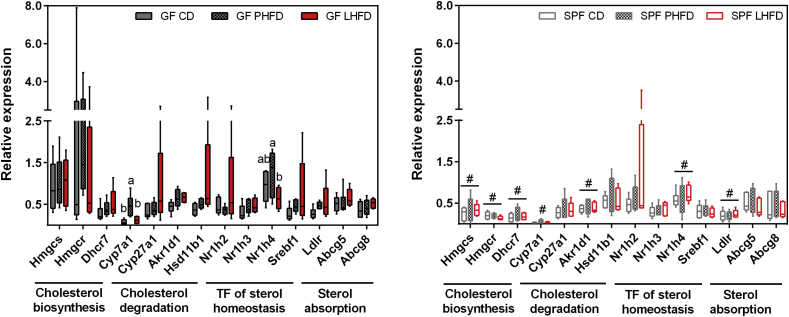
Figure 6 Altered substrate oxidation and fecal fat excretion in lean GF mice is linked to decreased CYP7A1 and NR1H4 expression. SPF CD: n = 6; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 5. Different superscript letters indicate significant differences between feeding groups of GF mice (p < 0.05). # GF vs. SPF: p < 0.05. Abcg5: ATP-binding cassette sub-family G member 5; Abcg8: ATP-binding cassette sub-family G member 8; Akr1d1: aldo-keto-reductase family member 1; Cyp7a1: cholesterol 7 alpha-hydroxylase; Cyp27a1: cholesterol 27 alpha-hydroxylase; Dhcr7: 7-dehydrocholesterol reductase; Hmgcr: 3-hydroxy-3-methylglutaryl Coenzyme A reductase; Hmgcs: 3-hydroxy-3-methylglutaryl Coenzyme A synthase 1; Hsd11b1: hydroxysteroid (11-β) dehydrogenase 1; Ldlr: low density lipoprotein receptor; Nr1h2: nuclear receptor subfamily 1, group H, member 2 (liver X receptor β); Nr1h3: nuclear receptor subfamily 1, group H, member 3 (liver X receptor α); Nr1h4: nuclear receptor subfamily 1, group H, member 4 (farnesoid X receptor α); Srebf1: sterol regulatory element binding transcription factor 1.
Figure 6 Altered substrate oxidation and fecal fat excretion in lean GF mice is linked to decreased CYP7A1 and NR1H4 expression. SPF CD: n = 6; SPF PHFD: n = 5; SPF LHFD: n = 5; GF CD: n = 6; GF PHFD: n = 6; GF LHFD: n = 5. Different superscript letters indicate significant differences between feeding groups of GF mice (p < 0.05). # GF vs. SPF: p < 0.05. Abcg5: ATP-binding cassette sub-family G member 5; Abcg8: ATP-binding cassette sub-family G member 8; Akr1d1: aldo-keto-reductase family member 1; Cyp7a1: cholesterol 7 alpha-hydroxylase; Cyp27a1: cholesterol 27 alpha-hydroxylase; Dhcr7: 7-dehydrocholesterol reductase; Hmgcr: 3-hydroxy-3-methylglutaryl Coenzyme A reductase; Hmgcs: 3-hydroxy-3-methylglutaryl Coenzyme A synthase 1; Hsd11b1: hydroxysteroid (11-β) dehydrogenase 1; Ldlr: low density lipoprotein receptor; Nr1h2: nuclear receptor subfamily 1, group H, member 2 (liver X receptor β); Nr1h3: nuclear receptor subfamily 1, group H, member 3 (liver X receptor α); Nr1h4: nuclear receptor subfamily 1, group H, member 4 (farnesoid X receptor α); Srebf1: sterol regulatory element binding transcription factor 1.CC BY-NC-ND · PubMed Central

Verification

Claims the paper makes

The claims and statistics of this paper haven’t been checked yet.

Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.

A few free checks a day · papers already verified open instantly · results are public

Self-check

Percentages, sums and reported differences re-computed from the paper’s own numbers.

The self-check needs the paper’s full text.

Citations

Cites

Show all 66 references

Cited by

Sorted by citations

Items 201–213 of 213

Metadata

Authors
Kübeck, R., Bonet-Ripoll, C., Hoffmann, C., Walker, A., Müller, V. M., Schüppel, V. L., Lagkouvardos, I., Scholz, B., Engel, K.-H., Daniel, H., Schmitt-Kopplin, P., Haller, D., Clavel, T., & Klingenspor, M.
Affiliations
  • Else Kröner Fresenius Zentrum für Ernährungsmedizin (DE)
  • Helmholtz Munich (DE)
  • Technical University of Munich (DE)
Corresponding author
Klingenspor, Martin
Venue
Molecular Metabolism
Publisher
Elsevier BV
Published
2016-12
Volume
5
Issue
12
Pages
1162-1174
ISSN
2212-8778 (ISSN-L)
OpenAlex
W2530535683
Cited by
211
References
66
Citations by year
2026: 11 · 2025: 16 · 2024: 18 · 2023: 22 · 2022: 32 · 2021: 35 · 2020: 30 · 2019: 19 · 2018: 17 · 2017: 11
FWCI
8.14
Type
journal article
Language
en
Open access
Locations
  • Molecular Metabolism (publishedVersion, cc-by-nc-nd)
  • PubMed Central (publishedVersion, cc-by-nc-nd)
  • PubMed (publishedVersion)
  • PuSH - Publication Server of Helmholtz Zentrum München (submittedVersion, cc-by-nc-nd)
  • DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion, cc-by-sa)
  • mediaTUM (Technical University of Munich) (submittedVersion, other-oa)
  • mediaTUM – the media and publications repository of the Technical University Munich (Technical University Munich) (submittedVersion, other-oa)
  • mediaTUM – the media and publications repository of the Technical University Munich (Technical University Munich) (submittedVersion)
  • Site cant be reached (submittedVersion, cc-by-nc-nd)
Funders
  • ZIEL – Institute for Food and Health
  • Else-Kröner-Fresenius-Stiftung
  • German Research Foundation
Topics
  • Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Gut microbiota and health
  • Health Sciences › Medicine › Endocrinology, Diabetes and Metabolism › Diet, Metabolism, and Disease
  • Health Sciences › Medicine › Endocrinology, Diabetes and Metabolism › Adipokines, Inflammation, and Metabolic Diseases
Keywords
diet-induced obesity, gut microbiota, germ-free mice, dietary cholesterol, lard, palm oil, bile acids, estradiol, energy expenditure, cecal metabolites, hepatic bile acid synthesis, Clostridiales, host-microbe interactions, high-fat diet
MeSH terms
Gastrointestinal Microbiome, Adipose Tissue, Animals, Cholesterol, Cholesterol, Dietary, Dietary Fats, Liver, Male, Mice, Inbred C57BL, Obesity, Lipid Metabolism, Mice, Diet, High-Fat

About these checks

Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.

Statistics and arithmetic are recomputed, not judged.

Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.

What counts as a claim ›How we measure confidence ›How we check this ›

Are you an author, or do you see a problem with this page? Request a review