Cited by 10Vector-borne infectious diseasesInvertebrate Immune Response MechanismsInsect symbiosis and bacterial influences

The DOI matches its Crossref record; 2 of the 2 references it cites were found in a registry or an index.

PERK-mediated antioxidant response is key for pathogen persistence in ticks

Open access

Published version of a preprint

Abstract

A crucial phase in the life cycle of tick-borne pathogens is the time spent colonizing and persisting within the arthropod. Tick immunity is emerging as a key force shaping how transmissible pathogens interact with the vector. How pathogens remain in the tick despite immunological pressure remains unknown. In persistently infected Ixodes scapularis , we found that Borrelia burgdorferi (causative agent of Lyme disease) and Anaplasma phagocytophilum (causative agent of granulocytic anaplasmosis) activate a cellular stress pathway mediated by the endoplasmic reticulum receptor PKR-like ER kinase (PERK) and the central regulatory molecule eIF2α. Disabling the PERK pathway through pharmacological inhibition and RNA interference (RNAi) significantly decreased microbial numbers. In vivo RNAi of the PERK pathway not only reduced the number of A. phagocytophilum and B. burgdorferi colonizing larvae after a bloodmeal but also significantly reduced the number of bacteria that survive the molt. An investigation into PERK pathway-regulated targets revealed that A. phagocytophilum and B. burgdorferi induce activity of the antioxidant response regulator, nuclear factor erythroid 2-related factor 2 (Nrf2). Tick cells deficient for nrf2 expression or PERK signaling showed accumulation of reactive oxygen and nitrogen species in addition to reduced microbial survival. Supplementation with antioxidants rescued the microbicidal phenotype caused by blocking the PERK pathway. Altogether, our study demonstrates that the Ixodes PERK pathway is activated by transmissible microbes and facilitates persistence in the arthropod by potentiating an Nrf2-regulated antioxidant environment. IMPORTANCE: Recent advances demonstrate that the tick immune system recognizes and limits the pathogens they transmit. Innate immune mediators such as antimicrobial peptides and reactive oxygen/nitrogen species are produced and restrict microbial survival. It is currently unclear how pathogens remain in the tick, despite this immune assault. We found that an antioxidant response controlled by the PERK branch of the unfolded protein response is activated in ticks that are persistently infected with Borrelia burgdorferi (Lyme disease) or Anaplasma phagocytophilum (granulocytic anaplasmosis). The PERK pathway induces the antioxidant response transcription factor, Nrf2, which coordinates a gene network that ultimately neutralizes reactive oxygen and nitrogen species. Interfering with this signaling cascade in ticks causes a significant decline in pathogen numbers. Given that innate immune products can cause collateral damage to host tissues, we speculate that this is an arthropod-driven response aimed at minimizing damage to “self” that also inadvertently benefits the pathogen. Collectively, our findings shed light on the mechanistic push and pull between tick immunity and pathogen persistence within the arthropod vector.

Overview

The claims and statistics of this paper haven’t been checked yet.

Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.

A few free checks a day · papers already verified open instantly · results are public

Integrity signals

Registry

Crossref · 10.1128/msphere.00321-23

Cites

2 of 2 references verified0 citation errors · 0 not checkable

Statistics

Figures

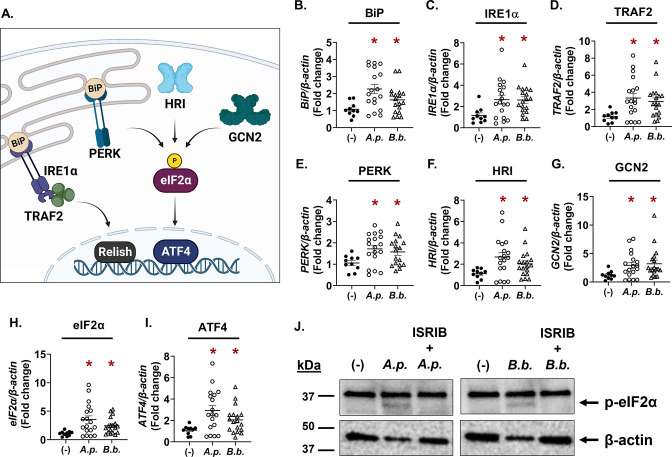
FIG 1 Tick-borne pathogens induce eIF2α-regulated stress responses in infected, unfed nymphs. (A) Graphic representation of IRE1α-TRAF2 signaling and the integrated stress response pathways in Ixodes ticks. (B–I) Gene expression in flat, unfed I. scapularis nymphs that are either uninfected (−), A. phagocytophilum-infected (A.p.), or B. burgdorferi-infected (B.b.). Each data point is representative of one nymph. Gene expression was quantified by qRT-PCR using primers listed in Table S1. Student’s t-test. *P < 0.05. (J) Phosphorylated eIF2α (36 kDa) immunoblot against ISE6 tick cells that were either uninfected (−), infected for 24 h (MOI 50), or treated with the eIF2α phosphorylation inhibitor ISRIB for 1 h prior to infection (24 h). β-Actin was probed as an internal loading control (45 kDa). Immunoblots are representative of two biological replicates. See also Fig. S1. A.p., A. phagocytophilum; B.b., B. burgdorferi; ISRIB, integrated stress response inhibitor.
FIG 1 Tick-borne pathogens induce eIF2α-regulated stress responses in infected, unfed nymphs. (A) Graphic representation of IRE1α-TRAF2 signaling and the integrated stress response pathways in Ixodes ticks. (B–I) Gene expression in flat, unfed I. scapularis nymphs that are either uninfected (−), A. phagocytophilum-infected (A.p.), or B. burgdorferi-infected (B.b.). Each data point is representative of one nymph. Gene expression was quantified by qRT-PCR using primers listed in Table S1. Student’s t-test. *P < 0.05. (J) Phosphorylated eIF2α (36 kDa) immunoblot against ISE6 tick cells that were either uninfected (−), infected for 24 h (MOI 50), or treated with the eIF2α phosphorylation inhibitor ISRIB for 1 h prior to infection (24 h). β-Actin was probed as an internal loading control (45 kDa). Immunoblots are representative of two biological replicates. See also Fig. S1. A.p., A. phagocytophilum; B.b., B. burgdorferi; ISRIB, integrated stress response inhibitor.CC BY · PubMed Central
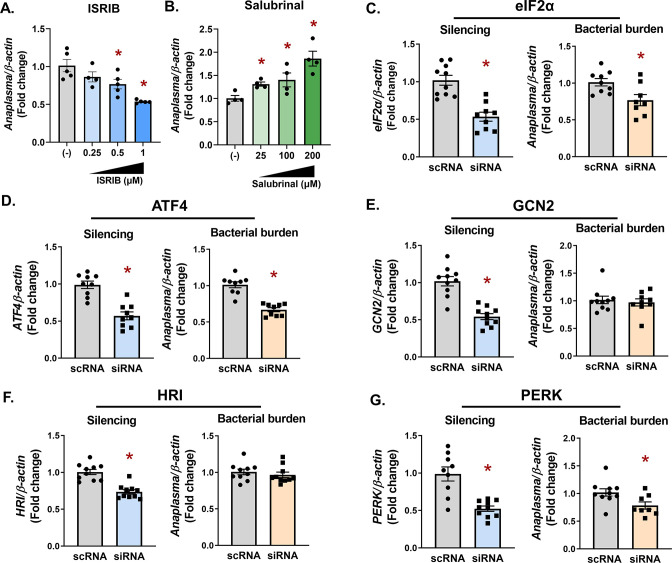
FIG 2 The PERK-eIF2α-ATF4 axis promotes A. phagocytophilum infection in tick cells. (A and B) ISE6 tick cells (1 × 10⁶) were pretreated with ISRIB (A) or salubrinal (B) at the indicated concentrations for 1 h prior to infection with A. phagocytophilum for 18 h (MOI 50). (C–G) IDE12 tick cells (1 × 10⁶) were treated with silencing RNAs (siRNAS) against indicated genes or scRNA controls for 24 h prior to infection with A. phagocytophilum (MOI 50) for 18 h. A. phagocytophilum burden and gene silencing for eIF2α (C), ATF4 (D), GCN2 (E), HRI (F), and PERK (G) were measured by qRT-PCR. Data are representative of at least five biological replicates with at least two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Student’s t-test). scRNA, scrambled RNA; siRNA, small interfering RNA.
FIG 2 The PERK-eIF2α-ATF4 axis promotes A. phagocytophilum infection in tick cells. (A and B) ISE6 tick cells (1 × 10⁶) were pretreated with ISRIB (A) or salubrinal (B) at the indicated concentrations for 1 h prior to infection with A. phagocytophilum for 18 h (MOI 50). (C–G) IDE12 tick cells (1 × 10⁶) were treated with silencing RNAs (siRNAS) against indicated genes or scRNA controls for 24 h prior to infection with A. phagocytophilum (MOI 50) for 18 h. A. phagocytophilum burden and gene silencing for eIF2α (C), ATF4 (D), GCN2 (E), HRI (F), and PERK (G) were measured by qRT-PCR. Data are representative of at least five biological replicates with at least two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Student’s t-test). scRNA, scrambled RNA; siRNA, small interfering RNA.CC BY · PubMed Central
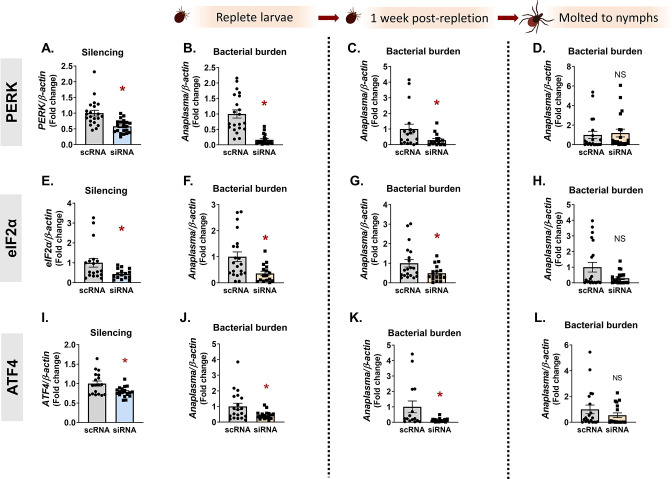
FIG 3 The PERK pathway supports A. phagocytophilum in vivo. I. scapularis larvae were immersed overnight in siRNA targeting PERK (A–D), eIF2α (E–H), or ATF4 (I–L) and fed on A. phagocytophilum-infected mice. Silencing efficiency (A, E, and I) and bacterial burden were assessed at three time intervals by qRT-PCR: immediately following repletion (B, F, and J), 1 week post-repletion (C, G, and K), and after ticks molted to nymphs (D, H, and L). Data are representative of 10–20 ticks and at least two experimental replicates. Each point represents one tick, with two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Mann-Whitney test). NS, non-significant; scRNA, scrambled RNA, siRNA, small interfering RNA.
FIG 3 The PERK pathway supports A. phagocytophilum in vivo. I. scapularis larvae were immersed overnight in siRNA targeting PERK (A–D), eIF2α (E–H), or ATF4 (I–L) and fed on A. phagocytophilum-infected mice. Silencing efficiency (A, E, and I) and bacterial burden were assessed at three time intervals by qRT-PCR: immediately following repletion (B, F, and J), 1 week post-repletion (C, G, and K), and after ticks molted to nymphs (D, H, and L). Data are representative of 10–20 ticks and at least two experimental replicates. Each point represents one tick, with two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Mann-Whitney test). NS, non-significant; scRNA, scrambled RNA, siRNA, small interfering RNA.CC BY · PubMed Central
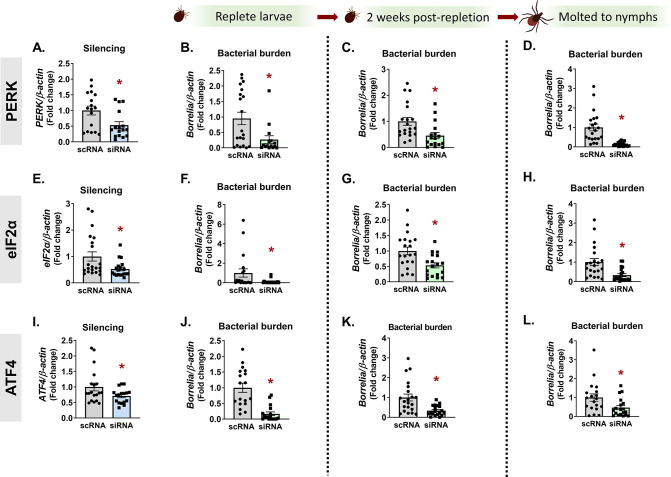
Fig 4 In vivo B. burgdorferi colonization and persistence through the molt is supported by the PERK pathway. PERK (A–D), eIF2α (E–H), or ATF4 (I–L) were silenced in I. scapularis larvae by immersing ticks in siRNA overnight. Recovered ticks were fed on B. burgdorferi-infected mice. Silencing efficiency (A, E, and I) and bacterial burden were assessed at three time intervals by qRT-PCR: immediately following repletion (B, F, and J), 2 weeks post-repletion (C, G, and K), and after ticks molted to nymphs (D, H, and L). Data are representative of 10–20 ticks and at least two experimental replicates. Each point represents one tick, with two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Mann-Whitney test). scRNA, scrambled RNA, siRNA, small interfering RNA.
Fig 4 In vivo B. burgdorferi colonization and persistence through the molt is supported by the PERK pathway. PERK (A–D), eIF2α (E–H), or ATF4 (I–L) were silenced in I. scapularis larvae by immersing ticks in siRNA overnight. Recovered ticks were fed on B. burgdorferi-infected mice. Silencing efficiency (A, E, and I) and bacterial burden were assessed at three time intervals by qRT-PCR: immediately following repletion (B, F, and J), 2 weeks post-repletion (C, G, and K), and after ticks molted to nymphs (D, H, and L). Data are representative of 10–20 ticks and at least two experimental replicates. Each point represents one tick, with two technical replicates. Error bars show standard error of the mean. *P < 0.05 (Mann-Whitney test). scRNA, scrambled RNA, siRNA, small interfering RNA.CC BY · PubMed Central
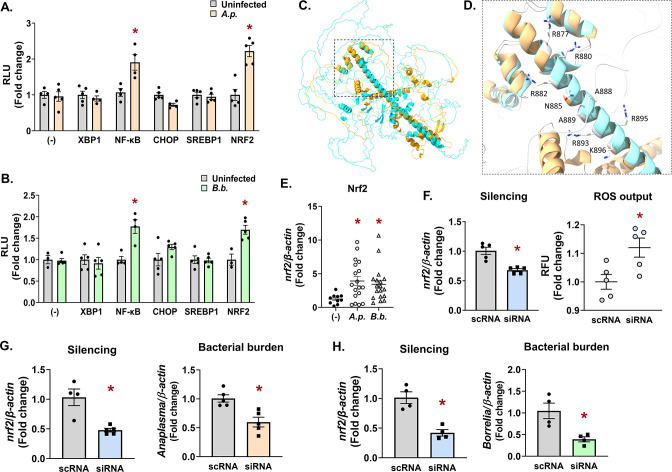
Fig 5 Infection triggers an Nrf2-regulated antioxidant response in ticks that promotes pathogen survival. (A and B) HEK293T cells (1 × 10⁴) were transfected with luciferase reporter vectors for assaying activity of ER stress transcription factors XBP1, NF-κB, CHOP, SREBP1, and NRF2 or were untransfected (−). Cells were then infected with A.p. (A) or B.b. (B). After 24 h, D-luciferin was added and luminescence was measured as RLU. Measurements were normalized to uninfected controls (gray bars). Luciferase assays are representative of three to five biological replicates with at least two experimental replicates ± SEM. Student’s t-test. *P < 0.05. (C and D) Predicted Ixodes Nrf2 structure modeled with AlphaFold (46, 47) (blue) and overlaid with human Nrf2 (orange) using UCSF ChimeraX.(48) The bZIP domain is indicated by a box with dashed lines. (D) Magnified region of the bZIP domain depicting residues that that are predicted to interact with antioxidant response element sequences in DNA promoter regions (R877, R880, R882, N885, A888, A889, R893, R895, and K896). See also Fig. S2. (E) Nrf2 expression levels in flat, unfed nymphs that are uninfected (−), A.p.-infected, or B.b.-infected. Each data point is representative of one nymph. Gene expression was quantified by qRT-PCR using Nrf2 primers listed in Table S1. Student’s t-test. *P < 0.05. (F–H) IDE12 tick cells were treated with silencing RNAs (siRNA) targeting nrf2 for 24 h prior to infection with A. phagocytophilum (18 h) (F and G) or B. burgdorferi (H). Gene silencing (F–H) and bacterial burden (G and H) were quantified by qRT-PCR. ROS was measured as relative fluorescent units after 24 h of infection (F). Data are representative of at least four to five biological replicates and two technical replicates. Error bars show SEM, *P < 0.05 (Student’s t-test). bZIP, basic leucine zipper; RLU, relative luminescence unit; scRNA, scrambled RNA; SEM, standard error of the mean; siRNA, small interfering RNA.
Fig 5 Infection triggers an Nrf2-regulated antioxidant response in ticks that promotes pathogen survival. (A and B) HEK293T cells (1 × 10⁴) were transfected with luciferase reporter vectors for assaying activity of ER stress transcription factors XBP1, NF-κB, CHOP, SREBP1, and NRF2 or were untransfected (−). Cells were then infected with A.p. (A) or B.b. (B). After 24 h, D-luciferin was added and luminescence was measured as RLU. Measurements were normalized to uninfected controls (gray bars). Luciferase assays are representative of three to five biological replicates with at least two experimental replicates ± SEM. Student’s t-test. *P < 0.05. (C and D) Predicted Ixodes Nrf2 structure modeled with AlphaFold (46, 47) (blue) and overlaid with human Nrf2 (orange) using UCSF ChimeraX.(48) The bZIP domain is indicated by a box with dashed lines. (D) Magnified region of the bZIP domain depicting residues that that are predicted to interact with antioxidant response element sequences in DNA promoter regions (R877, R880, R882, N885, A888, A889, R893, R895, and K896). See also Fig. S2. (E) Nrf2 expression levels in flat, unfed nymphs that are uninfected (−), A.p.-infected, or B.b.-infected. Each data point is representative of one nymph. Gene expression was quantified by qRT-PCR using Nrf2 primers listed in Table S1. Student’s t-test. *P < 0.05. (F–H) IDE12 tick cells were treated with silencing RNAs (siRNA) targeting nrf2 for 24 h prior to infection with A. phagocytophilum (18 h) (F and G) or B. burgdorferi (H). Gene silencing (F–H) and bacterial burden (G and H) were quantified by qRT-PCR. ROS was measured as relative fluorescent units after 24 h of infection (F). Data are representative of at least four to five biological replicates and two technical replicates. Error bars show SEM, *P < 0.05 (Student’s t-test). bZIP, basic leucine zipper; RLU, relative luminescence unit; scRNA, scrambled RNA; SEM, standard error of the mean; siRNA, small interfering RNA.CC BY · PubMed Central
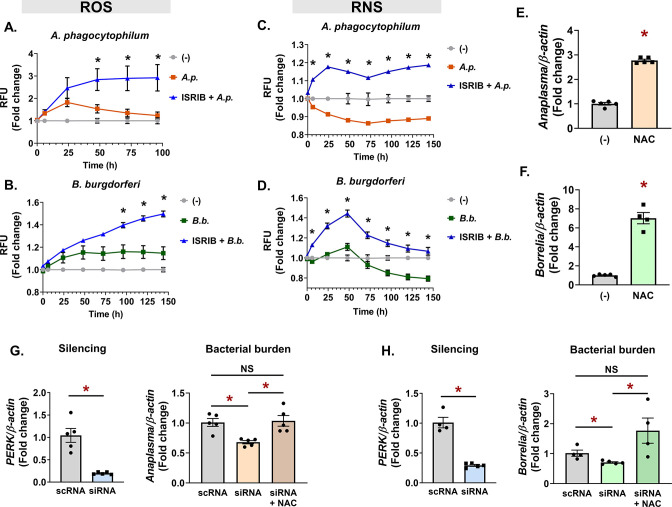
Fig 6 Antioxidant activity of the PERK-eIF2α pathway protects pathogens in ticks. (A–D) ROS (A and B) and RNS (C and D) measurements in ISE6 cells (1.68 × 10⁵) untreated (-), infected (A.p. or B.b.), or pretreated with 1-µM ISRIB prior to infection with A. phagocytophilum (ISRIB + A.p.) (A and C) or B. burgdorferi (ISRIB + B.b.) (B and D). Fluorescence was measured at the indicated time points and is presented as RFU, normalized to untreated, uninfected controls (−). See also Fig. S3A and B. (E and F) IDE12 cells were infected with A. phagocytophilum (E) or B. burgdorferi (F) alone or in the presence of NAC for 24 h. (G and H) perk was silenced in IDE12 cells (1 × 10⁶). Cells were infected with A. phagocytophilum (G) or B. burgdorferi (H) alone or in the presence of NAC. See also Fig. S4A and B. Silencing levels and bacterial burdens were quantified by qRT-PCR. Data are representative of at least four to five biological replicates and two technical replicates. Error bars show SEM. *P < 0.05 (Student’s t-test). NAC, N-acetyl cysteine; RFU, relative fluorescent unit; scRNA, scrambled RNA; siRNA, small interfering RNA.
Fig 6 Antioxidant activity of the PERK-eIF2α pathway protects pathogens in ticks. (A–D) ROS (A and B) and RNS (C and D) measurements in ISE6 cells (1.68 × 10⁵) untreated (-), infected (A.p. or B.b.), or pretreated with 1-µM ISRIB prior to infection with A. phagocytophilum (ISRIB + A.p.) (A and C) or B. burgdorferi (ISRIB + B.b.) (B and D). Fluorescence was measured at the indicated time points and is presented as RFU, normalized to untreated, uninfected controls (−). See also Fig. S3A and B. (E and F) IDE12 cells were infected with A. phagocytophilum (E) or B. burgdorferi (F) alone or in the presence of NAC for 24 h. (G and H) perk was silenced in IDE12 cells (1 × 10⁶). Cells were infected with A. phagocytophilum (G) or B. burgdorferi (H) alone or in the presence of NAC. See also Fig. S4A and B. Silencing levels and bacterial burdens were quantified by qRT-PCR. Data are representative of at least four to five biological replicates and two technical replicates. Error bars show SEM. *P < 0.05 (Student’s t-test). NAC, N-acetyl cysteine; RFU, relative fluorescent unit; scRNA, scrambled RNA; siRNA, small interfering RNA.CC BY · PubMed Central
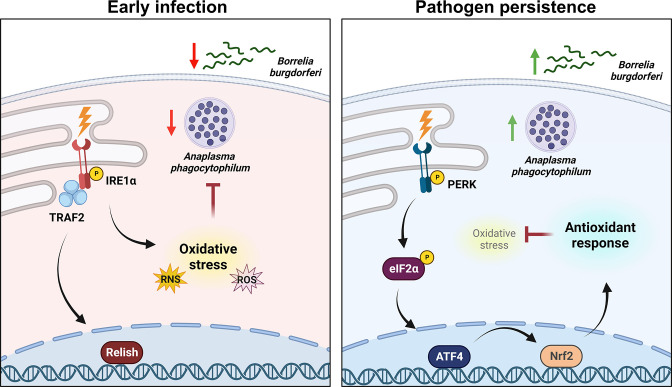
Fig 7 The PERK-eIF2α-ATF4 axis promotes pathogen survival in ticks through an Nrf2-mediated antioxidant response. When colonizing the tick, A. phagocytophilum and B. burgdorferi trigger the Ixodes IMD pathway and ROS/RNS through the IRE1α-TRAF2 axis of the UPR. Tick-borne microbes persist in the tick over time by stimulating the PERK branch of the UPR, which signals through eIF2α and the transcription factors ATF4 and Nrf2 to trigger an antioxidant response that promotes microbial survival.
Fig 7 The PERK-eIF2α-ATF4 axis promotes pathogen survival in ticks through an Nrf2-mediated antioxidant response. When colonizing the tick, A. phagocytophilum and B. burgdorferi trigger the Ixodes IMD pathway and ROS/RNS through the IRE1α-TRAF2 axis of the UPR. Tick-borne microbes persist in the tick over time by stimulating the PERK branch of the UPR, which signals through eIF2α and the transcription factors ATF4 and Nrf2 to trigger an antioxidant response that promotes microbial survival.CC BY · PubMed Central

Verification

Claims the paper makes

The claims and statistics of this paper haven’t been checked yet.

Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.

A few free checks a day · papers already verified open instantly · results are public

Self-check

Percentages, sums and reported differences re-computed from the paper’s own numbers.

The self-check needs the paper’s full text.

Citations

Cites

Show all 2 references

Research works printed but not linked: 104

  1. Paddock CD , Lane RS , Staples JE , Labruna MB . 2016. Changing paradigms for tick-borne diseases in the Americas. In Global health impacts of vector-borne diseases: workshop summary. National Academies Press (US), Washington (DC).
  2. 10.17226/13134 · DOI
  3. 10.1017/s0031182004005967 · DOI
  4. 10.3389/fcimb.2021.739419 · DOI
  5. 10.3389/fimmu.2023.1094326 · DOI
  6. 10.1038/embor.2011.177 · DOI
  7. 10.1603/0022-2585-38.1.99 · DOI
  8. 10.1016/s0145-305x(96)00023-7 · DOI
  9. 10.1038/ncomms14401 · DOI
  10. 10.1073/pnas.1808905116 · DOI
  11. 10.1016/j.dci.2015.12.018 · DOI
  12. 10.3389/fcimb.2014.00116 · DOI
  13. 10.1093/infdis/jis484 · DOI
  14. 10.1016/j.chom.2016.06.001 · DOI
  15. 10.1126/science.abl3837 · DOI
  16. 10.1073/pnas.2208673120 · DOI
  17. 10.1038/ncomms10507 · DOI
  18. 10.1093/molbev/msv093 · DOI
  19. 10.1128/mbio.02922-22 · DOI
  20. 10.3389/fimmu.2020.629777 · DOI
  21. 10.1038/nri.2016.62 · DOI
  22. 10.1038/nrm3270 · DOI
  23. 10.1146/annurev.biochem.73.011303.074134 · DOI
  24. 10.1086/322044 · DOI
  25. 10.15252/embr.201642195 · DOI · Paper page
  26. 10.1016/s1097-2765(03)00105-9 · DOI
  27. 10.1038/srep32886 · DOI
  28. 10.1007/s00018-012-1252-6 · DOI
  29. 10.1038/sj.emboj.7600596 · DOI
  30. 10.1038/ncb2738 · DOI · Paper page
  31. 10.7554/eLife.05033 · DOI
  32. 10.1016/j.bmcl.2005.05.120 · DOI
  33. 10.1126/science.1101902 · DOI
  34. 10.1128/JCM.36.12.3574-3578.1998 · DOI
  35. 10.1073/pnas.1613422114 · DOI
  36. 10.1016/j.chom.2013.12.001 · DOI
  37. 10.1038/s41467-017-00208-0 · DOI
  38. 10.4269/ajtmh.1990.42.352 · DOI
  39. 10.21775/cimb.042.113 · DOI
  40. 10.1186/1471-2164-9-552 · DOI
  41. 10.4049/jimmunol.158.7.3285 · DOI
  42. 10.1016/j.ygeno.2008.05.005 · DOI
  43. 10.3389/fpubh.2020.558283 · DOI
  44. 10.1128/IAI.05219-11 · DOI
  45. 10.1093/nar/gkab1061 · DOI · Paper page
  46. 10.1002/pro.3943 · DOI
  47. 10.1073/pnas.91.21.9926 · DOI · Paper page
  48. 10.1016/j.tibs.2014.02.002 · DOI
  49. 10.3390/cancers12030569 · DOI
  50. 10.1074/jbc.M314219200 · DOI
  51. 10.1074/jbc.M101198200 · DOI
  52. 10.1006/bbrc.1997.6943 · DOI · Paper page
  53. 10.1016/S0021-9258(18)99004-6 · DOI · Paper page
  54. 10.1038/s41588-022-01275-w · DOI
  55. 10.1093/nar/gkac1102 · DOI
  56. 10.1111/j.1462-5822.2006.00835.x · DOI
  57. 10.1007/978-1-60327-032-8_17 · DOI
  58. 10.1111/j.1365-2958.2009.06951.x · DOI
  59. 10.1128/IAI.01018-09 · DOI
  60. 10.1128/IAI.68.12.6697-6703.2000 · DOI
  61. 10.1046/j.1462-5822.2003.00323.x · DOI
  62. 10.1128/IAI.72.8.4772-4783.2004 · DOI
  63. 10.1038/s41598-019-49766-x · DOI
  64. 10.1111/j.1365-2958.2008.06204.x · DOI
  65. 10.1371/journal.ppat.1006225 · DOI
  66. 10.3389/fmicb.2016.01397 · DOI
  67. 10.1111/j.1365-2958.2011.07691.x · DOI
  68. 10.1371/journal.pone.0084625 · DOI
  69. 10.1074/jbc.M113.538272 · DOI
  70. 10.1128/iai.62.9.3663-3671.1994 · DOI
  71. 10.1016/0165-2478(94)90185-6 · DOI
  72. 10.1016/j.chom.2007.06.001 · DOI
  73. Park JM Genera BM Fahy D Swallow KT Nelson CM Oliver JD Shaw DK Munderloh UG Brayton KA . 2023. An Anaplasma phagocytophilum T4SS effector AteA is essential for tick infection. bioRxiv:2023.02.06.527355. doi:10.1101/2023.02.06.527355 2023.02.06.527355 · DOI
  74. 10.1016/j.it.2018.09.003 · DOI
  75. 10.1016/j.bbrc.2012.01.037 · DOI
  76. 10.1186/1475-2840-12-158 · DOI
  77. 10.1074/mcp.M115.051938 · DOI
  78. 10.7554/eLife.86636 · DOI
  79. 10.1089/ars.2017.7342 · DOI
  80. 10.1038/nrd4002 · DOI · Paper page
  81. 10.1111/imb.12184 · DOI
  82. 10.1111/imb.12304 · DOI
  83. 10.1186/s13071-019-3548-y · DOI
  84. 10.1016/j.actatropica.2020.105763 · DOI
  85. 10.1186/s13071-016-1579-1 · DOI
  86. 10.1371/journal.pone.0082012 · DOI
  87. 10.1186/1471-213X-9-42 · DOI
  88. 10.1111/imb.12218 · DOI
  89. 10.1186/s13071-017-2575-9 · DOI
  90. 10.1186/s40168-018-0524-2 · DOI
  91. 10.1016/j.celrep.2020.108317 · DOI
  92. 10.7554/eLife.12318 · DOI
  93. 10.1126/science.1214935 · DOI · Paper page
  94. 10.1146/annurev-immunol-020711-075030 · DOI · Paper page
  95. 10.1016/j.meegid.2018.03.023 · DOI
  96. 10.3389/fgene.2019.01266 · DOI
  97. 10.1111/j.1574-695X.2012.01001.x · DOI
  98. 10.4049/jimmunol.179.7.4783 · DOI
  99. 10.1128/IAI.69.1.446-455.2001 · DOI
  100. 10.1371/journal.pone.0155798 · DOI
  101. 10.1111/j.1365-2958.2007.05895.x · DOI
  102. 10.1093/infdis/jit380 · DOI
  103. 10.1016/j.chom.2018.10.005 · DOI · Paper page
  104. 10.1093/bioinformatics/btp033 · DOI

Metadata

Authors
Rosche, K. L., Hurtado, J., Fisk, E. A., Vosbigian, K. A., Warren, A. L., Sidak-Loftis, L. C., Wright, S. J., Ramirez-Zepp, E., Park, J. M., & Shaw, D. K.
Affiliations
  • Washington State University (US)
  • Department of Veterinary Microbiology and Pathology, Washington State University , Pullman, Washington, USA
Corresponding author
Shaw, Dana K.
Venue
mSphere
Published
2023-10-24
Volume
8
Issue
5
Pages
e0032123-e0032123
ISSN
2379-5042 (ISSN-L)
OpenAlex
W4386910548
Cited by
10
References
2
Citations by year
2026: 4 · 2025: 6
FWCI
2.35
Type
journal article
Language
en
Open access
Locations
  • mSphere (publishedVersion, cc-by)
  • bioRxiv (Cold Spring Harbor Laboratory) (acceptedVersion, cc-by-nc-nd)
  • PubMed Central (publishedVersion, cc-by)
  • PubMed (publishedVersion)
  • PubMed Central (submittedVersion, cc-by-nc-nd)
  • DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion, cc-by-sa)
Funders
  • HHS | NIH | National Institute of Allergy and Infectious Diseases (R21AI148578, R21AI139772, R01AI162819, T32GM008336, T32AI007025)
  • HHS | NIH | National Institute of Biomedical Imaging and Bioengineering (R25EB027606)
Topics
  • Life Sciences › Immunology and Microbiology › Parasitology › Vector-borne infectious diseases
  • Life Sciences › Immunology and Microbiology › Immunology › Invertebrate Immune Response Mechanisms
  • Life Sciences › Agricultural and Biological Sciences › Insect Science › Insect symbiosis and bacterial influences
Keywords
PERK signaling, unfolded protein response, tick immunity, Borrelia burgdorferi, Anaplasma phagocytophilum, Nrf2, antioxidant response, reactive oxygen species, reactive nitrogen species, Ixodes scapularis, tick-borne pathogens, eIF2α, tick innate immunity, Lyme disease, human granulocytic anaplasmosis

About these checks

Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.

Statistics and arithmetic are recomputed, not judged.

Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.

What counts as a claim ›How we measure confidence ›How we check this ›

Are you an author, or do you see a problem with this page? Request a review

How to cite

Cite CoChat for the checks on this page, and the paper for its own findings.

This page
CoChat. (2026). Citation check: PERK-mediated antioxidant response is key for pathogen persistence in ticks. https://app.cochat.ai/papers/10.1128/msphere.00321-23
The paper
Rosche, K. L., Hurtado, J., Fisk, E. A., Vosbigian, K. A., Warren, A. L., Sidak-Loftis, L. C., Wright, S. J., Ramirez-Zepp, E., Park, J. M., & Shaw, D. K. (2023). PERK-mediated antioxidant response is key for pathogen persistence in ticks. mSphere. https://doi.org/10.1128/msphere.00321-23