

The DOI matches its Crossref record; 57 of the 58 references it cites were found in a registry or an index.
RNAs Containing Modified Nucleotides Fail To Trigger RIG-I Conformational Changes for Innate Immune Signaling
Open accessAbstract
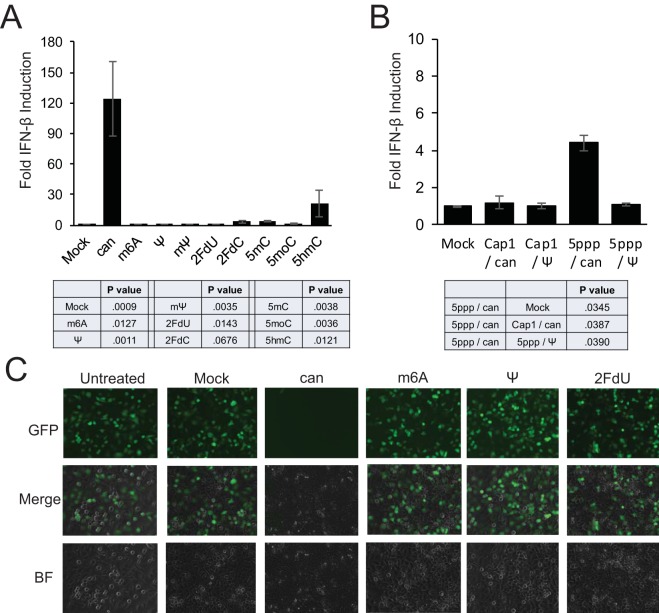
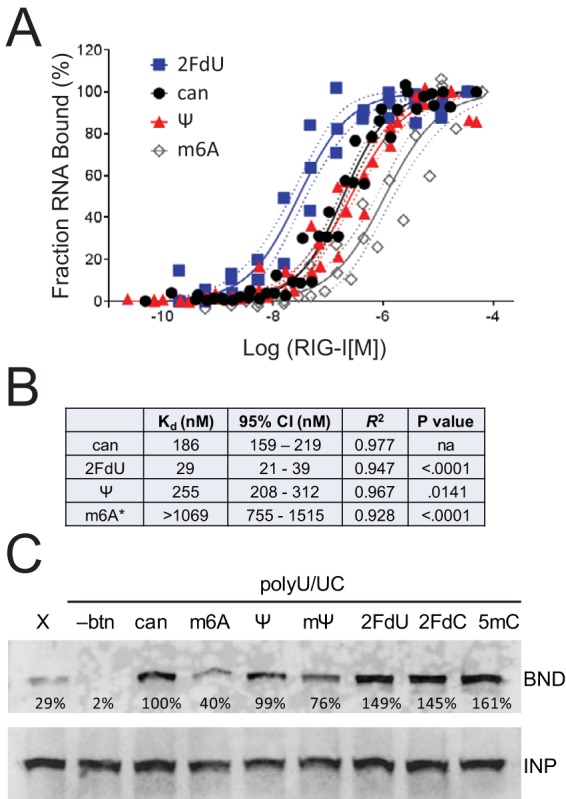
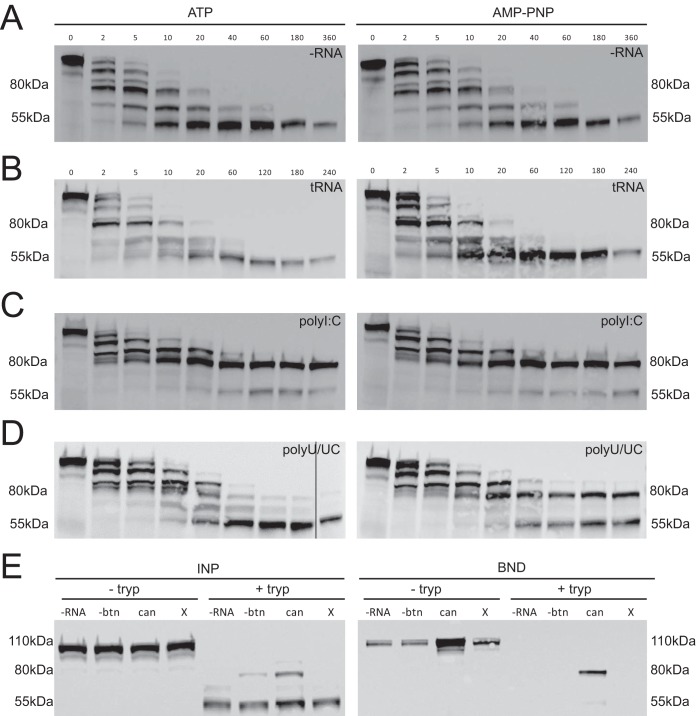
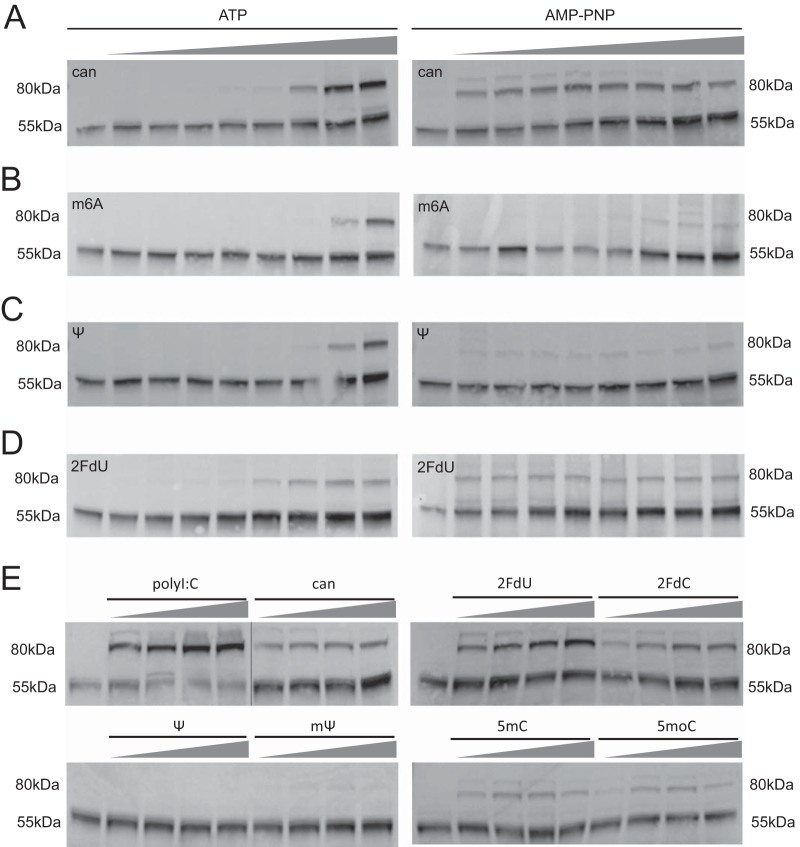
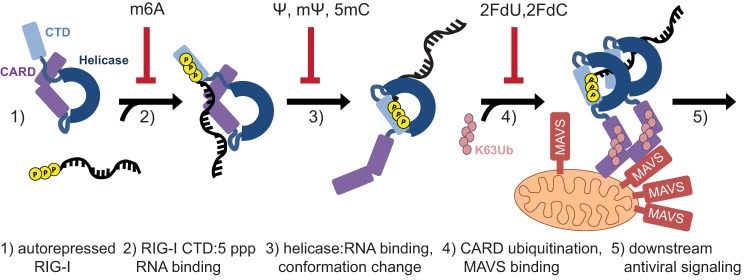
UNLABELLED: Invading pathogen nucleic acids are recognized and bound by cytoplasmic (retinoic acid-inducible gene I [RIG-I]-like) and membrane-bound (Toll-like) pattern recognition receptors to activate innate immune signaling. Modified nucleotides, when present in RNA molecules, diminish the magnitude of these signaling responses. However, mechanisms explaining the blunted signaling have not been elucidated. In this study, we used several independent biological assays, including inhibition of virus replication, RIG-I:RNA binding assays, and limited trypsin digestion of RIG-I:RNA complexes, to begin to understand how RNAs containing modified nucleotides avoid or suppress innate immune signaling. The experiments were based on a model innate immune activating RNA molecule, the polyU/UC RNA domain of hepatitis C virus, which was transcribed in vitro with canonical nucleotides or with one of eight modified nucleotides. The approach revealed signature assay responses associated with individual modified nucleotides or classes of modified nucleotides. For example, while both N-6-methyladenosine (m6A) and pseudouridine nucleotides correlate with diminished signaling, RNA containing m6A modifications bound RIG-I poorly, while RNA containing pseudouridine bound RIG-I with high affinity but failed to trigger the canonical RIG-I conformational changes associated with robust signaling. These data advance understanding of RNA-mediated innate immune signaling, with additional relevance for applying nucleotide modifications to RNA therapeutics. IMPORTANCE: The innate immune system provides the first response to virus infections and must distinguish between host and pathogen nucleic acids to mount a protective immune response without activating autoimmune responses. While the presence of nucleotide modifications in RNA is known to correlate with diminished innate immune signaling, the underlying mechanisms have not been explored. The data reported here are important for defining mechanistic details to explain signaling suppression by RNAs containing modified nucleotides. The results suggest that RNAs containing modified nucleotides interrupt signaling at early steps of the RIG-I-like innate immune activation pathway and also that nucleotide modifications with similar chemical structures can be organized into classes that suppress or evade innate immune signaling steps. These data contribute to defining the molecular basis for innate immune signaling suppression by RNAs containing modified nucleotides. The results have important implications for designing therapeutic RNAs that evade innate immune detection.
Overview
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Run the check — free, no account needed. It reads the open-access text and checks the sources it cites.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
In the citing paper
“by incorporating naturally occurring modified nucleotides into the IVT mRNA, its innate immune activity could be drastically reduced [6,7]”
From The dawn of mRNA vaccines: the COVID-19 case (2021) · cites this paper as [7]
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
Karikó, K., Buckstein, M., Ni, H., & Weissman, D. (2005) · Immunity · doi:10.1016/j.immuni.2005.06.008 · Cited by 2,728
Warren, L., Manos, P. D., Ahfeldt, T., Loh, Y.-H., Li, H., Lau, F., Ebina, W., Mandal, P. K., Smith, Z. D., Meissner, A., et al. (2010) · Cell Stem Cell · doi:10.1016/j.stem.2010.08.012 · Cited by 2,662
5'-Triphosphate RNA Is the Ligand for RIG-I
Hornung, V., Ellegast, J., Kim, S., Brzózka, K., Jung, A., Kato, H., Poeck, H., Akira, S., Conzelmann, K.-K., Schlee, M., et al. (2006) · Science · doi:10.1126/science.1132505 · Cited by 2,474
RIG-I-mediated antiviral responses to single-stranded RNA bearing 5’-phosphates
Pichlmair, A., Schulz, O., Tan, C. P., Näslund, T. I., Liljeström, P., Weber, F., & Reis e Sousa, C. (2006) · Science · doi:10.1126/science.1132998 · Cited by 2,210
TRIM25 RING-finger E3 ubiquitin ligase is essential for RIG-I-mediated antiviral activity
Gack, M. U., Shin, Y. C., Joo, C.-H., Urano, T., Liang, C., Sun, L., Takeuchi, O., Akira, S., Chen, Z. J., Inoue, S., et al. (2007) · Nature · doi:10.1038/nature05732 · Cited by 1,683
Widespread occurrence of 5-methylcytosine in human coding and non-coding RNA
Squires, J. E., Patel, H. R., Nousch, M., Sibbritt, T., Humphreys, D. T., Parker, B. J., Suter, C. M., & Preiß, T. (2012) · Nucleic Acids Research · doi:10.1093/nar/gks144 · Cited by 1,033
MODOMICS: a database of RNA modification pathways—2013 update
Machnicka, M. A., Milanowska, K., Oglou, O. O., Purta, E., Kurkowska, M., Olchowik, A., Januszewski, W., Kalinowski, S., Dunin-Horkawicz, S., Rother, K. M., et al. (2012) · Nucleic Acids Research · doi:10.1093/nar/gks1007 · Cited by 1,003
2′-O methylation of the viral mRNA cap evades host restriction by IFIT family members
Daffis, S., Szretter, K. J., Schriewer, J. M., Li, J., Youn, S., Errett, J. S., Lin, T., Schneller, S. W., Züst, R., Dong, H., et al. (2010) · Nature · doi:10.1038/nature09489 · Cited by 910
Sumpter, R., Loo, Y., Foy, E. M., Li, K., Yoneyama, M., Fujita, T., Lemon, S. M., & Gale, M. (2005) · Journal of Virology · doi:10.1128/jvi.79.5.2689-2699.2005 · Cited by 900
Karikó, K., Muramatsu, H., Ludwig, J., & Weissman, D. (2011) · Nucleic Acids Research · doi:10.1093/nar/gkr695 · Cited by 898
Research works printed but not linked: 1
- 10.3791/51415:e51415 · DOI
Cited by
Sorted by citations
N6-Methyladenosine Modification Controls Circular RNA Immunity
Chen, Y. G., Chen, R., Ahmad, S., Verma, R., Kasturi, S. P., Amaya, L., Broughton, J. P., Kim, J., Cadena, C., Pulendran, B., et al. (2019) · Molecular Cell · doi:10.1016/j.molcel.2019.07.016 · Cited by 578
Innate immune mechanisms of mRNA vaccines
Verbeke, R., Hogan, M. J., Loré, K., & Pardi, N. (2022) · Immunity · doi:10.1016/j.immuni.2022.10.014 · Cited by 535
The dawn of mRNA vaccines: the COVID-19 case
Verbeke, R., Lentacker, I., De Smedt, S. C., & Dewitte, H. (2021) · Journal of Controlled Release · doi:10.1016/j.jconrel.2021.03.043 · Cited by 504
Mettl3-mediated mRNA m6A methylation promotes dendritic cell activation
Wang, H., Hu, X., Huang, M., Liu, J., Gu, Y. H., Ma, L., Zhou, Q., & Cao, X. (2019) · Nature Communications · doi:10.1038/s41467-019-09903-6 · Cited by 507
RNA Circularization Diminishes Immunogenicity and Can Extend Translation Duration In Vivo
Wesselhoeft, R. A., Kowalski, P. S., Parker-Hale, F. C., Huang, Y., Bisaria, N., & Anderson, D. G. (2019) · Molecular Cell · doi:10.1016/j.molcel.2019.02.015 · Cited by 482
Metadata
- Authors
- Durbin, A. F., Wang, C., Marcotrigiano, J., & Gehrke, L.
- Affiliations
- Harvard University (US)
- Rutgers, The State University of New Jersey (US)
- Corresponding author
- Gehrke, Lee
- Venue
- mBio
- Publisher
- American Society for Microbiology
- Published
- 2016-11-02
- Volume
- 7
- Issue
- 5
- ISSN
- 2150-7511 (ISSN-L)
- 2161-2129
- PMC
- PMC5030355
- OpenAlex
- W2522303658
- Cited by
- 238
- References
- 58
- Citations by year
- 2026: 13 · 2025: 22 · 2024: 25 · 2023: 27 · 2022: 28 · 2021: 49 · 2020: 30 · 2019: 23 · 2018: 13 · 2017: 8
- FWCI
- 8.88
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Licence
- Locations
- mBio (publishedVersion, cc-by)
- Europe PMC (PubMed Central) (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- Digital Access to Scholarship at Harvard (DASH) (Harvard University) (submittedVersion, cc-by)
- DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion, cc-by-sa)
- DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion)
- DSpace@MIT (Massachusetts Institute of Technology) (submittedVersion, cc-by-nc)
- Funders
- HHS | U.S. Public Health Service (CA159132, AI100190)
- Topics
- Life Sciences › Immunology and Microbiology › Immunology › interferon and immune responses
- Life Sciences › Immunology and Microbiology › Immunology › Immune Response and Inflammation
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › RNA regulation and disease
- Keywords
- RIG-I, modified nucleotides, innate immune signaling, pseudouridine, RNA conformational change, RNA therapeutics, immune evasion, viral RNA recognition
- MeSH terms
- DEAD Box Protein 58, Cell Line, Humans, Immunity, Innate, Models, Molecular, Ribonucleosides, RNA, Viral, Signal Transduction, Hepacivirus, Interferon-beta
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
