

DNA Specificity Determinants Associate with Distinct Transcription Factor Functions
Open accessThe DOI matches its Crossref record; 53 of the 53 references it cites were found in a registry or an index.
Abstract
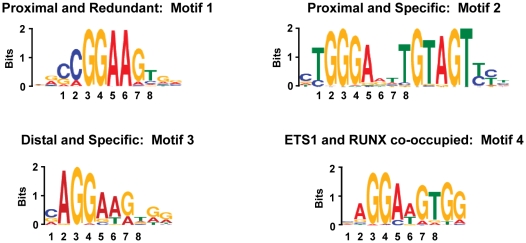
To elucidate how genomic sequences build transcriptional control networks, we need to understand the connection between DNA sequence and transcription factor binding and function. Binding predictions based solely on consensus predictions are limited, because a single factor can use degenerate sequence motifs and because related transcription factors often prefer identical sequences. The ETS family transcription factor, ETS1, exemplifies these challenges. Unexpected, redundant occupancy of ETS1 and other ETS proteins is observed at promoters of housekeeping genes in T cells due to common sequence preferences and the presence of strong consensus motifs. However, ETS1 exhibits a specific function in T cell activation; thus, unique transcriptional targets are predicted. To uncover the sequence motifs that mediate specific functions of ETS1, a genome-wide approach, chromatin immunoprecipitation coupled with high-throughput sequencing (ChIP-seq), identified both promoter and enhancer binding events in Jurkat T cells. A comparison with DNase I sensitivity both validated the dataset and also improved accuracy. Redundant occupancy of ETS1 with the ETS protein GABPA occurred primarily in promoters of housekeeping genes, whereas ETS1 specific occupancy occurred in the enhancers of T cell-specific genes. Two routes to ETS1 specificity were identified: an intrinsic preference of ETS1 for a variant of the ETS family consensus sequence and the presence of a composite sequence that can support cooperative binding with a RUNX transcription factor. Genome-wide occupancy of RUNX factors corroborated the importance of this partnership. Furthermore, genome-wide occupancy of co-activator CBP indicated tight co-localization with ETS1 at specific enhancers, but not redundant promoters. The distinct sequences associated with redundant versus specific ETS1 occupancy were predictive of promoter or enhancer location and the ontology of nearby genes. These findings demonstrate that diversity of DNA binding motifs may enable variable transcription factor function at different genomic sites.
Overview
The claims and statistics of this paper haven’t been checked yet.
Free: it reads the open-access text and checks the first 5 claims that cite a source we can check. Create a free account to check every claim.
Integrity signals
Registry
Cites
Statistics
Figures


Verification
Claims the paper makes
The claims and statistics of this paper haven’t been checked yet.
Free: it reads the open-access text and checks the first 5 claims that cite a source we can check. Create a free account to check every claim.
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
The cited source says what the claim attributes to it.
In the citing paper
“This selection would be necessary at enhancers, where ERG (62) and ETS1 specificity (65) is observed, but not at redundant promoter-binding sites where the ETS-binding sequence can be protected from DNA methylation as a result of proximity to, or inclusion in, hypomethylated CpG islands.”
From Genomic and biochemical insights into the specificity of ETS transcription factors (2011) · cites this paper as [65]
The cited source says what the claim attributes to it.
In the citing paper
“Thus, the ETS/RUNX sequence motif is predictive of the function of nearby genes (65).”
From Genomic and biochemical insights into the specificity of ETS transcription factors (2011) · cites this paper as [65]
In the citing paper
“Quantitative DNA-binding studies indicate that the affinity of different ETS proteins for the same consensus sequence many vary by only ~10-fold, whereas the affinity of the same protein for variant consensus sites differs by ~5- to 80-fold (53, 56, 65).”
From Genomic and biochemical insights into the specificity of ETS transcription factors (2011) · cites this paper as [65]
In the citing paper
“ERK2 phosphorylates Thr38, as well as a nonconsensus acceptor Ser41, within the unstructured N-terminal region of ETS1, immediately adjacent to its PNT domain.”
From Genomic and biochemical insights into the specificity of ETS transcription factors (2011) · cites this paper as [65]
In the citing paper
“The reported overlap for ETS1 and GABPA shows most GABPA-bound regions are also occupied by ETS1 in Jurkat cells (65, 136).”
From Genomic and biochemical insights into the specificity of ETS transcription factors (2011) · cites this paper as [65]
6 more claims about this paper
Create a free account to see every claim other papers make about this one.
Self-check
Percentages, sums and reported differences re-computed from the paper’s own numbers.
The self-check needs the paper’s full text.
Citations
Cites
DNA methylation patterns and epigenetic memory
Bird, A. (2002) · Genes & Development · doi:10.1101/gad.947102 · Cited by 7,124 · cited 1×
“. The CpG islands at housekeeping promoters are generally hypomethylated, whereas CpG dinucleotides distributed in lower density throughout the genome are likely to be methylated”
BackgroundHigh-Resolution Profiling of Histone Methylations in the Human Genome
Barski, A., Cuddapah, S., Cui, K., Roh, T.-Y., Schones, D. E., Wang, Z., Wei, G., Chepelev, I., & Zhao, K. (2007) · Cell · doi:10.1016/j.cell.2007.05.009 · Cited by 6,845
Fitting a mixture model by expectation maximization to discover motifs in biopolymers.
Bailey, T. L., & Elkan, C. (1994) · PubMed · Cited by 5,806
Heintzman, N. D., Stuart, R. K., Hon, G., Fu, Y., Ching, C. W., Hawkins, R. D., Barrera, L. O., Van Calcar, S., Qu, C., Ching, K. A., et al. (2007) · Nature Genetics · doi:10.1038/ng1966 · Cited by 3,398 · cited 4×
“p300 has a strong correlation with enhancers [21,30,46].”
BackgroundInfluentialGenome-scale DNA methylation maps of pluripotent and differentiated cells
Meissner, A., Mikkelsen, T. S., Gu, H., Wernig, M., Hanna, J., Sivachenko, A., Zhang, X., Bernstein, B. E., Nusbaum, C., Jaffe, D. B., et al. (2008) · Nature · doi:10.1038/nature07107 · Cited by 2,536
ChIP-seq accurately predicts tissue-specific activity of enhancers
Visel, A., Blow, M. J., Li, Z., Zhang, T., Akiyama, J. A., Holt, A., Plajzer-Frick, I., Shoukry, M., Wright, C., Chen, F., et al. (2009) · Nature · doi:10.1038/nature07730 · Cited by 1,639 · cited 2×
“p300 has a strong correlation with enhancers [21,30,46].”
BackgroundLarge-scale analysis of the human and mouse transcriptomes
Su, A. I., Cooke, M. P., Ching, K. A., Hakak, Y., Walker, J. R., Wiltshire, T., Orth, A. P., Vega, R. G., Sapinoso, L. M., Moqrich, A., et al. (2002) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.012025199 · Cited by 1,466 · cited 1×
“Tissue specific gene lists were derived from the GNF SymAtlas database [52] and were based on the level of mRNA in T cells or pancreas compared to the median in all surveyed tissues with cutoffs (20-fold higher for T cells, 5fold higher for pancreas) that returned similar sized lists.”
MethodHigh-Resolution Mapping and Characterization of Open Chromatin across the Genome
Boyle, A. P., Davis, S., Shulha, H. P., Meltzer, P., Margulies, E. H., Weng, Z., Furey, T. S., & Crawford, G. E. (2008) · Cell · doi:10.1016/j.cell.2007.12.014 · Cited by 1,415 · cited 1×
“Jurkat cell line) identifies DNase I accessible regions as mapped by high-throughput sequencing and ChIP-chip”
BackgroundGenome-wide mapping of HATs and HDACs reveals distinct functions in active and inactive genes
Wang, Z., Zang, C., Cui, K., Schones, D. E., Barski, A., Peng, W., & Zhao, K. (2009) · Cell · doi:10.1016/j.cell.2009.06.049 · Cited by 1,344 · cited 1×
“p300 has a strong correlation with enhancers [21,30,46].”
BackgroundHertz, G. Z., & Stormo, G. D. (1999) · Bioinformatics · doi:10.1093/bioinformatics/15.7.563 · Cited by 1,243 · cited 4×
“PATSER score cutoffs used were Motif 1:9; Motif 2:12; Motif 4:10.3.”
BackgroundInfluentialGoMiner: a resource for biological interpretation of genomic and proteomic data
Zeeberg, B. R., Feng, W., Wang, G., Wang, M. D., Fojo, A. T., Sunshine, M., Narasimhan, S., Kane, D. W., Reinhold, W. C., Lababidi, S., et al. (2003) · Genome Biology · doi:10.1186/gb-2003-4-4-r28 · Cited by 1,198 · cited 1×
“Associated genes, as determined by nearest TSS, were searched for over-represented ontologies with the GoMiner program [29].”
MethodThe ETS-domain transcription factor family
Sharrocks, A. D. (2001) · Nature Reviews Molecular Cell Biology · doi:10.1038/35099076 · Cited by 1,086
Nucleosome positioning and gene regulation: advances through genomics
Jiang, C., & Pugh, B. F. (2009) · Nature Reviews Genetics · doi:10.1038/nrg2522 · Cited by 1,057 · cited 1×
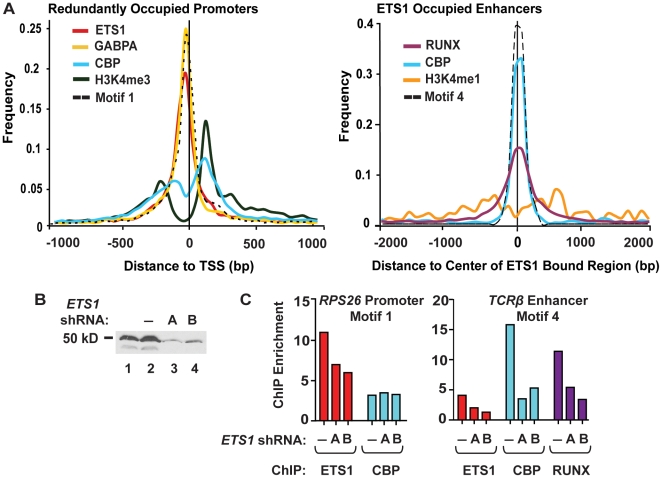
“This extremely TSS proximal location and the location of histone H3K4 tri-methylation on either side of the ETS1 bound region indicated that redundant ETS binding occurs in the nucleosome-free region [31].”
BackgroundTelomerase maintains telomere structure in normal human cells
Kenichi, M., Yu, E. Y., Shilagardi, K., Ben‐Porath, I., Currier, J. L., Metz, G. B., Brooks, M. W., Kaneko, S., Seishi, M., DeCaprio, J. A., et al. (2006) · Kanazawa University Repository for Academic Resources (DSpace) (Kanazawa University) · Cited by 738
Genome-wide analysis of transcription factor binding sites based on ChIP-Seq data
Valouev, A., Johnson, D. S., Sundquist, A., Medina, C., Anton, E., Batzoglou, S., Myers, R. M., & Sidow, A. (2008) · Nature Methods · doi:10.1038/nmeth.1246 · Cited by 695 · cited 2×
“Jurkat cells [23] with the same methodology as our ETS1 analysis.”
BackgroundMethodMolecular biology of the Ets family of transcription factors
Oikawa, T., & Yamada, T. (2003) · Gene · doi:10.1016/s0378-1119(02)01156-3 · Cited by 688
DNA binding site sequence directs glucocorticoid receptor structure and activity
Meijsing, S. H., Pufall, M. A., So, A. Y., Bates, D. L., Chen, L., & Yamamoto, K. R. (2009) · Science · doi:10.1126/science.1164265 · Cited by 673 · cited 1×
“binding site variants can alter the repressing or activating transcriptional activity of the factor once it is bound [6,7].”
BackgroundGiese, K., Kingsley, C., Kirshner, J. R., & Grosschedl, R. (1995) · Genes & Development · doi:10.1101/gad.9.8.995 · Cited by 541 · cited 1×
“) to regions of the human chromosome (Chr) indicated by chromosomal coordinates (NCBI Build 36.1). Positions of Refseq genes are shown with genes transcribed from left to right above the nucleotide position bar and genes in the opposite orientation below. Vertical lines (right) indicate the ETS/RUNX binding sequences…”
BackgroundInfluentialOne Nucleotide in a κB Site Can Determine Cofactor Specificity for NF-κB Dimers
Leung, T. H., Hoffmann, A., & Baltimore, D. (2004) · Cell · doi:10.1016/j.cell.2004.08.007 · Cited by 392
Regulation of Organogenesis by the Caenorhabditis elegans FoxA Protein PHA-4
Gaudet, J., & Mango, S. E. (2002) · Science · doi:10.1126/science.1065175 · Cited by 363
The Ets-1 Transcription Factor Is Required for the Development of Natural Killer Cells in Mice
Barton, K., Muthusamy, N., Fischer, C., Ting, C.-N., Walunas, T. L., Lanier, L. L., & Leiden, J. M. (1998) · Immunity · doi:10.1016/s1074-7613(00)80638-x · Cited by 359 · cited 2×
“ETS1 and RUNX co-occupancy predict tissue-specific enhancers Mice with an ETS1 gene disruption have reduced numbers of NK and NKT cells and show defects in T cell activation [14,38,39].”
BackgroundResultCombinatorial Regulation of Endothelial Gene Expression by Ets and Forkhead Transcription Factors
De Val, S., Chi, N. C., Meadows, S. M., Minovitsky, S., Anderson, J. P., Harris, I. S., Ehlers, M. L., Agarwal, P., Visel, A., Xu, S.-M., et al. (2008) · Cell · doi:10.1016/j.cell.2008.10.049 · Cited by 343 · cited 1×
“and sequence preferences, experimental data indicate that individual ETS proteins have unique biological functions [10–13].”
BackgroundDefective activation and survival of T cells lacking the Ets-1 transcription factor
Muthusamy, N., Barton, K., & Leiden, J. M. (1995) · Nature · doi:10.1038/377639a0 · Cited by 330 · cited 2×
“ETS1 and RUNX co-occupancy predict tissue-specific enhancers Mice with an ETS1 gene disruption have reduced numbers of NK and NKT cells and show defects in T cell activation [14,38,39].”
BackgroundERM is required for transcriptional control of the spermatogonial stem cell niche
Chen, C., Ouyang, W., Grigura, V., Zhou, Q., Carnes, K., Lim, H., Zhao, G.-Q., Arber, S., Kurpios, N., Murphy, T. L., et al. (2005) · Nature · doi:10.1038/nature03894 · Cited by 321
Bories, J.-C., Willerford, D. M., Grévin, D., Davidson, L., Camus, A., Martin, P., Stéhelin, D., & Alt, F. W. (1995) · Nature · doi:10.1038/377635a0 · Cited by 317 · cited 1×
“ETS1 and RUNX co-occupancy predict tissue-specific enhancers Mice with an ETS1 gene disruption have reduced numbers of NK and NKT cells and show defects in T cell activation [14,38,39].”
BackgroundKitabayashi, I. (1998) · The EMBO Journal · doi:10.1093/emboj/17.11.2994 · Cited by 306 · cited 1×
“For example, because both ETS1 and RUNX can bind the coactivator CBP [15,16,45], and CBP occupies the same position as ETS1 and RUNX at enhancers (Figure 6A), cooperative CBP recruitment may require this particular configuration of ETS1 and RUNX.”
BackgroundHollenhorst, P. C., Shah, A. A., Hopkins, C., & Graves, B. J. (2007) · Genes & Development · doi:10.1101/gad.1561707 · Cited by 290 · cited 9×
“promoters, the sequence CCGGAAGT and CpG islands [18].”
BackgroundMethodInfluentialSelf-citationEgawa, T., Eberl, G., Taniuchi, I., Benlagha, K., Geissmann, F., Hennighausen, L., Bendelac, A., & Littman, D. R. (2005) · Immunity · doi:10.1016/j.immuni.2005.03.011 · Cited by 270
Chromatin decouples promoter threshold from dynamic range
Lam, F. H., Steger, D. J., & O’Shea, E. K. (2008) · Nature · doi:10.1038/nature06867 · Cited by 244 · cited 1×
“In yeast, PHO4 responsiveness to phosphate levels is regulated by alterative sequence motifs that affect affinity and program different roles for binding sites [5].”
BackgroundEmpirical methods for controlling false positives and estimating confidence in ChIP-Seq peaks
Nix, D. A., Courdy, S. J., & Boucher, K. M. (2008) · BMC Bioinformatics · doi:10.1186/1471-2105-9-523 · Cited by 225 · cited 1×
“The following software from the Useq package [50] was used to identify regions enriched by ChIP compared to input control.”
MethodCooperative binding of Ets-1 and core binding factor to DNA.
Wotton, D., Ghysdael, J., Wang, S., Speck, N. A., & Owen, M. J. (1994) · Molecular and Cellular Biology · doi:10.1128/mcb.14.1.840 · Cited by 216 · cited 1×
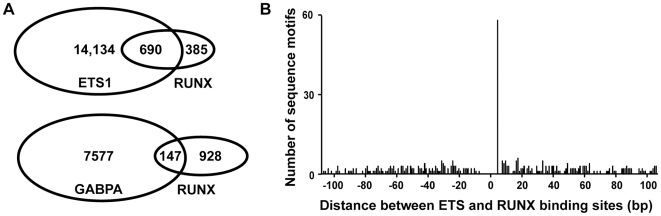
“This strict conservation was somewhat surprising because ETS1 and RUNX1 bind to DNA cooperatively in vitro at a variety of other spacings and orientations [26,43].”
BackgroundSelf-citationHollenhorst, P. C. (2004) · Nucleic Acids Research · doi:10.1093/nar/gkh906 · Cited by 214 · cited 1×
“ETS family members are extensively coexpressed [8,9].”
Self-citationYang, C., Shapiro, L. H., Rivera, M., Kumar, A., & Brindle, P. K. (1998) · Molecular and Cellular Biology · doi:10.1128/mcb.18.4.2218 · Cited by 213 · cited 1×
“For example, because both ETS1 and RUNX can bind the coactivator CBP [15,16,45], and CBP occupies the same position as ETS1 and RUNX at enhancers (Figure 6A), cooperative CBP recruitment may require this particular configuration of ETS1 and RUNX.”
BackgroundRas/Mitogen-Activated Protein Kinase Signaling Activates Ets-1 and Ets-2 by CBP/p300 Recruitment
Foulds, C. E., Nelson, M. L., Blaszczak, A. G., & Graves, B. J. (2004) · Molecular and Cellular Biology · doi:10.1128/mcb.24.24.10954-10964.2004 · Cited by 190
Self-citationRobertson, A. G., Bilenky, M., Tam, A., Zhao, Y., Zeng, T., Thiessen, N., Cezard, T., Fejes, A. P., Wederell, E. D., Cullum, R., et al. (2008) · Genome Research · doi:10.1101/gr.078519.108 · Cited by 182 · cited 1×
“mono-methylation is enriched in enhancers [21,22].”
A Mechanism for Coordinating Chromatin Modification and Preinitiation Complex Assembly
Black, J. C., Choi, J. E., Lombardo, S. R., & Carey, M. (2006) · Molecular Cell · doi:10.1016/j.molcel.2006.07.018 · Cited by 169 · cited 1×
“Potential CBP recruitment mechanisms include interaction with general transcription factors [47] and enhancer-promoter looping [48,49].”
BackgroundSun, W., Graves, B. J., & Speck, N. A. (1995) · Journal of Virology · doi:10.1128/jvi.69.8.4941-4949.1995 · Cited by 149 · cited 2×
“Vertical lines (right) indicate the ETS/RUNX binding sequences previously tested for function [27,44] in the TCRa enhancer (sequence GAGGATGTGGC) or the TCRb enhancer (sequence CAGGATGTGGT).”
BackgroundSelf-citationWang, C. Y., Bassuk, A. G., Boise, L. H., Thompson, C. B., Bravo, R., & Leiden, J. M. (1994) · Molecular and Cellular Biology · doi:10.1128/mcb.14.2.1153 · Cited by 143 · cited 1×
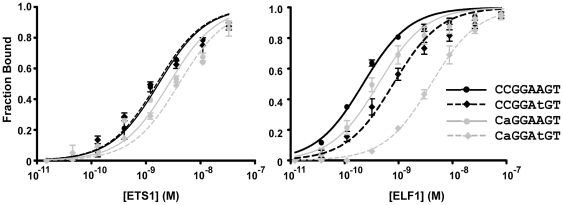
“To test the ability of the two nucleotide changes to act alone or in combination to select for ETS1 we measured the relative binding affinity of ETS1 and second ETS factor, ELF1 which is also reported to be active in T cells [25].”
BackgroundJayaraman, G., Srinivas, R., Duggan, C., Ferreira, E., Swaminathan, S., Somasundaram, K., Williams, J., Hauser, C., Kurkinen, M., Dhar, R., et al. (1999) · Journal of Biological Chemistry · doi:10.1074/jbc.274.24.17342 · Cited by 139
Galang, C. K., Muller, W. J., Foos, G., Oshima, R. G., & Hauser, C. A. (2004) · Journal of Biological Chemistry · doi:10.1074/jbc.m311887200 · Cited by 132 · cited 1×
“ETS family members are extensively coexpressed [8,9].”
E2F in vivo binding specificity: Comparison of consensus versus nonconsensus binding sites
Rabinovich, A., Jin, V. X., Rabinovich, R., Xu, X., & Farnham, P. J. (2008) · Genome Research · doi:10.1101/gr.080622.108 · Cited by 131 · cited 1×
“The emerging picture is that no single sequence motif fully explains all in vivo binding [1–3].”
BackgroundAuto-Inhibition of Ets-1 Is Counteracted by DNA Binding Cooperativity with Core-Binding Factor α2
Goetz, T. L., Gu, T.-L., Speck, N. A., & Graves, B. J. (2000) · Molecular and Cellular Biology · doi:10.1128/mcb.20.1.81-90.2000 · Cited by 128 · cited 1×
“Unique cooperative DNA binding between closely apposed binding proteins can also drive specific occupancy of transcription factors. A well-characterized partnership for ETS1 is with the RUNX factors”
BackgroundSelf-citationOhno, S., Sato, T., Kohu, K., Takeda, K., Okumura, K., Satake, M., & Habu, S. (2007) · International Immunology · doi:10.1093/intimm/dxm120 · Cited by 100 · cited 1×
“RUNX genes are essential for NK, NKT, and T cell differentiation [40–42].”
BackgroundGaston, K., & Fried, M. (1995) · Nucleic Acids Research · doi:10.1093/nar/23.6.901 · Cited by 99 · cited 1×
“the binding of ETS proteins [33,34].”
Yokomori, N., Kobayashi, R., Moore, R., Sueyoshi, T., & Negishi, M. (1995) · Molecular and Cellular Biology · doi:10.1128/mcb.15.10.5355 · Cited by 88 · cited 1×
“the binding of ETS proteins [33,34].”
Mechanism of Action of a Distal NF-κB-Dependent Enhancer
Teferedegne, B., Green, M. R., Guo, Z., & Boss, J. M. (2006) · Molecular and Cellular Biology · doi:10.1128/mcb.00271-06 · Cited by 85 · cited 1×
“Potential CBP recruitment mechanisms include interaction with general transcription factors [47] and enhancer-promoter looping [48,49].”
BackgroundChIPping away at gene regulation
Massie, C. E., & Mills, I. G. (2008) · EMBO reports · doi:10.1038/embor.2008.44 · Cited by 77 · cited 1×
“High-throughput sequencing coupled with chromatin immunoprecipitation (ChIP-seq) facilitates genome-wide searches for transcription factor binding sites [1].”
BackgroundGuo, Y., Maillard, I., Chakraborti, S., Rothenberg, E. V., & Speck, N. A. (2008) · Blood · doi:10.1182/blood-2007-10-120261 · Cited by 74 · cited 1×
“RUNX genes are essential for NK, NKT, and T cell differentiation [40–42].”
BackgroundSelf-citationTelomerase Maintains Telomere Structure in Normal Human Cells
Masutomi, K., Yu, E. Y., Khurts, S., Ben-Porath, I., Currier, J. L., Metz, G. B., Brooks, M. W., Kaneko, S., Murakami, S., DeCaprio, J. A., et al. (2003) · Cell · doi:10.1016/s0092-8674(03)00550-6 · Cited by 70 · cited 1×
“1p [51] and introduced to Jurkat T cells by MMLV based retroviruses.”
BackgroundJi, H., Vokes, S. A., & Wong, W. H. (2006) · Nucleic Acids Research · doi:10.1093/nar/gkl803 · Cited by 69 · cited 1×
“The emerging picture is that no single sequence motif fully explains all in vivo binding [1–3].”
BackgroundRozenberg, J. M., Shlyakhtenko, A., Glass, K., Rishi, V., Myakishev, M. V., FitzGerald, P. C., & Vinson, C. (2008) · BMC Genomics · doi:10.1186/1471-2164-9-67 · Cited by 62
Bosselut, R., Levin, J., Adjadj, E., & Ghysdael, J. (1993) · Nucleic Acids Research · doi:10.1093/nar/21.22.5184 · Cited by 56
Resendes, K. K., & Rosmarin, A. G. (2006) · Molecular and Cellular Biology · doi:10.1128/mcb.26.8.3060-3070.2006 · Cited by 29 · cited 1×
“Potential CBP recruitment mechanisms include interaction with general transcription factors [47] and enhancer-promoter looping [48,49].”
Background
Cited by
Annotation of functional variation in personal genomes using RegulomeDB
Boyle, A. P., Hong, E. L., Hariharan, M., Cheng, Y., Schaub, M. A., Kasowski, M., Karczewski, K. J., Park, J., Hitz, B. C., Weng, S., et al. (2012) · Genome Research · doi:10.1101/gr.137323.112 · Cited by 2,722
“Inaddition, we have included transcriptionfactor ChIP-seq data availablefrom the NCBI Sequence Read Archive (Hollenhorst et al. 2009; Jolma et al. 2010; Verzi et al. 2010; Wei et al. 2010; Hu et al. 2011; Lo et al. 2011; Novershtern et al. 2011; Palii et al. 2011; Yu et al. 2011).”
MethodGenome-wide analysis of ETS-family DNA-binding in vitro and in vivo
Wei, G., Badis, G., Berger, M. F., Kivioja, T., Palin, K., Enge, M., Bonke, M., Jolma, A., Varjosalo, M., Gehrke, A. R., et al. (2010) · The EMBO Journal · doi:10.1038/emboj.2010.106 · Cited by 568
“ELK1 or ELK4 can bind DNA together with SRF (Dalton and Treisman, 1992; Cooper et al, 2007; Boros et al, 2009), FLI1 associates with SMAD3 (Ravasi et al, 2010) and ETS1 can bind to composite sites with PAX5 (Garvie et al, 2001) and RUNX1 (Hollenhorst et al, 2007, 2009).”
InfluentialGenomic and biochemical insights into the specificity of ETS transcription factors
Hollenhorst, P. C., McIntosh, L. P., & Graves, B. J. (2011) · Annual Review of Biochemistry · doi:10.1146/annurev.biochem.79.081507.103945 · Cited by 490
Self-citationGordân, R., Shen, N., Dror, I., Zhou, T., Horton, J., Rohs, R., & Bulyk, M. L. (2013) · Cell Reports · doi:10.1016/j.celrep.2013.03.014 · Cited by 355
Sanda, T., Lawton, L. N., Barrasa, M. I., Fan, Z. P., Kohlhammer, H., Gutierrez, A., Ma, W., Tatarek, J., Ahn, Y., Kelliher, M. A., et al. (2012) · Cancer Cell · doi:10.1016/j.ccr.2012.06.007 · Cited by 334
“By comparing the ChIP-seq binding profiles for TAL1 complex members determined in our study with those described by three other groups (Hollenhorst et al., 2009; Palii et al., 2011b; Valouev et al., 2008), we determined that ETS1 occupancy correlates with the binding of other members of the TAL1 complex, as compared w…”
Metadata
- Authors
- Hollenhorst, P. C., Chandler, K. J., Poulsen, R. L., Johnson, W. E., Speck, N. A., & Graves, B. J.
- Affiliations
- University of Utah (US)
- Brigham Young University (US)
- Abramson Cancer Center (US)
- Corresponding author
- Graves, Barbara J.
- Venue
- PLoS Genetics
- Publisher
- Public Library of Science (PLoS)
- Published
- 2009-12-18
- Volume
- 5
- Issue
- 12
- Pages
- e1000778
- ISSN
- 1553-7390 (ISSN-L)
- 1553-7404
- PMC
- PMC2787013
- OpenAlex
- W2127600515
- Cited by
- 198
- References
- 53
- Citations by year
- 2026: 4 · 2025: 4 · 2024: 8 · 2023: 7 · 2022: 3 · 2021: 13 · 2020: 7 · 2019: 11 · 2018: 8 · 2017: 9 · 2016: 13 · 2015: 16 · 2014: 18 · 2013: 16 · 2012: 23
- FWCI
- 8.18
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Locations
- PLoS Genetics (publishedVersion, cc-by)
- Europe PMC (PubMed Central) (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- DOAJ (DOAJ: Directory of Open Access Journals) (submittedVersion, cc-by-sa)
- Figshare (submittedVersion, cc-by)
- Funders
- Huntsman Cancer Institute
- National Institutes of Health (CA42014)
- National Heart, Lung, and Blood Institute (HL089969, R01HL089969)
- National Cancer Institute (R01CA058343, CA42014, P30CA042014)
- National Institute of General Medical Sciences (GM 38663, R01GM038663)
- Topics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Genomics and Chromatin Dynamics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Chromatin Remodeling and Cancer
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Gene Regulatory Network Analysis
- Keywords
- ETS1, ETS transcription factors, DNA sequence specificity, transcription factor binding motifs, enhancer binding, promoter binding, T cell activation, GABPA, RUNX, DNase I sensitivity, housekeeping genes, chromatin occupancy
- MeSH terms
- Base Sequence, Binding Sites, Enhancer Elements, Genetic, Humans, Lymphocyte Activation, Promoter Regions, Genetic, Protein Binding, T-Lymphocytes, Transcription Factors, Genome, Human, Jurkat Cells, Core Binding Factor alpha Subunits, Proto-Oncogene Protein c-ets-1, GA-Binding Protein Transcription Factor, Gene Regulatory Networks
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
Data sources
Bibliographic data: Semantic Scholar, OpenAlex, Crossref.
Contains information from the Semantic Scholar Academic Graph Datasets, made available under the ODC Attribution License (ODC-BY 1.0).
Semantic Scholar’s data is described in: Kinney, R., et al. (2023). The Semantic Scholar Open Data Platform. arXiv:2301.10140.
