

The DOI matches its Crossref record; 78 of the 78 references it cites were found in a registry or an index; 21 of the 184 sources its claims cite were checked for support.
Recent evidence that TADs and chromatin loops are dynamic structures
Open accessAbstract
Mammalian genomes are folded into spatial domains, which regulate gene expression by modulating enhancer-promoter contacts. Here, we review recent studies on the structure and function of Topologically Associating Domains (TADs) and chromatin loops. We discuss how loop extrusion models can explain TAD formation and evidence that TADs are formed by the ring-shaped protein complex, cohesin, and that TAD boundaries are established by the DNA-binding protein, CTCF. We discuss our recent genomic, biochemical and single-molecule imaging studies on CTCF and cohesin, which suggest that TADs and chromatin loops are dynamic structures. We highlight complementary polymer simulation studies and Hi-C studies employing acute depletion of CTCF and cohesin, which also support such a dynamic model. We discuss the limitations of each approach and conclude that in aggregate the available evidence argues against stable loops and supports a model where TADs are dynamic structures that continually form and break throughout the cell cycle.
Overview
AI snapshot
Written from the paper’s full text.
TL;DR
This review argues that CTCF/cohesin-dependent TADs and chromatin loops are dynamic structures that continually form and break, with mean lifetimes of minutes to tens of minutes, rather than stable structures. It integrates single-molecule imaging, polymer simulations, and acute CTCF/cohesin depletion Hi-C studies to support a loop-extrusion/dynamic LMC model.
Key findings
- TADs are formed by cohesin-mediated loop extrusion and boundaries are established by CTCF; acute depletion of CTCF or cohesin causes TADs and loops to largely disappear, with CTCF loss having essentially no effect on genome-averaged contact probability and cohesin loss reducing contact probability at the tens-to-hundreds-of-kilobases scale. Cohesin loss increases epigenomic compartmentalization ∼2-fold.
- Imaging in mES and U2OS cells yields CTCF chromatin residence times of ∼1–4 min and cohesin G1 residence times of ∼20–25 min; because cohesin eventually dissociates, the paper proposes that cohesin-mediated loops have mean lifetimes of a few to tens of minutes.
- In ΔWAPL cells, average TAD size increases substantially and median loop size increases from 370 kb to 575 kb, supporting dynamic cohesin-controlled TADs. CTCF binds ∼2-fold more sites than cohesin (68,077 vs. 33,434 called peaks).
- TADs emerge at the population level from many differently positioned extrusion complexes; even strong Hi-C loop anchors contact in only a small subset of cells, and insulation between adjacent TADs is only ∼2-fold.
Methods
- Design: Extra View/review synthesizing recent studies on TAD and chromatin-loop structure and function, including the authors’ genomic, biochemical, and single-molecule imaging work plus complementary polymer simulation and Hi-C acute depletion studies.
- Data/sample: live-cell imaging used CRISPR/Cas9-mediated homozygous HaloTag or SNAPf tagging of CTCF and cohesin in mouse embryonic stem cells and human U2OS cells, with ChIP-Seq, co-immunoprecipitation, single-molecule tracking at 225 Hz, FRAP, and PALM/STORM; cited Hi-C studies include ΔWAPL cells and auxin-AID-mediated acute Rad21 degradation.
- Analysis: critical synthesis and evaluation of evidence across imaging, polymer modeling, and Hi-C perturbation approaches; the article is a review/synthesis rather than a new primary experimental study.
Limitations
- Stated: imaging cannot identify which locus a molecule is bound to, reports genomic-average residence times, binding times are stochastic and exponentially distributed, very small (<5%) subpopulations with different binding times cannot be excluded, and using CTCF/cohesin binding dynamics to infer loop stability is indirect.
- Stated: polymer modeling faces the problem that many mutually inconsistent models can fit the data, and fitting data does not prove mechanistic assumptions; acute cohesin degradation studies may not reflect normal turnover rates and have poor time resolution.
- Stated/evident: final demonstration that TADs and loops are dynamic requires direct real-time observation of specific loci in live cells, and whether epigenomic compartments are stable or dynamic remains unknown; the review’s conclusion is an aggregate argument from indirect approaches.
Model-written summary. Check it against the paper before relying on it.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
62 Not checked yet · 34 Own interpretation · 17 Own result · 11 Own method · 5 Partly supported · 3 Supported so far · 3 No basis given · 2 Supported · 1 Couldn’t confirm · accuracy not yet measured
The cited sources support only part of this claim — read each source’s verdict below.
In the paper
“A large body of evidence suggests that TADs correspond to functional regulatory domains by primarily restricting contact between enhancers and promoters to occur within the same TAD3,21–25”
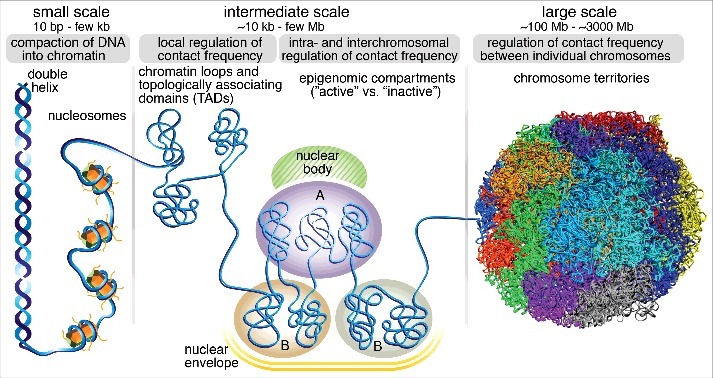
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Partly supportedcites [3] sourceExperimental — accuracy not yet measured
The conclusion (page unavailable) says TADs define regulatory neighborhoods, and the boundary-deletion passage reports ectopic contacts between neighboring TADs. The paper supports a role for TADs in spatially limiting regulatory contacts, but it does not specifically establish that enhancer–promoter contacts occur primarily within the same TAD. (LLM, conf=0.84)
- Not checked yetcites [21] source
- Not checked yetcites [22] source
- Supportedcites [23] source
In Results, under “Long-range interactions and 3D architectural features” (page unavailable), the paper reports that most promoter–genome interactions occur within TADs; only 6% in ESCs and 9.1% in FLCs cross TAD boundaries. This supports the citing sentence’s hedged claim that TADs primarily restrict regulatory contacts to within the same domain, while allowing exceptions. (LLM, conf=0.88)
- Supportedcites [24] source
The paper reports that regulatory domains lie largely within TADs and that enhancer influence appears confined to the topological domain (Abstract; Discussion; page numbers unavailable). It also notes that TAD transitions may dampen rather than absolutely block regulatory influence, consistent with the claim’s qualifier “primarily.” (LLM, conf=0.88)
- Partly supportedcites [25] sourceExperimental — accuracy not yet measured
The Discussion (page unavailable) says CCDs align with TADs and that loops within them have transcriptional and regulatory functions. Results IV gives an example of an enhancer interacting with a promoter through such a loop. The copy does not establish that TAD boundaries primarily restrict enhancer–promoter contacts to the same TAD. (LLM, conf=0.82)
hedgedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- Partly supported
The cited sources support only part of this claim — read each source’s verdict below.
In the paper
“A key piece of the puzzle came from the “convergent rule”: loop-anchored TADs almost always form between CTCF binding sites in a convergent orientation.16,20”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
- Supportedcites [16] source
The Discussion (page unavailable) calls domains demarcated by loops “loop domains” and reports that CTCF motifs at loop anchors are convergent in more than 90% of cases. The Results (page unavailable) likewise find convergent motifs at 92% of the examined loop peaks, supporting the stated convergent rule. (LLM, conf=0.88)
- Partly supportedcites [20] sourceExperimental — accuracy not yet measured
The Results section, “Conserved CTCF Sites Are Directional and Interact with Other Conserved Sites” (page unavailable), reports domain-defining interactions anchored by pairs of conserved CTCF sites on opposite strands. It does not establish that the sites face one another in a convergent orientation or that this holds for almost all loop-anchored TADs. (LLM, conf=0.86)
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- Supported
The sources with a verdict support this claim; the rest weren’t checked yet, have no full text we could read, or their verdicts aren’t rated yet.
In the paper
“Thus, the ΔWAPL Hi-C studies12,14,15 support our conclusion that CTCF binds more dynamically than cohesin.7”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Supportedcites [12] source
The Results sections report that WAPL loss impairs cohesin turnover and that ΔWAPL Hi-C reveals loops extending beyond CTCF boundaries. In the Discussion (‘To the Boundary and Beyond’), the authors propose that longer cohesin residence could let cohesin remain on DNA after CTCF dissociates. The study therefore supports the citing authors’ inference, though it does not directly measure a CTCF-versus-cohesin binding-rate difference. (LLM, conf=0.84)
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
- Not checked yetcites [15] Gassler J, 2017, bioRxiv
- Supportedcites [7] source
The Results section, “CTCF and cohesin bind chromatin with very different dynamics,” reports a ~10–20-fold difference in residence times. The paper also states that CTCF binds and unbinds its sites ~20–30 times per cohesin binding cycle. Citation 7 supports the conclusion about binding dynamics; the ΔWAPL Hi-C studies have separate citations. (LLM, conf=0.93)
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- Supported
The sources with a verdict support this claim; the rest weren’t checked yet, have no full text we could read, or their verdicts aren’t rated yet.
In the paper
“cohesin's residence time is prolonged in ΔWAPL cells,12,14”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Supportedcites [12] source
The Results section (‘WAPL Restricts Chromatin Loop Extension’) reports that WAPL deficiency severely impaired cohesin turnover on chromatin in ΔWAPL HAP1 cells. The Discussion (‘To the Boundary and Beyond’) explicitly describes a longer residence time of cohesin on DNA in WAPL-deficient cells. (LLM, conf=0.93)
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- Supported
Every source the paper cites for this claim was checked and supports it.
In the paper
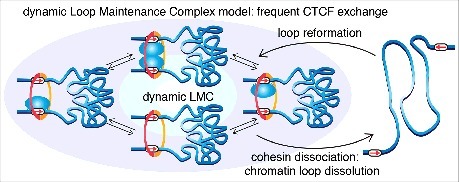
“we propose that cohesin-mediated chromatin loops are dynamic structures that continuously form and fall apart throughout the cell cycle”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
What the sources say
- Supportedcites [7] source
The Discussion says cohesin holds chromatin loops together and that cohesin dissociation likely causes them to fall apart. It concludes that loops are continuously formed and dissolved throughout a typical mammalian cell cycle, matching the citing sentence’s proposal. (LLM, conf=0.94)
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- The authors state this as an assumption: CTCF positions cohesin at its convergent cognate binding sites and cohesin holds together two strands of chromatin.
- Supported
In the paper
“We next performed co-immunoprecipitation (IP) experiments and found that CTCF IP pulled down all the subunits of the cohesin complex consistent with earlier reports,61”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
What the sources say
- Not checked yetcites [61] source
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“in mES cells, ∼50% of all CTCF molecules are bound to cognate sites.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“our co-IP, ChIP-Seq and STORM studies strongly suggested that CTCF and cohesin form an LMC protein complex”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
boostedstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We found that CTCF and cohesin also exhibit very distinct diffusion dynamics”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“the search mechanism involves large amounts of non-specific chromatin interactions (such as sliding or hopping; ∼35%) in addition to 3D diffusion (∼65%).”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- It may state two separate claims as one. 50
- Probably not a substantial claim. 13
Every source the paper cites for this claim was checked and supports it.
In the paper
“In mammalian nuclei, active chromatin tends to associate with active chromatin and vice versa giving rise to a “plaid” pattern in maps obtained by genome-wide chromosome conformation capture studies (Hi-C).5”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Supportedcites [5] source
The passage on the plaid pattern (labeled Abstract in our copy) says contacts are enriched within each of two compartments and depleted between them. Another passage under the same label identifies these as open and closed chromatin compartments and notes interactions between active genes and between inactive genes. No page numbers are provided in our copy. (LLM, conf=0.93)
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- Supported
The cited sources that could be checked couldn’t confirm or dispute this claim.
In the paper
“These epigenomic compartments range in size from 6 kb to more than 5 Mb.16”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Could not verifycites [16] sourceExperimental — accuracy not yet measured
The Results section on nuclear subcompartments reports a median interval length of 300 Kb but gives no range from 6 kb to more than 5 Mb. The Results section on small domains gives a 40 Kb–3 Mb range, but those domains are not identified as the epigenomic compartments in the claim. Searches for the claimed range and for epigenomic compartment sizes found no passage establishing it. (LLM, conf=0.70)
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
- Could not verify
The cited sources support only part of this claim — read each source’s verdict below.
In the paper
“Both DNA FISH3,9,36–39 and single-cell Hi-C40,41 studies show that genome organization is highly variable between cells and that even strong Hi-C loop anchors only contact in a small subset of cells”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
- Could not verifycites [3] sourceExperimental — accuracy not yet measured
The paper’s Abstract reports DNA FISH measurements of probe distances and colocalisation in the X-inactivation centre, but does not say that genome organisation is highly variable between individual cells. Searches for cell-to-cell variability and the fraction of cells with contacts found no passage addressing whether strong Hi-C loop anchors contact in only a small subset of cells; the paper describes 5C rather than single-cell Hi-C. (LLM, conf=0.73)
- Not checked yetcites [9] source
- Not checked yetcites [36] source
- Not checked yetcites [37] Finn E, 2017, bioRxiv
- Partly supportedcites [38] sourceExperimental — accuracy not yet measured
The Results section ('The internal structure of the Tsix TAD is highly variable between cells'; page unavailable) reports DNA FISH evidence of substantial cell-to-cell variation and estimates that its strongest long-range contacts occur in 34–45% of cells. But these are contacts identified from 5C at the Tsix TAD, not strong Hi-C loop anchors. The Introduction also says single-cell Hi-C lacked sufficient resolution to assess contact frequencies within individual TADs. (LLM, conf=0.88)
- Not checked yetcites [39] source
- Not checked yetcites [40] source
- Not checked yetcites [41] source
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- Could not verify
The sources with a verdict support this claim; the rest weren’t checked yet, have no full text we could read, or their verdicts aren’t rated yet.
In the paper
“Finally, ∼18% of TAD boundaries appear to be partially resistant to CTCF loss,10 suggesting that additional boundary factors, such as active promoters4 since engaged RNA Pol II can block cohesin extrusion46 as well as alternative architectural factors, may also play a role.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
- Supportedcites [10] source
The Results section, “CTCF Depletion Triggers Dramatic Loss of TAD Insulation,” reports that 1,000 boundaries—18% of the initial boundaries—persisted without detectable CTCF binding and were much less affected by depletion. This supports the ∼18% figure and the description of partial resistance; the citing sentence attaches this citation to that finding, not to the later examples of possible factors. (LLM, conf=0.94)
- Could not verifycites [4] sourceExperimental — accuracy not yet measured
The paper’s discussion of boundary factors (section labeled Abstract; page unavailable) reports CTCF enrichment and notes that CTCF binding alone is insufficient to demarcate boundaries. Searches for the cited claim’s distinctive terms found no passage reporting CTCF loss or that approximately 18% of boundaries resist it. The active-promoter suggestion is attached to a different citation in the citing sentence. (LLM, conf=0.75)
- Not checked yetcites [46] source
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- Supported
The cited sources support only part of this claim — read each source’s verdict below.
In the paper
“Thus, chromatin is still compacted and extruded by cohesin, but without sharp boundaries, TADs disappear in Hi-C maps.10,14”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
- Partly supportedcites [10] sourceExperimental — accuracy not yet measured
The Results section (“CTCF Depletion Triggers Dramatic Loss of TAD Insulation”; page unavailable) reports that Hi-C maps showed extensive contacts across former TAD boundaries after CTCF depletion, but 18% of boundaries persisted. The Discussion says cohesin packages chromatin and the observations are consistent with loop extrusion; it does not establish ongoing extrusion as a measured fact. Thus the claim captures the main pattern but overstates both the mechanism and the disappearance of TADs. (LLM, conf=0.88)
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- Partly supported
The cited sources support only part of this claim — read each source’s verdict below.
In the paper
“Notably, a key advantage of dynamic loop extrusion models is that they can explain recent perturbation experiments where CTCF binding sites have been added or deleted9,49-51 and also explain the loss of either CTCF or cohesin.10-15”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
- Not checked yetcites [9] source
- Supportedcites [49] source
The citation is attached to the perturbation experiments, not to the citing authors’ claim about what loop-extrusion models can explain. The paper describes a 9-bp deletion of a CTCF-binding motif in the HoxA cluster and reports that the resulting loss of binding relocates a chromatin boundary during motor-neuron differentiation (passages [8] and [7]). It therefore provides an example of the cited binding-site deletion experiments; it need not also test site addition or the model. (LLM, conf=0.91)
- Supportedcites [50] source
The Results section on the β-globin locus reports CRISPR deletion of CTCF-binding sites and the resulting changes in chromatin looping, making this paper an example of the cited perturbation experiments. The citation is attached to those experiments, not to the sentence’s separate claims about loop-extrusion models or loss of CTCF or cohesin. Page numbers were not available in our copy. (LLM, conf=0.88)
- Not checked yetcites [51] source
- Supportedcites [10] source
The Discussion (page not supplied) says the CTCF-depletion results are compatible with models in which loops accumulate between CTCF-bound boundaries. It also describes a model in which cohesin packages chromatin while CTCF constrains that activity, accounting for their different depletion effects. This supports the part of the citing sentence about models explaining loss of CTCF or cohesin. (LLM, conf=0.87)
- Not checked yetcites [11] source
- Partly supportedcites [12] sourceExperimental — accuracy not yet measured
The Introduction (page unavailable) describes a loop-extrusion model in which cohesin enlarges loops and CTCF limits their extension. The Results sections on SCC4-independent cohesin loading and loop extension report that reducing chromatin-bound cohesin is associated with more diffuse TAD boundaries. The paper does not test the complete loss of either CTCF or cohesin; the added-or-deleted CTCF-site experiments are attached to a different citation group in the citing sentence. (LLM, conf=0.82)
- Not checked yetcites [13] Rao S, 2017, bioRxiv
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
- Not checked yetcites [15] Gassler J, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We additionally performed ChIP-Seq and found that although CTCF binds ∼2-fold more sites than cohesin (68,077 vs. 33,434 called peaks; note that cohesin extrusion likely “spreads out” its ChIP signal and thus results in fewer “peaks”), essentially all cohesin ChIP-Seq peaks co-localize with CTCF peaks.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Kinetic modeling of the FRAP data using a “reaction dominant” model yielded a FRAP residence time of ∼3-4 min in mES cells and somewhat longer in U2OS cells.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“FRAP and kinetic modeling revealed a G1 residence time of ∼20-25 min, ∼10-fold more stable than CTCF”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“we found an average CTCF SMT residence time of ∼1 min in mES cells for specific binding events at cognate sites and somewhat longer in U2OS cells.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We found that both CTCF and cohesin form small clusters”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“we showed that both CTCF and cohesin form small protein clusters7”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Conclusion and outlook
What the sources say
- Not checked yetcites [7] source
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“although we can report average residence times for CTCF (∼1–4 min) and cohesin (∼20-25 min in G1) in mESCs, these numbers are genomic averages.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
- Not checked yetcites [7] source
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“TADs may emerge at the population level when averaged over many heterogeneous single-cell genome topologies.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
None of the sources cited for this claim have been checked yet.
In the paper
“TADs were identified through Hi-C3,4 and their existence have since been confirmed by alternative methods such as intrinsic 3C (i3C),18 which avoids the cross-linking step and Genome Architecture Mapping (GAM),19 which avoids the ligation step.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Moreover, TADs often have a nested, hierarchical configuration, where smaller TADs can make up larger TADs, and range in size from ∼40 kb to ∼3 MB with a median size of ∼185 kb16, though these numbers depend somewhat on the resolution of the Hi-C data used to identify them”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Not checked yetcites [16] source
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“loss of a TAD boundary between limb enhancers and the wnt6 gene is sufficient to upregulate wnt6 expression and cause developmental defects in both mice and humans.28”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Not checked yetcites [28] source
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Accordingly, deletion of a boundary between two TADs causes ectopic contacts between previously insulated loci3 and can cause aberrant gene expression through improper enhancer-promoter contact.27,28”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“In contrast, compartments composed of repressed chromatin tend to be located near the nuclear envelope through lamina association and are also referred to as Lamina-Associated Domains (LADs)17”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
What the sources say
- Not checked yetcites [17] source
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
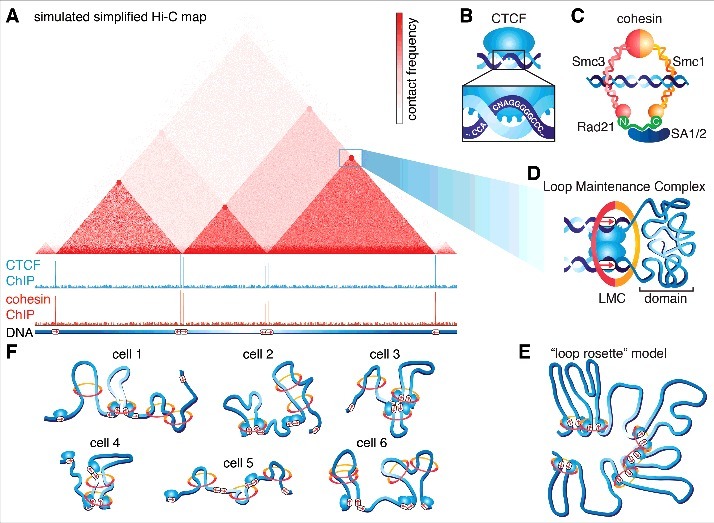
“TADs appear as triangles, within which there are more frequent chromatin contacts and are often marked by “cornerpeaks”, suggesting that they are held together by a chromatin loop.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- The authors state this as an assumption: The presence of CTCF and cohesin bound corner peaks in Hi-C maps corresponds to a chromatin loop held together by CTCF and cohesin.
The paper states this without a source or data behind it here, so there is nothing to check it against. The quote shows it is in the paper.
In the paper
“Below, simulated CTCF and cohesin ChIP-Seq tracks illustrating that TAD and loop boundaries are almost always bound by CTCF and cohesin.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs and epigenomic compartments: Interplay between structure and function
boostedstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Thus, TADs likely regulate enhancer-promoter contacts and gene expression.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Introduction
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“First, chromatin is organized into Topological Associating Domains (TADs) that are characterized by preferential contacts between loci inside the same TAD and insulation from loci in adjacent TADs.3,4”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Introduction
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Third, although it requires cohesin extrusion to be quite fast, closely related SMC-condensin complexes were recently found to extrude at ∼50 kb/min in B. subtilis52 and ∼16-19 kb/min in Caulobacter.53”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Although the loop extrusion model remains a hypothesis, it has proved remarkably resilient to testing.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- The authors state this as an assumption: In the loop extrusion model, cohesin spontaneously engages chromatin and begins extruding a DNA loop.
- The authors state this as an assumption: Loop extrusion continues until cohesin spontaneously falls off or until it encounters an occupied CTCF binding site in the convergent orientation.
None of the sources cited for this claim have been checked yet.
In the paper
“Cohesin is thought to topologically entrap DNA (Fig. 2C),34 a structural feature that enables cohesin to mediate multiple functions including sister chromatid cohesion and homologous recombination.35”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Since almost all TADs are demarcated by CTCF ChIP-Seq peaks,16 but only around one-third of CTCF ChIP-Seq peaks flank TADs,1,7”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Using slightly anthropomorphic imagery, CTCF is the “passive” partner and predominantly sits bound to its cognate sites and “waits” for extruding cohesin complexes, whereas cohesin plays the “active” role by constantly moving along and extruding DNA until it “finds” CTCF.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
- The authors state this as an assumption: In the loop extrusion model, cohesin spontaneously engages chromatin and begins extruding a DNA loop.
- The authors state this as an assumption: Loop extrusion continues until cohesin spontaneously falls off or until it encounters an occupied CTCF binding site in the convergent orientation.
None of the sources cited for this claim have been checked yet.
In the paper
“In accordance with the extrusion model, TADs and well-defined Hi-C loops largely disappear when either CTCF10,14 or cohesin11,13–15 is strongly depleted, but for different reasons.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Likewise, CTCF loss has only a small effect on epigenomic compartments,10 whereas cohesin loss increases the degree of epigenomic compartmentalization ∼2-fold.11,13”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Consistent with their different roles, CTCF loss has essentially no effect on genome-averaged contact probability at any distance scale,10 whereas cohesin loss significantly reduces contact probability at the scale of tens to hundreds of kilobases,11”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“First, we performed a series of control experiments to verify that tagging CTCF and cohesin – both essential proteins – did not affect their function or expression levels.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“The CTCF/cohesin anchored loop domain matching the Hi-C corner-peak actually only exists in a small subset of cells, which is also consistent with the high levels of cell-to-cell variability in contact probability observed in DNA FISH studies.3,9,36–39”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“What has been clear is that TADs and loops are absent in mitosis, but present in G1-phase.54,55”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Are TADs and chromatin loops dynamic or stable structures?
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“Since Hi-C provides a static snapshot derived from the average of a large cell population, Hi-C based methods are necessarily limited in their ability to reveal dynamics and heterogeneity.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Are TADs and chromatin loops dynamic or stable structures?
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“A unique advantage of live-cell imaging is that single protein molecules can be followed over time and their dynamics can thus be directly observed at the single-cell level.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds.
What the paper did — it cites no source for this, so there is none to check. The quote shows it is in the paper.
In the paper
“While single-cell methods such as single-cell Hi-C and DNA-FISH can report on cell-to-cell variability, they still provide a terminal snapshot and thus can only give limited dynamic information.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Are TADs and chromatin loops dynamic or stable structures?
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“In conclusion, recent studies10–15 employing induced CTCF and cohesin degradation now strongly support a model where cohesin forms TADs and CTCF establishes TAD boundaries.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
boostedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“In summary, CTCF and cohesin are required for chromatin looping,10–15 form a biochemically stable protein-complex and both bind chromatin at loop anchors.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
What the sources say
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“This result also argues against a hierarchical model where TADs are the building blocks of compartments and demonstrates that TADs and epigenomic compartments are formed by distinct and mutually antagonistic mechanisms.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
boostedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Cohesin loss has no apparent effect on CTCF binding to chromatin,13 consistent with CTCF functioning upstream of cohesin.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > TADs are formed by cohesin and TAD boundaries are defined by CTCF
What the sources say
- Not checked yetcites [13] Rao S, 2017, bioRxiv
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“after cohesin dissociation, previously held-together chromatin will likely only move apart slowly even though the loop is broken”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds.
In the paper
“these results are consistent with our imaging results showing that CTCF binding is stochastic and less stable than cohesin.7”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [7] source
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“The best agreement with experimental Hi-C data16 was obtained when cohesin extrudes for ∼120-240 kb before falling off and a mean separation of ∼120 kb between extrusion complexes (note that these are average numbers).8”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Upon auxin treatment, near-complete loss of Rad21 was achieved in 1 hour in Rao et al.13 or ∼20 min in Wutz et al..14”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [13] Rao S, 2017, bioRxiv
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“the loop extrusion model introduced by Fudenberg and Imakaev et al.8 explicitly favored dynamic loops and convincingly argued against static loops.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [8] source
boostedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“which is quite stable compared to conventional transcription factors (∼2-15 seconds),62 but very dynamic compared to the cell cycle (15-30 hours).”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Single-molecule imaging approaches suggest that TADs and loops are dynamic
What the sources say
- Not checked yetcites [62] source
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“which – assuming no change in cohesin's extrusion speed – would increase cohesin extrusion processivity.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
hedgedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper may give no reason why it holds.
- The authors state this as an assumption: In ΔWAPL cells, cohesin's extrusion speed does not change.
None of the sources cited for this claim have been checked yet.
In the paper
“the average TAD size increased substantially in ΔWAPL cells12,14,15 and the median loop size increased from 370 kb to 575 kb.12”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [12] source
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
- Not checked yetcites [15] Gassler J, 2017, bioRxiv
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“a recent study found that CTCF can form large foci upon senescence, which causes genome reorganization.74”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Conclusion and outlook
What the sources say
- Not checked yetcites [74] Zirkel A, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“Taken together, these studies13,14 suggest that the mechanisms by which TADs and loops are formed and broken down are both quite fast, which argues against stable TADs and favors dynamic TADs.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [13] Rao S, 2017, bioRxiv
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
hedgedstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We note that dynamically extruding cohesin complexes are also likely to be functionally important by facilitating dynamic and repeated enhancer-promoter scanning in cis.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Conclusion and outlook
hedgedstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
In the paper
“Similarly, Wutz et al. found that 96% of loops, but only 53% of TADs were lost 15 min after auxin addition, whereas TADs were fully lost at later time points.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
What the sources say
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“Nevertheless, it must be noted that the ability of a particular model to fit data does not prove that the model's mechanistic assumptions are also true.68”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
- Not checked yetcites [68] source
plain- Asserted: passes — The authors put it forward as true.
- Checkable: fails — It may be too vague to check against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. It may be too vague to check against evidence. The paper’s conclusions may not depend on it.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“These results show that loops and TADs rapidly disappear at a timescale of a few to tens of minutes after acute cohesin loss, which is consistent with the notion that cohesin binding dynamics control TAD dynamics.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Evidence that TADs and loops are dynamic from polymer simulation and acute CTCF/cohesin degradation studies
plainstates a possible cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
In the paper
“(∼18% of TAD boundaries were not sensitive to CTCF loss10 and could have different dynamics)”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
- Not checked yetcites [10] source
hedged- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“(genome organization dynamics could be different in some cell types, e.g. in post-mitotic olfactory sensory neurons, which exhibit a highly unusual and specialized nuclear organization69,70)”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Conclusion and outlook
hedgedstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: passes — The paper gives a reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it.
A conclusion the paper draws from its own results — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Almost certainly, some binding sites will exhibit longer and shorter binding times.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
boosted- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: fails — The paper’s conclusions may not depend on it.
- Based: fails — The paper may give no reason why it holds.
Probably not a substantial claim. The paper’s conclusions may not depend on it. The paper may give no reason why it holds.
- Rests on an assumption: Binding times to cognate sites are highly stochastic and exponentially distributed such that few events exhibit the mean value.
In the paper
“although TADs are somewhat conserved between different cell types,1 several do change.”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Conclusion and outlook
What the sources say
- Not checked yetcites [1] Merkenschlager M, 2017, Annu Rev Genomics Hum Genet
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“recent studies13,14 showing that TADs and loops are lost within tens of minutes after acute cohesin degradation and quickly reformed after cohesin replenishment”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
- Not checked yetcites [13] Rao S, 2017, bioRxiv
- Not checked yetcites [14] Wutz G, 2017, bioRxiv
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
None of the sources cited for this claim have been checked yet.
In the paper
“recent polymer studies8,9 of presumably cohesin-motor driven loop extrusion were able to quantitatively account for Hi-C data, but so was a mechanistically distinct model by Benedetti et al., where supercoiling drives the formation of TADs.66”
§ Recent evidence that TADs and chromatin loops are dynamic structures > Critical evaluation of evidence for TADs and loops being dynamic
What the sources say
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
It may state two separate claims as one.
The authors state this as an assumption.
The presence of CTCF and cohesin bound corner peaks in Hi-C maps corresponds to a chromatin loop held together by CTCF and cohesin.
“The presence of CTCF and cohesin bound “corner peaks” in Hi-C maps are generally assumed to correspond to a chromatin loop held together by CTCF and cohesin as sketched.”
The authors state this as an assumption.
TADs are formed by cohesin-mediated extrusion, which stops at occupied CTCF binding sites.
“This picture assumes that TADs are formed by cohesin-mediated extrusion, which stops at occupied CTCF binding sites.”
The authors state this as an assumption.
CTCF binds its cognate sites and recruits cohesin, which then folds the in-between chromatin into a loop structure.
“This readily suggested a model wherein CTCF binds its cognate sites and recruits cohesin, which then folds the in-between chromatin into a loop structure.”
The authors state this as an assumption.
In the loop extrusion model, cohesin spontaneously engages chromatin and begins extruding a DNA loop.
“In this model, cohesin spontaneously engages chromatin and begins extruding a DNA loop.”
The authors state this as an assumption.
Loop extrusion continues until cohesin spontaneously falls off or until it encounters an occupied CTCF binding site in the convergent orientation.
“Loop extrusion then continues until cohesin spontaneously falls off or until it encounters an occupied CTCF binding site in the convergent orientation.”
The authors state this as an assumption.
The orientation of the CTCF binding site determines the orientation of the CTCF protein.
“Since the orientation of the CTCF binding site determines the orientation of the CTCF protein, this may explain how an extruding cohesin complex distinguishes between convergent and divergent CTCF binding sites.”
The authors state this as an assumption.
In ΔWAPL cells, cohesin's extrusion speed does not change.
“assuming no change in cohesin's extrusion speed”
The authors state this as an assumption.
CTCF positions cohesin at its convergent cognate binding sites and cohesin holds together two strands of chromatin.
“Cohesin functions to hold together two strands of chromatin and CTCF positions cohesin at its convergent cognate binding sites as previously proposed.”
The paper relies on this without support.
The main function of cohesin in G1 is loop extrusion.
“the main function of cohesin in G1 is loop extrusion”
The paper relies on this without support.
Binding times to cognate sites are highly stochastic and exponentially distributed such that few events exhibit the mean value.
“Moreover, the binding times to cognate sites are highly stochastic and exponentially distributed such that few events exhibit the mean value.”
The paper relies on this without support.
Replenishment of cohesin involves translation of enough Rad21 protein, incorporation into cohesin complexes, loading onto chromatin, initiation and continuation of extrusion, and re-formation of TADs.
“For example, replenishment of cohesin involves translation of enough Rad21 protein, incorporation into cohesin complexes, loading onto chromatin, initiation and continuation of extrusion, and re-formation of TADs.”
Claims other papers make about this one
Each is checked against this paper’s own text: does it say what the citing paper says it does?
In the citing paper
“loop extrusion mediated by cohesin and CTCF mediates the formation of chromatin loops and self-interacting Topologically Associating Domains (TADs)”
From Neuronal DNA double-strand breaks lead to genome structural variations and 3D genome disruption in neurodegeneration (2023) · cites this paper as [81]
Citations
Cites
A 3D Map of the Human Genome at Kilobase Resolution Reveals Principles of Chromatin Looping
Rao, S. S. P., Huntley, M. H., Durand, N. C., Stamenova, E. K., Bochkov, I. D., Robinson, J. T., Sanborn, A. L., Machol, I., Omer, A. D., Lander, E. S., et al. (2014) · Cell · doi:10.1016/j.cell.2014.11.021 · Cited by 9,212
Comprehensive Mapping of Long-Range Interactions Reveals Folding Principles of the Human Genome
Lieberman-Aiden, E., van Berkum, N. L., Williams, L., Imakaev, M., Ragoczy, T., Telling, A., Amit, I., Lajoie, B. R., Sabo, P. J., Dorschner, M. O., et al. (2009) · Science · doi:10.1126/science.1181369 · Cited by 8,898
Topological domains in mammalian genomes identified by analysis of chromatin interactions
Dixon, J. R., Selvaraj, S., Yue, F., Kim, A., Li, Y., Shen, Y., Hu, M., Liu, J. S., & Ren, B. (2012) · Nature · doi:10.1038/nature11082 · Cited by 6,829
Spatial partitioning of the regulatory landscape of the X-inactivation centre
Nora, E. P., Lajoie, B. R., Schulz, E. G., Giorgetti, L., Okamoto, I., Servant, N., Piolot, T., van Berkum, N. L., Meisig, J., Sedat, J., et al. (2012) · Nature · doi:10.1038/nature11049 · Cited by 2,895
Disruptions of Topological Chromatin Domains Cause Pathogenic Rewiring of Gene-Enhancer Interactions
Lupiáñez, D. G., Kraft, K., Heinrich, V., Krawitz, P., Brancati, F., Klopocki, E., Horn, D., Kayserili, H., Opitz, J. M., Laxova, R., et al. (2015) · Cell · doi:10.1016/j.cell.2015.04.004 · Cited by 2,132
Formation of chromosomal domains by loop extrusion
Fudenberg, G., Imakaev, M., Lu, C., Goloborodko, A., Abdennur, N., & Mirny, L. A. (2016) · Cell Reports · doi:10.1016/j.celrep.2016.04.085 · Cited by 2,003
Cohesin Loss Eliminates All Loop Domains
Rao, S. S. P., Huang, S.-C., Glenn St Hilaire, B., Engreitz, J. M., Perez, E. M., Kieffer-Kwon, K.-R., Sanborn, A. L., Johnstone, S. E., Bascom, G. D., Bochkov, I. D., et al. (2017) · Cell · doi:10.1016/j.cell.2017.09.026 · Cited by 1,883
Sanborn, A. L., Rao, S. S. P., Huang, S.-C., Durand, N. C., Huntley, M. H., Jewett, A. I., Bochkov, I. D., Chinnappan, D., Cutkosky, A., Li, J., et al. (2015) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1518552112 · Cited by 1,730
Nora, E. P., Goloborodko, A., Valton, A.-L., Gibcus, J. H., Uebersohn, A., Abdennur, N., Dekker, J., Mirny, L. A., & Bruneau, B. G. (2017) · Cell · doi:10.1016/j.cell.2017.05.004 · Cited by 1,709
A general method to improve fluorophores for live-cell and single-molecule microscopy
Grimm, J. B., English, B. P., Chen, J., Slaughter, J. P., Zhang, Z., Revyakin, A. G., Patel, R. H., Macklin, J. J., Normanno, D., Singer, R. H., et al. (2015) · Nature Methods · doi:10.1038/nmeth.3256 · Cited by 1,509
Research works printed but not linked: 7
- Merkenschlager M, 2017, Annu Rev Genomics Hum Genet, 17, 1
- Rao S, 2017, bioRxiv
- Wutz G, 2017, bioRxiv
- Gassler J, 2017, bioRxiv
- Finn E, 2017, bioRxiv
- Hansen AS, 2017, bioRxiv
- Zirkel A, 2017, bioRxiv
Cited by
Sorted by citations
Transcription factors and 3D genome conformation in cell-fate decisions
Stadhouders, R., Filion, G. J. P., & Graf, T. (2019) · Nature · doi:10.1038/s41586-019-1182-7 · Cited by 530
Extensive Heterogeneity and Intrinsic Variation in Spatial Genome Organization
Finn, E. H., Pegoraro, G., Brandão, H. B., Valton, A.-L., Oomen, M. E., Dekker, J., Mirny, L., & Misteli, T. (2019) · Cell · doi:10.1016/j.cell.2019.01.020 · Cited by 459
Emerging Evidence of Chromosome Folding by Loop ExtrusionPreprint
Fudenberg, G., Abdennur, N. A., Imakaev, M., Goloborodko, A. A., & Mirny, L. A. (2017) · Cold Spring Harbor Symposia on Quantitative Biology · doi:10.1101/sqb.2017.82.034710 · Cited by 298
Distinct Classes of Chromatin Loops Revealed by Deletion of an RNA-Binding Region in CTCF
Hansen, A. S., Hsieh, T.-H. S., Cattoglio, C., Pustova, I., Saldaña-Meyer, R., Reinberg, D., Darzacq, X., & Tjian, R. (2019) · Molecular Cell · doi:10.1016/j.molcel.2019.07.039 · Cited by 279
Self-citationCohesin and CTCF control the dynamics of chromosome folding
Mach, P., Kos, P. I., Zhan, Y., Cramard, J., Gaudin, S., Tünnermann, J., Marchi, E., Eglinger, J., Zuin, J., Kryzhanovska, M., et al. (2022) · Nature Genetics · doi:10.1038/s41588-022-01232-7 · Cited by 269
CTCF mediates chromatin looping via N-terminal domain-dependent cohesin retention
Pugacheva, E. M., Kubo, N., Loukinov, D. I., Tajmul, M., Kang, S., Kovalchuk, A. L., Strunnikov, A. V., Zentner, G. E., Ren, B., & Lobanenkov, V. V. (2020) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1911708117 · Cited by 224
McCord, R. P., Kaplan, N., & Giorgetti, L. (2020) · Molecular Cell · doi:10.1016/j.molcel.2019.12.021 · Cited by 220
Wheat chromatin architecture is organized in genome territories and transcription factories
Concia, L., Veluchamy, A., Ramirez-Prado, J. S., Martin-Ramirez, A., Huang, Y., Perez, M., Domenichini, S., Rodriguez-Granados, N. R., Kim, S., Blein, T., et al. (2020) · Genome Biology · doi:10.1186/s13059-020-01998-1 · Cited by 120
Pierro, M. D., Potoyan, D. A., Wolynes, P. G., & Onuchic, J. N. (2018) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1806297115 · Cited by 163
Guided nuclear exploration increases CTCF target search efficiency
Hansen, A. S., Amitai, A., Cattoglio, C., Tjian, R., & Darzacq, X. (2019) · Nature Chemical Biology · doi:10.1038/s41589-019-0422-3 · Cited by 145
Self-citationCTCF sites display cell cycle–dependent dynamics in factor binding and nucleosome positioningPreprint
Oomen, M. E., Hansen, A. S., Liu, Y., Darzacq, X., & Dekker, J. (2019) · Genome Research · doi:10.1101/gr.241547.118 · Cited by 137
Self-citationDetermining cellular CTCF and cohesin abundances to constrain 3D genome models
Cattoglio, C., Pustova, I., Walther, N., Ho, J. J., Hantsche-Grininger, M., Inouye, C. J., Hossain, M. J., Dailey, G. M., Ellenberg, J., Darzacq, X., et al. (2019) · eLife · doi:10.7554/elife.40164 · Cited by 133
Self-citationDileep, V., Boix, C. A., Mathys, H., Marco, A., Welch, G. M., Meharena, H. S., Loon, A., Jeloka, R., Peng, Z., Bennett, D. A., et al. (2023) · Cell · doi:10.1016/j.cell.2023.08.038 · Cited by 130
STAG2 Loss Rewires Oncogenic and Developmental Programs to Promote Metastasis in Ewing Sarcoma
Adane, B., Alexe, G., Seong, B., Lu, D. Y., Hwang, E. E., Hnisz, D., Lareau, C., Ross, L., Lin, S., Cruz, F. D. D., et al. (2021) · Cancer Cell · doi:10.1016/j.ccell.2021.05.007 · Cited by 103
Lee, R., Kang, M.-K., Kim, Y.-J., Yang, B., Shim, H., Kim, S., Kim, K., Yang, C. M., Min, B.-G., Jung, W.-J., et al. (2021) · Nucleic Acids Research · doi:10.1093/nar/gkab1242 · Cited by 123
CTCF orchestrates long-range cohesin-driven V(D)J recombinational scanning
Ba, Z., Lou, J., Ye, A. Y., Dai, H., Dring, E. W., Lin, S. G., Jain, S., Kyritsis, N., Kieffer-Kwon, K.-R., Casellas, R. C., et al. (2020) · Nature · doi:10.1038/s41586-020-2578-0 · Cited by 115
Clustered CTCF binding is an evolutionary mechanism to maintain topologically associating domains
Kentepozidou, E., Aitken, S. J., Feig, C., Stefflova, K., Ibarra-Soria, X., Odom, D. T., Roller, M., & Flicek, P. (2020) · Genome biology · doi:10.1186/s13059-019-1894-x · Cited by 123
Scholz, B. A., Sumida, N., de Lima, C. D. M., Chachoua, I., Martino, M., Tzelepis, I., Nikoshkov, A., Zhao, H., Mehmood, R., Sifakis, E. G., et al. (2019) · Nature Genetics · doi:10.1038/s41588-019-0535-3 · Cited by 114
The role of chromatin loop extrusion in antibody diversification
Zhang, Y., Zhang, X., Dai, H., Hu, H., & Alt, F. W. (2022) · Nature reviews. Immunology · doi:10.1038/s41577-022-00679-3 · Cited by 106
Chromatin topology, condensates and gene regulation: shifting paradigms or just a phase?
Mir, M., Bickmore, W. A., Furlong, E. E. M., & Narlikar, G. J. (2019) · Development · doi:10.1242/dev.182766 · Cited by 113
RNA polymerase II is required for spatial chromatin reorganization following exit from mitosis
Zhang, S., Übelmesser, N., Josipović, N., Forte, G., Slotman, J. A., Chiang, M., Gothe, H. J., Gusmao, E. G., Becker, C., Altmüller, J., et al. (2021) · Science Advances · doi:10.1126/sciadv.abg8205 · Cited by 114
Cell fate decisions, transcription factors and signaling during early retinal development
Diacou, R., Nandigrami, P., Fiser, A., Liu, W., Ashery‐Padan, R., & Cvekl, A. (2022) · Progress in Retinal and Eye Research · doi:10.1016/j.preteyeres.2022.101093 · Cited by 107
CTCF as a boundary factor for cohesin-mediated loop extrusion: evidence for a multi-step mechanism
Hansen, A. S. (2020) · Nucleus · doi:10.1080/19491034.2020.1782024 · Cited by 101
Self-citationChromosome territories and the global regulation of the genome
Fritz, A. J., Sehgal, N., Pliss, A., Xu, J., & Berezney, R. (2019) · Genes Chromosomes and Cancer · doi:10.1002/gcc.22732 · Cited by 102
Wu, Q., Guo, Y., Lu, Y., Li, J., Guo, Y., & Jia, Z. (2020) · Genome biology · doi:10.1186/s13059-020-01984-7 · Cited by 84
Jpx RNA regulates CTCF anchor site selection and formation of chromosome loops
Oh, H. J., Aguilar, R., Kesner, B., Lee, H.-G., Kriz, A. J., Chu, H.-P., & Lee, J. T. (2021) · Cell · doi:10.1016/j.cell.2021.11.012 · Cited by 84
Tracking and interpreting long-range chromatin interactions with super-resolution live-cell imaging
Brandão, H. B., Gabriele, M., & Hansen, A. S. (2021) · Current Opinion in Cell Biology · doi:10.1016/j.ceb.2020.11.002 · Cited by 77
Self-citationMulti-level remodelling of chromatin underlying activation of human T cells
Bediaga, N. G., Coughlan, H. D., Johanson, T. M., Garnham, A. L., Naselli, G., Schröder, J., Fearnley, L. G., Bandala‐Sanchez, E., Allan, R. S., Smyth, G. K., et al. (2021) · Scientific Reports · doi:10.1038/s41598-020-80165-9 · Cited by 82
The role of the dynamic epigenetic landscape in senescence: orchestrating SASP expression
Dasgupta, N., Arnold, R., Equey, A., Gandhi, A., & Adams, P. D. (2024) · npj Aging · doi:10.1038/s41514-024-00172-2 · Cited by 93
Order and stochasticity in the folding of individual Drosophila genomes
Ulianov, S. V., Zakharova, V. V., Galitsyna, A. A., Kos, P. I., Polovnikov, K. E., Flyamer, I. M., Mikhaleva, E. A., Khrameeva, E. E., Germini, D., Logacheva, M. D., et al. (2021) · Nature Communications · doi:10.1038/s41467-020-20292-z · Cited by 64
Brown, J. M., Roberts, N. A., Graham, B., Waithe, D., Lagerholm, C., Telenius, J. M., De Ornellas, S., Oudelaar, A. M., Scott, C., Szczerbal, I., et al. (2018) · Nature Communications · doi:10.1038/s41467-018-06248-4 · Cited by 72
Mechanisms of Enhancer-Promoter Interactions in Higher Eukaryotes
Georgiev, P. G., & Kyrchanova, O. (2021) · International Journal of Molecular Sciences · doi:10.3390/ijms22020671 · Cited by 72
Cresswell, K. G., Stansfield, J. C., & Dozmorov, M. G. (2020) · BMC Bioinformatics · doi:10.1186/s12859-020-03652-w · Cited by 64
Profiling the epigenome using long-read sequencing
Liu, T., & Conesa, A. (2025) · Nature Genetics · doi:10.1038/s41588-024-02038-5 · Cited by 67
Soochit, W., Sleutels, F., Stik, G., Bartkuhn, M., Basu, S., Hernández, S. C., Merzouk, S., Vidal, E., Boers, R., Boers, J., et al. (2021) · Nature Cell Biology · doi:10.1038/s41556-021-00722-w · Cited by 55
Bouwman, B. A. M., & Crosetto, N. (2018) · Genes · doi:10.3390/genes9120632 · Cited by 65
Epigenetic Changes in Islets of Langerhans Preceding the Onset of Diabetes
Admin, A., Ouni, M., Saussenthaler, S., Eichelmann, F., Jähnert, M., Stadion, M., Wittenbecher, C., Rönn, T., Zellner, L., Gottmann, P., et al. (2020) · Diabetes · doi:10.2337/db20-0204 · Cited by 53
Physical and data structure of 3D genome
Huang, K., Li, Y., Shim, A. R., Nap, R. J., Agrawal, V., Virk, R. K. A., Eshein, A., Almassalha, L. M., Backman, V., & Szleifer, I. G. (2020) · Science Advances · doi:10.1126/sciadv.aay4055 · Cited by 54
Regulation of Chromatin Structure During Neural Development
Kishi, Y., & Gotoh, Y. (2018) · Frontiers in Neuroscience · doi:10.3389/fnins.2018.00874 · Cited by 51
Condensins and cohesins – one of these things is not like the other!
Skibbens, R. V. (2019) · Journal of Cell Science · doi:10.1242/jcs.220491 · Cited by 52
Heterogeneity of lipidomic profiles among lung cancer subtypes of patients
Lv, J., Gao, D., Zhang, Y., Wu, D., Shen, L., & Wang, X. (2018) · Journal of Cellular and Molecular Medicine · doi:10.1111/jcmm.13782 · Cited by 48
One-carbon epigenetics and redox biology of neurodegeneration
Coppedè, F. (2020) · Free Radical Biology and Medicine · doi:10.1016/j.freeradbiomed.2020.12.002 · Cited by 48
Shi, G., & Thirumalai, D. (2019) · Nature Communications · doi:10.1038/s41467-019-11897-0 · Cited by 48
The 3D Genome: From Structure to Function
Mohanta, T. K., Mishra, A. K., & Al‐Harrasi, A. (2021) · International Journal of Molecular Sciences · doi:10.3390/ijms222111585 · Cited by 51
Entering the Next Dimension: Plant Genomes in 3D
Sotelo-Silveira, M., Montes, R. A. C., Sotelo-Silveira, J. R., Marsch‐Martínez, N., & de Folter, S. (2018) · Trends in Plant Science · doi:10.1016/j.tplants.2018.03.014 · Cited by 45
Predicting coarse-grained chromatin polymer properties from nucleosome-level contact data
Kadam, S., Kumari, K., Vinoth, M., Dutta, S., Mitra, M. K., & Padinhateeri, R. (2023) · Nature Communications · doi:10.1038/s41467-023-39907-2 · Cited by 41
Epigenetic principles underlying epileptogenesis and epilepsy syndromes
Conboy, K., Henshall, D. C., & Brennan, G. P. (2020) · Neurobiology of Disease · doi:10.1016/j.nbd.2020.105179 · Cited by 46
Local Chromatin Motion and Transcription
Babokhov, M., Hibino, K., Itoh, Y., & Maeshima, K. (2019) · Journal of Molecular Biology · doi:10.1016/j.jmb.2019.10.018 · Cited by 42
Arc Regulates Transcription of Genes for Plasticity, Excitability and Alzheimer’s Disease
Leung, H.-W., Foo, G., & VanDongen, A. M. J. (2022) · Biomedicines · doi:10.3390/biomedicines10081946 · Cited by 41
Oocyte Quality Control: Causes, Mechanisms, and ConsequencesPreprint
Hunter, N. (2017) · Cold Spring Harbor Symposia on Quantitative Biology · doi:10.1101/sqb.2017.82.035394 · Cited by 47
SMC motor proteins extrude DNA asymmetrically and can switch directions
Barth, R., Davidson, I. F., van der Torre, J., Taschner, M., Gruber, S., Peters, J.-M., & Dekker, C. (2025) · Cell · doi:10.1016/j.cell.2024.12.020 · Cited by 40
Reawakening the Developmental Origins of Cancer Through Transposable Elements
Lynch‐Sutherland, C. F., Chatterjee, A., Stockwell, P. A., Eccles, M. R., & Macaulay, E. C. (2020) · Frontiers in Oncology · doi:10.3389/fonc.2020.00468 · Cited by 43
Chromatin Looping Links Target Genes with Genetic Risk Loci for Dermatological Traits
Shi, C., Ray-Jones, H., Ding, J., Duffus, K., Fu, Y., Gaddi, V. P., Gough, O., Hankinson, J., Martin, P., McGovern, A., et al. (2021) · Journal of Investigative Dermatology · doi:10.1016/j.jid.2021.01.015 · Cited by 32
3D spatial genome organization in the nervous system: From development and plasticity to disease
Fujita, Y., Pather, S. R., Ming, G., & Song, H. (2022) · Neuron · doi:10.1016/j.neuron.2022.06.004 · Cited by 37
Kyrchanova, O., Sabirov, M. S., Mogila, V., Kurbidaeva, A., Postika, N., Maksimenko, O. G., Schedl, P. D., & Georgiev, P. G. (2019) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1907190116 · Cited by 35
Analysis of epigenetic features characteristic of L1 loci expressed in human cells
Freeman, B., White, T., Kaul, T. K., Stow, E. C., Baddoo, M., Ungerleider, N., Morales, M. E., Yang, H., deHaro, D. L., Deininger, P. L., et al. (2022) · Nucleic Acids Research · doi:10.1093/nar/gkac013 · Cited by 33
Characterizing chromatin packing scaling in whole nuclei using interferometric microscopy
Eid, A., Eshein, A., Li, Y., Virk, R. K. A., Derway, D. V., Zhang, D., Taflove, A., & Backman, V. (2020) · Optics Letters · doi:10.1364/ol.400231 · Cited by 33
Are Parallel Proliferation Pathways Redundant?
Nussinov, R., Tsai, C., & Jang, H. (2020) · Trends in Biochemical Sciences · doi:10.1016/j.tibs.2020.03.013 · Cited by 33
Maksimenko, O. G., Фурсенко, Д. В., Belova, E., & Georgiev, P. G. (2021) · Acta Naturae · doi:10.32607/actanaturae.11206 · Cited by 32
Dynamic Crowding Regulates Transcription
Shim, A. R., Nap, R. J., Huang, K., Almassalha, L. M., Matusda, H., Backman, V., & Szleifer, I. G. (2019) · Biophysical Journal · doi:10.1016/j.bpj.2019.11.007 · Cited by 31
Smith, J. S., Craig, S. G., Liberante, F. G., Lappin, K. M., Crean, C. M., McDade, S. S., Thompson, A., Mills, K., & Savage, K. I. (2020) · Journal of Translational Medicine · doi:10.1186/s12967-020-02500-y · Cited by 31
Olfactory receptor choice: a case study for gene regulation in a multi-enhancer system
Pourmorady, A., & Lomvardas, S. (2021) · Current Opinion in Genetics & Development · doi:10.1016/j.gde.2021.11.003 · Cited by 32
Dysregulated Transcriptional Control in Prostate Cancer
Baumgart, S. J., Nevedomskaya, E., & Haendler, B. (2019) · International Journal of Molecular Sciences · doi:10.3390/ijms20122883 · Cited by 30
Dynamic regulation of CTCF stability and sub-nuclear localization in response to stress
Lehman, B. J., López-Díaz, F. J., Santisakultarm, T. P., Fang, L., Shokhirev, M. N., Diffenderfer, K. E., Manor, U., & Emerson, B. M. (2021) · PLoS Genetics · doi:10.1371/journal.pgen.1009277 · Cited by 30
Liu, Y., Zhao, N., Kanemaki, M. T., Yamamoto, Y., Sadamura, Y., Ito, Y., Tokunaga, M., Stasevich, T. J., & Kimurâ, H. (2021) · Genes to Cells · doi:10.1111/gtc.12893 · Cited by 29
Transcriptional control of interferon-stimulated genes
Babadei, O., Strobl, B., Müller, M. M., & Decker, T. (2024) · Journal of Biological Chemistry · doi:10.1016/j.jbc.2024.107771 · Cited by 28
All eukaryotic SMC proteins induce a twist of −0.6 at each DNA loop extrusion step
Janissen, R., Barth, R., Davidson, I., Taschner, M., Gruber, S., Peters, J.-M., & Dekker, C. (2024) · bioRxiv · doi:10.1126/sciadv.adt1832 · Cited by 26
Super enhancers—Functional cores under the 3D genome
Zhang, J., Yue, W., Zhou, Y., Liao, M., Chen, X., & Hua, J. (2020) · Cell Proliferation · doi:10.1111/cpr.12970 · Cited by 25
Nuclear genome organization in fungi: from gene folding to Rabl chromosomes
Torres, D. E., Reckard, A. T., Klocko, A. D., & Seidl, M. F. (2023) · FEMS Microbiology Reviews · doi:10.1093/femsre/fuad021 · Cited by 29
Transcription-induced active forces suppress chromatin motion
Shin, S., Cho, H. W., Shi, G., & Thirumalai, D. (2023) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.2307309121 · Cited by 35
Epigenetic regulation in Alzheimer’s disease: is it a potential therapeutic target?
Coppedè, F. (2021) · Expert Opinion on Therapeutic Targets · doi:10.1080/14728222.2021.1916469 · Cited by 30
Bansal, K., Michelson, D. A., Ramírez, R. N., Viny, A. D., Levine, R. L., Benoist, C. O., & Mathis, D. J. (2021) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.2110991118 · Cited by 26
The SMC5/6 complex: folding chromosomes back into shape when genomes take a break
Roy, S., Adhikary, H., & D’Amours, D. (2024) · Nucleic Acids Research · doi:10.1093/nar/gkae103 · Cited by 24
Kurotaki, D., Kikuchi, K., Cui, K., Kawase, W., Saeki, K., Fukumoto, J., Nishiyama, A., Nagamune, K., Zhao, K., Ozato, K., et al. (2022) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.2207009119 · Cited by 27
Managing the Steady State Chromatin Landscape by Nucleosome Dynamics
Ahmad, K., Henikoff, S., & Ramachandran, S. (2022) · Annual Review of Biochemistry · doi:10.1146/annurev-biochem-032620-104508 · Cited by 27
Three-dimensional genome: developmental technologies and applications in precision medicine
Li, Y., Tao, T., Du, L., & Zhu, X. M. (2020) · Journal of Human Genetics · doi:10.1038/s10038-020-0737-7 · Cited by 24
Feeling the force from within – new tools and insights into nuclear mechanotransduction
Morival, J. L. P., Hazelwood, A., & Lammerding, J. (2025) · Journal of Cell Science · doi:10.1242/jcs.263615 · Cited by 26
Halsall, J. A., Andrews, S., Krueger, F., Rutledge, C. E., Ficz, G., Reik, W., & Turner, B. M. (2021) · Scientific Reports · doi:10.1038/s41598-021-82539-z · Cited by 26
Chemical-induced phase transition and global conformational reorganization of chromatin
Wang, T., Shi, S., Shi, Y., Jiang, P., Hu, G., Ye, Q., Shi, Z., Yu, K., Wang, C., Fan, G., et al. (2023) · Nature Communications · doi:10.1038/s41467-023-41340-4 · Cited by 22
Epigenetic Regulation of Neural Stem Cells: The Emerging Role of Nucleoporins
Colussi, C., & Grassi, C. (2021) · Stem Cells · doi:10.1002/stem.3444 · Cited by 22
Impact of CAR Agonist Ligand TCPOBOP on Mouse Liver Chromatin Accessibility
Lodato, N. J., Rampersaud, A., & Waxman, D. J. (2018) · Toxicological Sciences · doi:10.1093/toxsci/kfy070 · Cited by 19
Defining the Transcriptional Ecosystem
Silveira, M. A. D., & Bilodeau, S. (2018) · Molecular Cell · doi:10.1016/j.molcel.2018.11.022 · Cited by 22
Mach, P., Kos, P., Zhan, Y., Cramard, J., Gaudin, S., Tünnermann, J., Marchi, E., Eglinger, J., Zuin, J., Kryzhanovska, M., et al. (2022) · bioRxiv · doi:10.1101/2022.03.03.482826 · Cited by 18
Vicioso‐Mantis, M., Fueyo, R., Navarro, C., Cruz-Molina, S., van IJcken, W. F. J., Rebollo, E., Rada-Iglesias, Á., & Martínez‐Balbás, M. A. (2022) · Nature Communications · doi:10.1038/s41467-022-30614-y · Cited by 22
Ng, W. S., Sielaff, H., & Zhao, Z. (2022) · International Journal of Molecular Sciences · doi:10.3390/ijms23148039 · Cited by 23
Exploring chromatin hierarchical organization via Markov State Modelling
Tan, Z. W., Guarnera, E., & Berezovsky, I. N. (2018) · PLoS Computational Biology · doi:10.1371/journal.pcbi.1006686 · Cited by 18
The Impact of Space and Time on the Functional Output of the GenomePreprint
Nollmann, M., Bennabi, I., Götz, M., & Gregor, T. (2021) · Cold Spring Harbor Perspectives in Biology · doi:10.1101/cshperspect.a040378 · Cited by 23
Crosstalk between Hepatitis B Virus and the 3D Genome Structure
Dias, J. D., Sarica, N., Cournac, A., Koszul, R., & Neuveut, C. (2022) · Viruses · doi:10.3390/v14020445 · Cited by 18
Messina, O., Raynal, F., Gurgo, J., Fiche, J.-B., Pancaldi, V., & Nöllmann, M. (2023) · Nature Communications · doi:10.1038/s41467-023-42485-y · Cited by 19
ZNF143 deletion alters enhancer/promoter looping and CTCF/cohesin geometry
Zhang, M., Huang, H., Li, J., & Wu, Q. (2024) · Cell Reports · doi:10.1016/j.celrep.2023.113663 · Cited by 20
Chrm3 Gene and M3 Muscarinic Receptors Contribute to Salt-Sensitive Hypertension
Cowley, A. W. (2018) · Hypertension · doi:10.1161/hypertensionaha.118.11494 · Cited by 19
Modulation of the high-order chromatin structure by Polycomb complexes
Guo, Y., & Wang, G. G. (2022) · Frontiers in Cell and Developmental Biology · doi:10.3389/fcell.2022.1021658 · Cited by 19
Pletenev, I. A., Bazarevich, M., Zagirova, D., Kononkova, A. D., Cherkasov, A. V., Efimova, O., Tiukacheva, E. A., Morozov, K. V., Ulianov, K. A., Komkov, D., et al. (2024) · Nucleic Acids Research · doi:10.1093/nar/gkae271 · Cited by 18
Expanded Insights Into Mechanisms of Gene Expression and Disease Related Disruptions
Smith, M., & Flodman, P. L. (2018) · Frontiers in Molecular Biosciences · doi:10.3389/fmolb.2018.00101 · Cited by 18
Packaging development: how chromatin controls transcription in zebrafish embryogenesis
Horsfield, J. A. (2019) · Biochemical Society Transactions · doi:10.1042/bst20180617 · Cited by 18
Logic and lineage impacts on functional transcription factor deployment for T-cell fate commitment
Rothenberg, E. V. (2021) · Biophysical Journal · doi:10.1016/j.bpj.2021.04.002 · Cited by 17
preciseTAD: a transfer learning framework for 3D domain boundary prediction at base-pair resolution
Stilianoudakis, S. C., Marshall, M. A., & Dozmorov, M. G. (2021) · Bioinformatics · doi:10.1093/bioinformatics/btab743 · Cited by 19
Fluorescent sensing of nucleus density assists in identifying tumor cells using an AIE luminogen
Situ, B., He, B., Chen, X., He, X., Feng, W., Ye, X., Huang, Y., Xue, X., Liu, S., Xia, Q., et al. (2020) · Chemical Engineering Journal · doi:10.1016/j.cej.2020.128183 · Cited by 17
Epigenetic Regulation of WNT3A Enhancer during Regeneration of Injured Cortical Neurons
Chang, C.-Y., Hung, J., Huang, L.-W., Li, J., Fung, K. S., Kao, C.-F., & Chen, L. (2020) · International Journal of Molecular Sciences · doi:10.3390/ijms21051891 · Cited by 16
Barutcu, A. R., Elizalde, G., Gonzalez, A. E., Soni, K., Rinn, J. L., Wagers, A. J., & Almada, A. E. (2022) · Skeletal Muscle · doi:10.1186/s13395-022-00303-x · Cited by 16
Metadata
- Authors
- Hansen, A. S., Cattoglio, C., Darzacq, X., & Tjian, R.
- Affiliations
- Howard Hughes Medical Institute (US)
- University of California, Berkeley (US)
- Corresponding author
- Hansen, Anders S.
- Venue
- Nucleus
- Publisher
- Informa UK Limited
- Published
- 2017-12-14
- Volume
- 9
- Issue
- 1
- Pages
- 20-32
- ISSN
- 1949-1034 (ISSN-L)
- 1949-1042
- PMC
- PMC5990973
- OpenAlex
- W2767110090
- Semantic Scholar
- 105d85c2ba436e44587d8b60f1d342ae96d7e316
- Cited by
- 266
- References
- 78
- Citations by year
- 2026: 14 · 2025: 24 · 2024: 31 · 2023: 24 · 2022: 42 · 2021: 35 · 2020: 44 · 2019: 32 · 2018: 17 · 2017: 2
- Type
- journal article
- Language
- en
- Open access
- gold
- doi.org
- Licence
- Locations
- Nucleus (publishedVersion, cc-by)
- Europe PMC (PubMed Central) (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by)
- PubMed (publishedVersion)
- eScholarship (California Digital Library) (submittedVersion)
- eScholarship (California Digital Library) (submittedVersion, cc-by)
- Funders
- California Institute of Regenerative Medicine (LA1-08013)
- Siebel Stem Cell Institute
- National Institutes of Health (DK 107980)
- National Institute of Diabetes and Digestive and Kidney Diseases (U54DK107980)
- National Institute of Biomedical Imaging and Bioengineering (U01EB021236)
- Topics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Genomics and Chromatin Dynamics
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Chromatin Remodeling and Cancer
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Nuclear Structure and Function
- Keywords
- topologically associating domains, chromatin looping, loop extrusion, cohesin, CTCF, 3D genome organization, enhancer-promoter interactions, loop dynamics, cell cycle, Hi-C, polymer simulation, single-molecule imaging
- MeSH terms
- Animals, Chromatin, Humans, Models, Molecular, Chromatin Assembly and Disassembly
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
A language model drew the claims from the paper on 2026-10-10, under version 3 of the claim definition (model deepseek-v4.1-flash, prompt extract-v3).
A second model labelled each claim on 2026-10-10 (model jev-1.13-20260917, definition revision gold-guideline-v0.2).
Cited sources are checked with a language model’s help (gpt-6-sol).
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
