

The DOI matches its Crossref record; 65 of the 65 references it cites were found in a registry or an index; none of the 47 sources its claims cite is checked for support yet.
RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis
Open accessAbstract
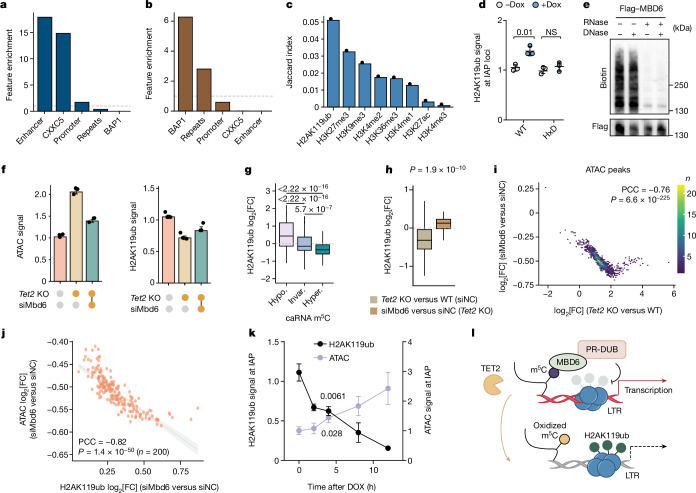
Mutation of tet methylcytosine dioxygenase 2 (encoded by TET2 ) drives myeloid malignancy initiation and progression 1–3 . TET2 deficiency is known to cause a globally opened chromatin state and activation of genes contributing to aberrant haematopoietic stem cell self-renewal 4,5 . However, the open chromatin observed in TET2-deficient mouse embryonic stem cells, leukaemic cells and haematopoietic stem and progenitor cells 5 is inconsistent with the designated role of DNA 5-methylcytosine oxidation of TET2. Here we show that chromatin-associated retrotransposon RNA 5-methylcytosine (m 5 C) can be recognized by the methyl-CpG-binding-domain protein MBD6, which guides deubiquitination of nearby monoubiquitinated Lys119 of histone H2A (H2AK119ub) to promote an open chromatin state. TET2 oxidizes m 5 C and antagonizes this MBD6-dependent H2AK119ub deubiquitination. TET2 depletion thereby leads to globally decreased H2AK119ub, more open chromatin and increased transcription in stem cells. TET2- mutant human leukaemia becomes dependent on this gene activation pathway, with MBD6 depletion selectively blocking proliferation of TET2 -mutant leukaemic cells and largely reversing the haematopoiesis defects caused by Tet2 loss in mouse models. Together, our findings reveal a chromatin regulation pathway by TET2 through retrotransposon RNA m 5 C oxidation and identify the downstream MBD6 protein as a feasible target for developing therapies specific against TET2 mutant malignancies.
Overview
CoChat Summary
Written by AI from the paper’s full text.
TL;DR
TET2 oxidizes chromatin-associated retrotransposon RNA m5C, and TET2 loss increases m5C that is read by MBD6 to recruit PR-DUB/BAP1, deubiquitinate H2AK119ub, open chromatin, and activate leukaemogenic genes. Targeting MBD6 reverses Tet2-loss phenotypes in mouse HSPCs and impairs TET2-mutant leukaemia cell growth and xenograft progression.
Key findings
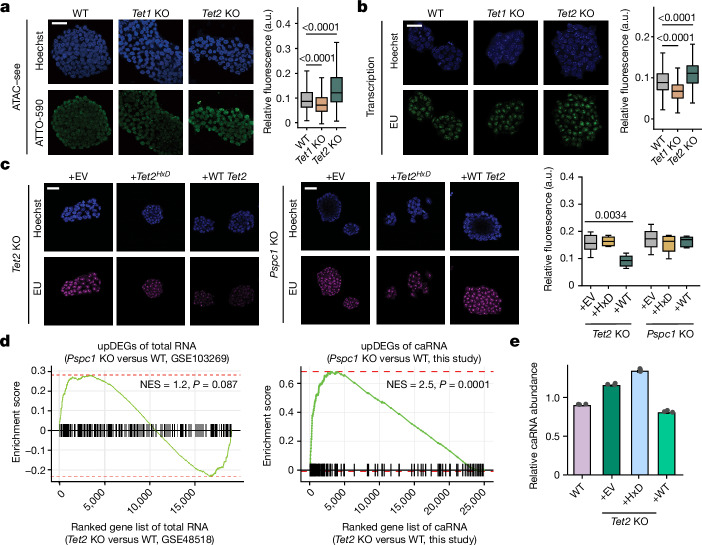
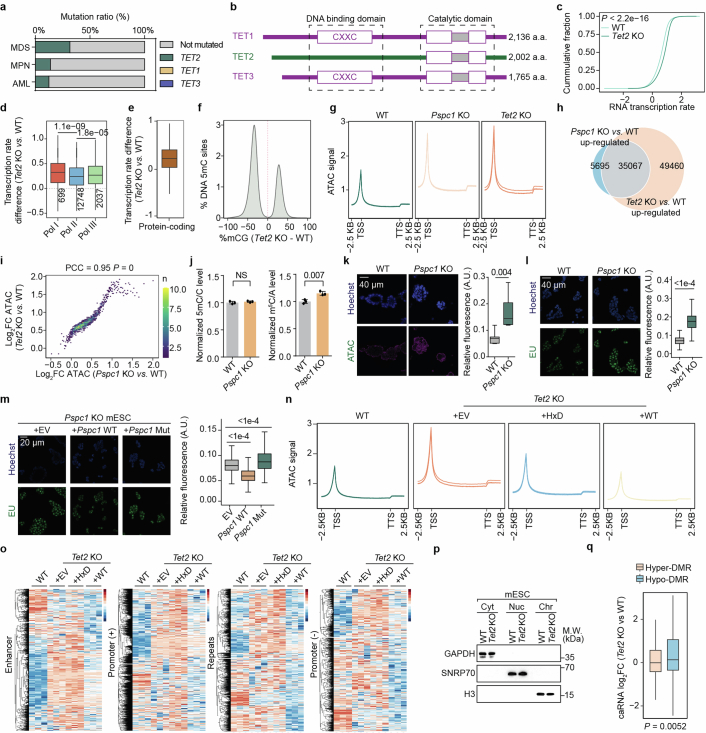
- In mES cells, Tet2 KO increased chromatin accessibility and global transcription; WT Tet2, but not catalytically dead HxD, restored repression in Tet2-KO but not Pspc1-KO cells, implicating PSPC1-dependent RNA oxidation.
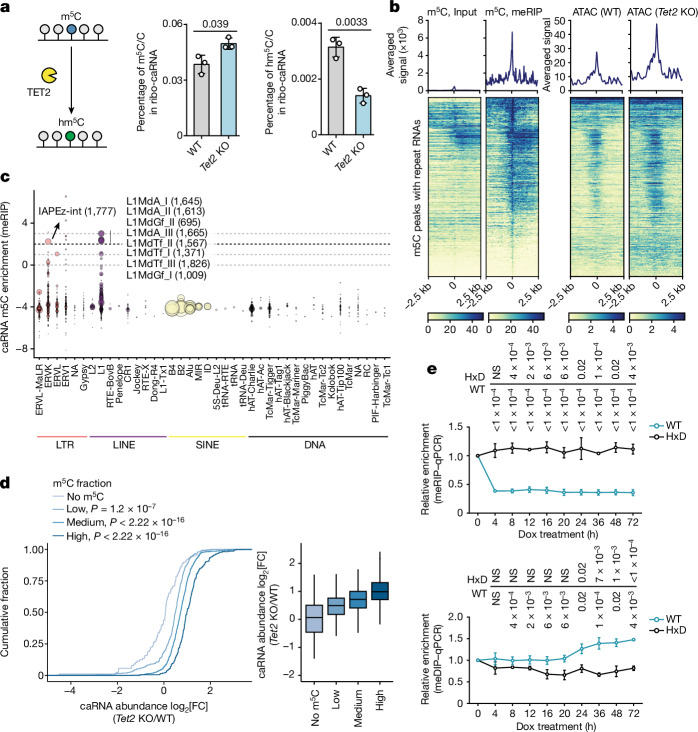
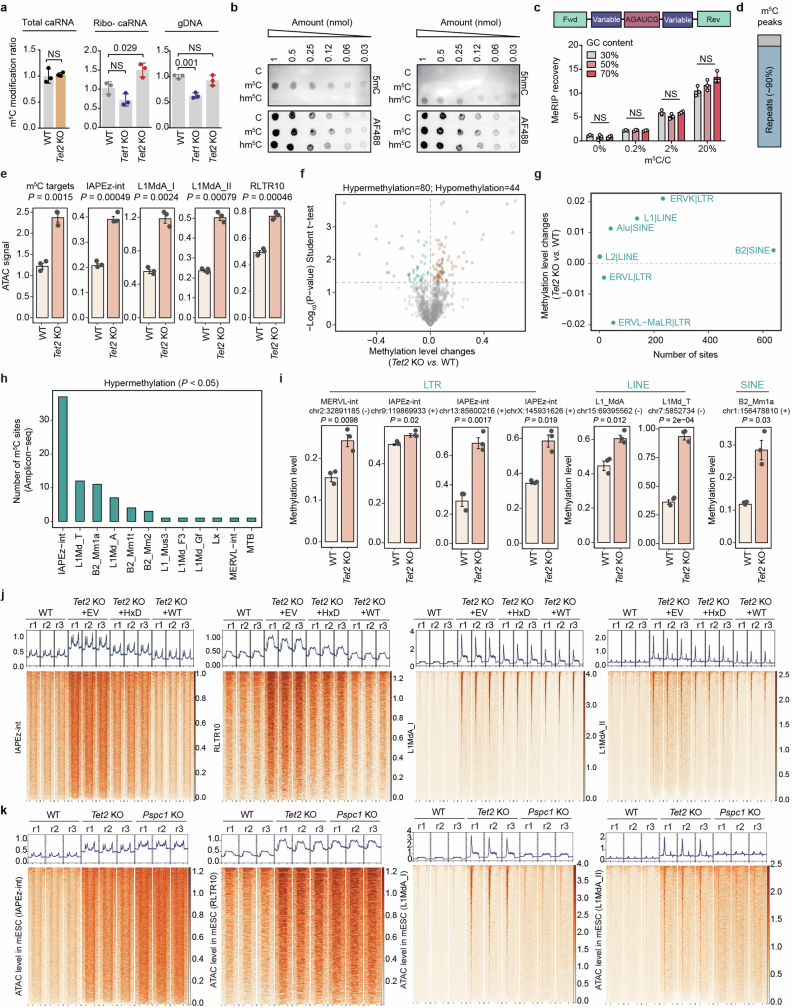
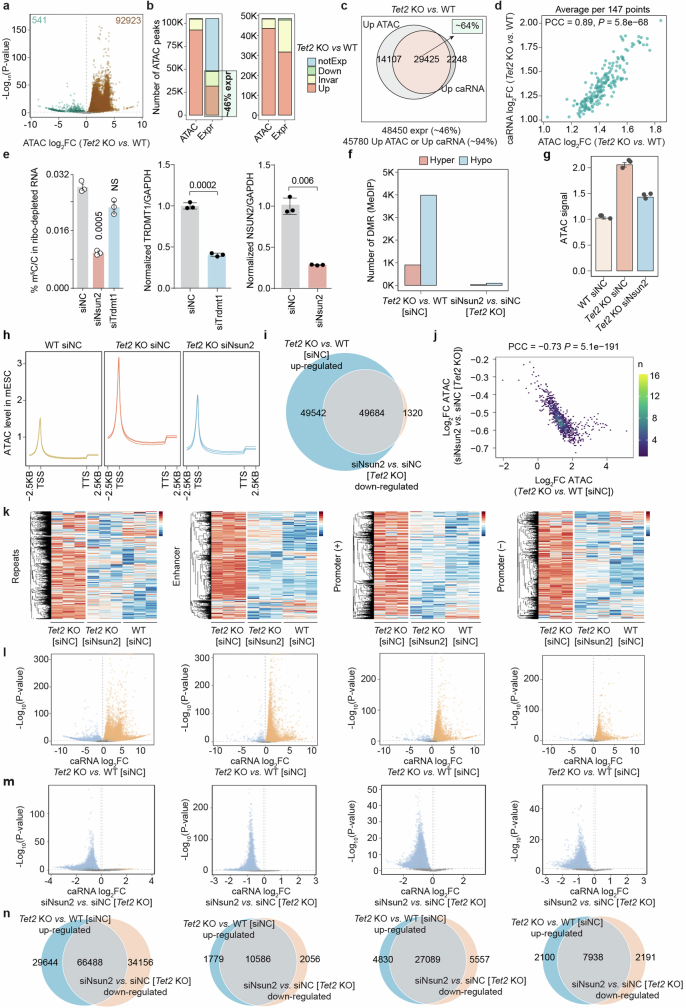
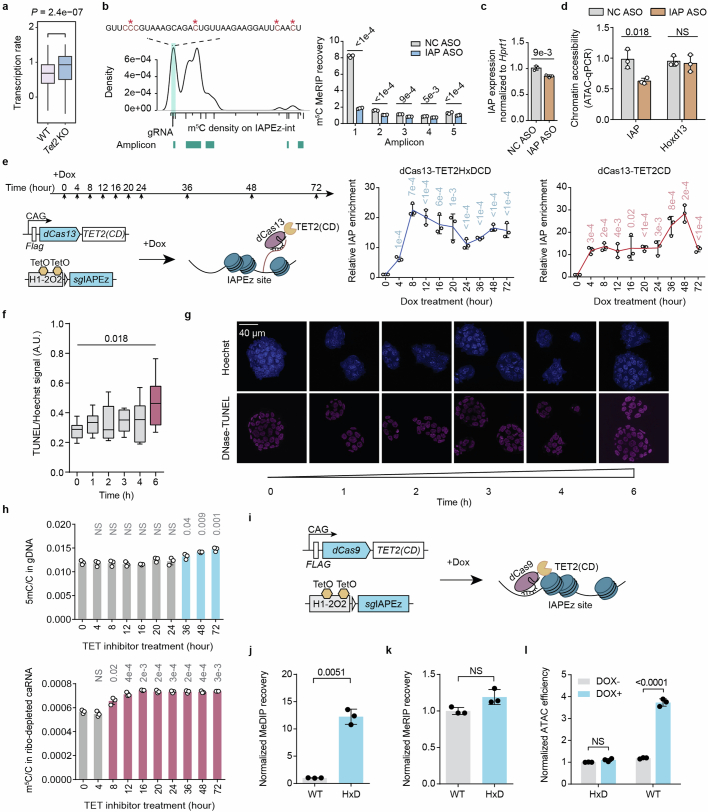
- caRNA m5C is a TET2 substrate: Tet2 KO increased caRNA m5C and decreased hm5C; m5C peaks were enriched in repeat RNA, especially LTR/LINE families such as IAP. Nsun2 depletion reduced caRNA m5C by approximately 70% and closed chromatin; dCas13–TET2-CD targeting IAP reduced RNA m5C and increased local DNA 5mC.
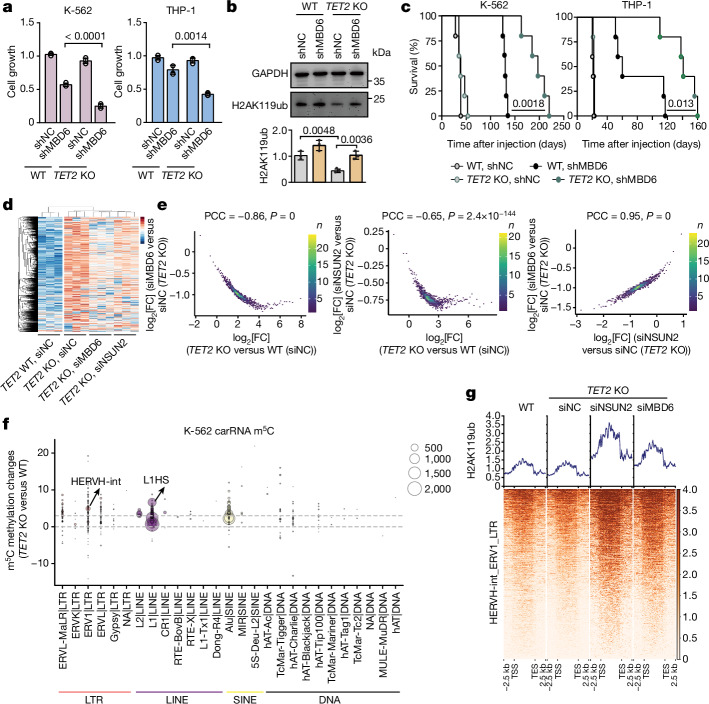
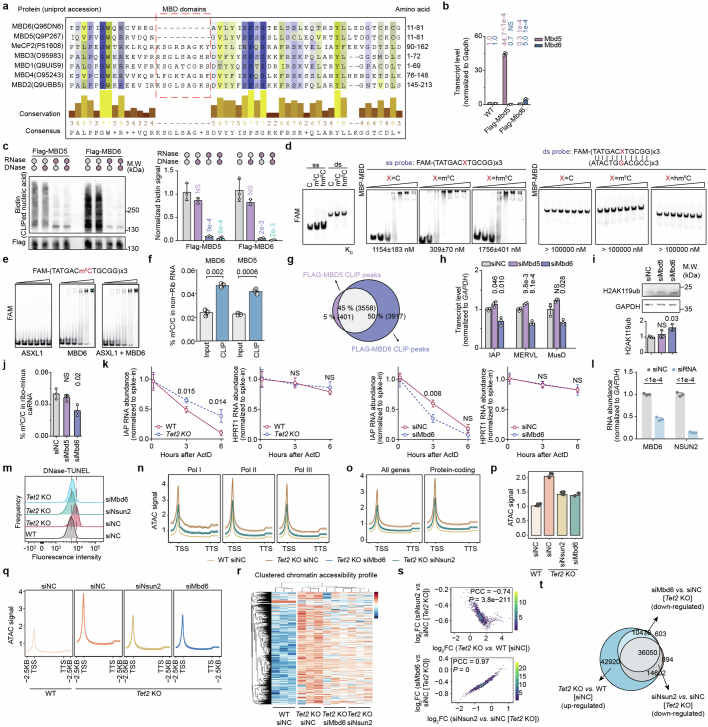
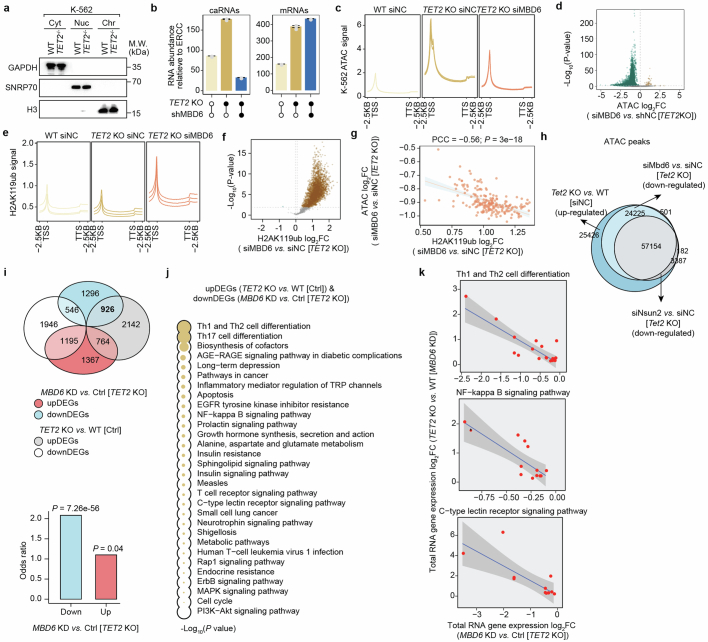
- MBD6 reads m5C RNA and recruits PR-DUB: H2AK119ub ranked top among correlated marks; approximately 37% of ATAC–seq peaks were marked with H2AK119ub, H2AK119ub was downregulated in around 89% of those regions after Tet2 KO, and approximately 85% of regions with higher ATAC signals overlapped H2AK119ub loss. Mbd6 KD reversed chromatin opening and H2AK119ub loss.
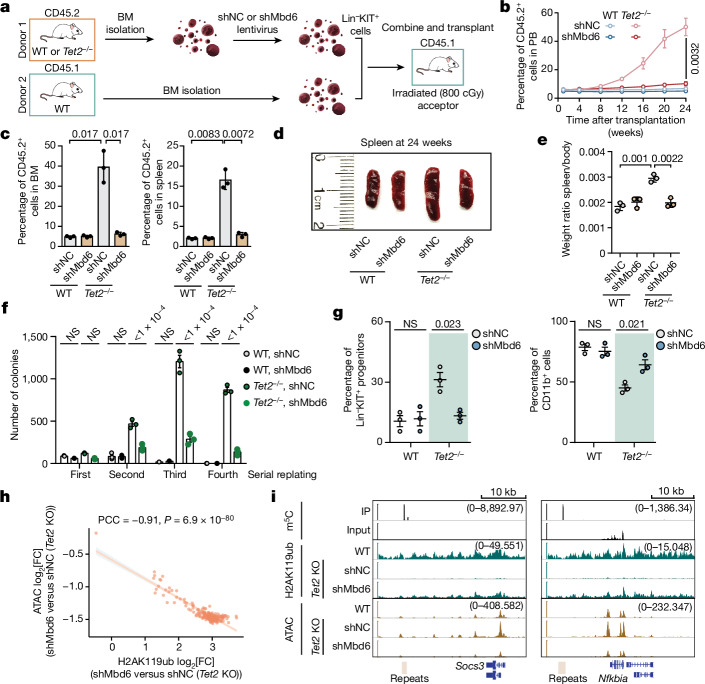
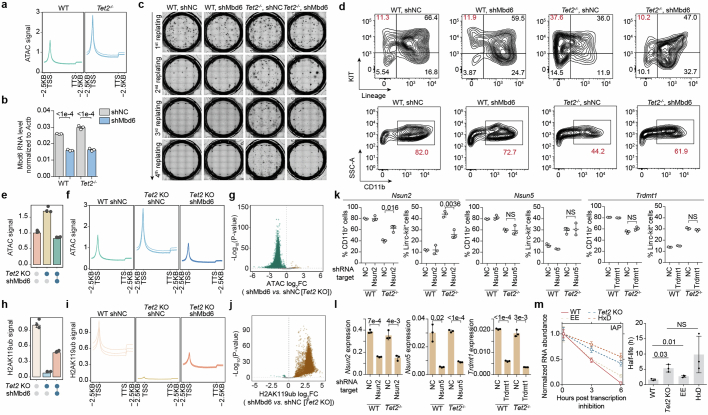
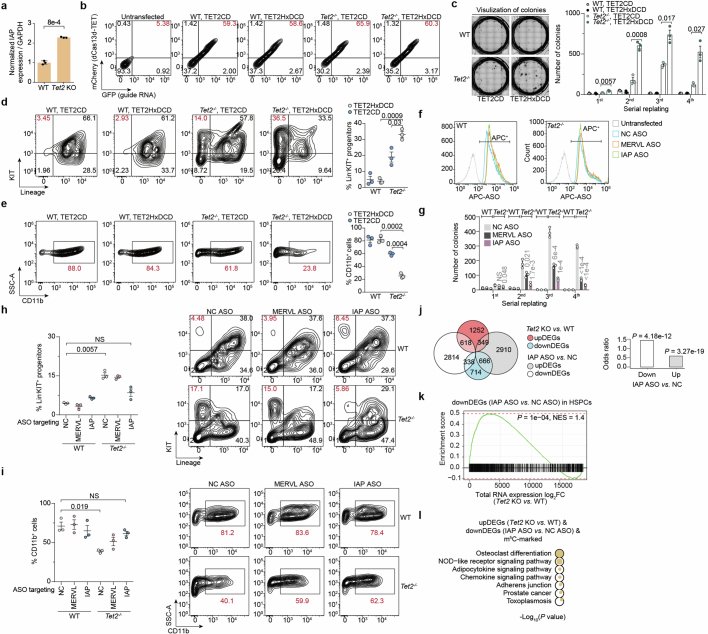
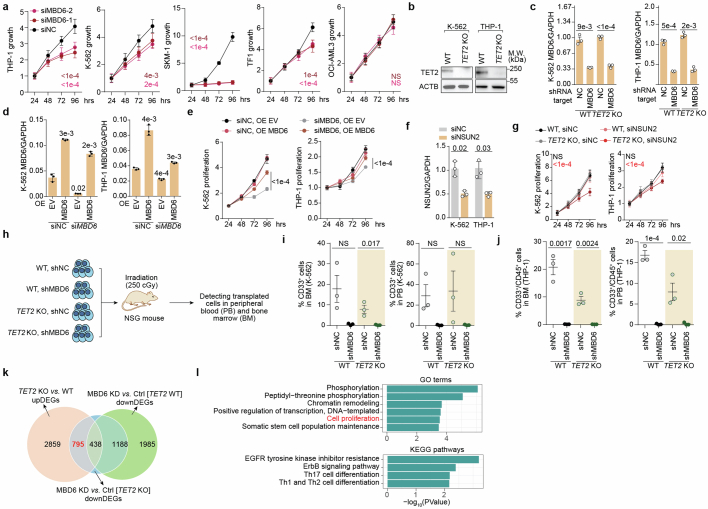
- In vivo, Tet2−/− + shNC HSPC chimerism reached around 50% at 6 months versus around 5% with shMbd6; Mbd6 KD rescued splenomegaly and replating/differentiation defects. MBD6 KD blocked proliferation of TET2-mutant SKM-1 and TET2-KO K-562/THP-1 cells; in NSG xenografts, TET2-KO + shMBD6 recipients survived longer (reported ranges 125–135 days or 163–220 days).
Methods
- Mouse mES cells (WT, Tet2-KO, Pspc1-KO), mouse HSPCs (Lin−KIT+), human leukaemia cell lines (SKM-1, K-562, THP-1 and others), NSG xenotransplantation, and competitive BM transplantation assays.
- Assays included ATAC–seq/ATAC–see, RNA-seq/caRNA-seq, m5C meRIP–seq, UHPLC–MS/MS, RNA bisulfite amplicon sequencing, meDIP–seq, CUT&Tag, CLIP/PAR-CLIP, EMSA, dCas13/dCas9 tethering, ASO treatment, proliferation/colony formation, and flow cytometry.
- Main analyses used spike-in-normalized genome-wide data, differential expression/accessibility/methylation, correlation analyses, and survival comparisons; most experiments used n = 3 biological replicates unless otherwise noted.
Limitations
- The paper states that whether the oxidation product hm5C further promotes caRNA degradation remains to be investigated.
- Evident from the text: mechanistic and in vivo evidence comes mainly from mouse mES cells/HSPCs and human leukaemia cell lines/xenografts, not primary TET2-mutant patient samples.
- Evident from the text: MBD6 KD also suppressed transplanted TET2 WT human cells in vivo, so selectivity for TET2-mutant disease is not absolute; the study focused on MBD6, although MBD5 may have important roles in other cell types.
Model-written summary. Check it against the paper before relying on it.
Integrity signals
Registry
Cites
Statistics
Figures
Verification
Claims the paper makes
123 Own result · 27 Own interpretation · 24 Own method · 19 Check pending · 7 Not checked yet · 1 No full text of the sources
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
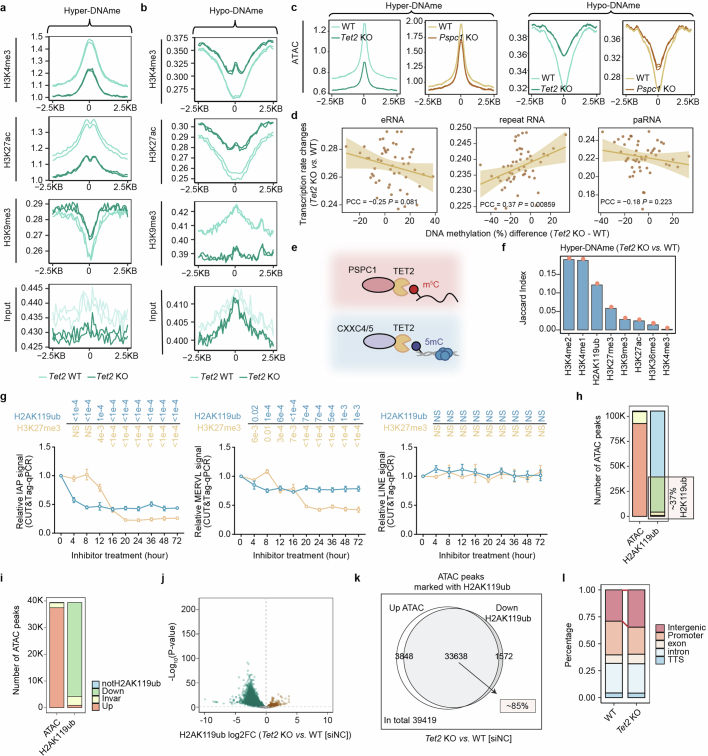
“Approximately 37% of ATAC–seq peaks were marked with H2AK119ub (Extended Data Fig. 5h)”
§ RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis > MBD6 binds to RNA m5C to recruit PR-DUB
plain- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: unclear — It is unclear whether the paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“We observed a negative correlation between changes in enhancer transcription and DNA methylation resulting from Tet2 KO in mES cells, which contrasts with the pattern observed for repeat RNA (Extended Data Fig. 5d).”
§ RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis > caRNA m5C oxidation by TET2
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Only Nsun2 depletion caused an approximately 70% decrease in caRNA m5C abundance (Extended Data Fig. 3e)”
§ RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis > caRNA m5C oxidation by TET2
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“The elevated caRNA expression correlates with DNA hypomethylated regions instead of hypermethylated regions”
§ RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis > Main
plainstates an association- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
A result the paper reports from its own data — it cites no other source for it, so there is none to check. The quote shows it is in the paper.
In the paper
“Tet2 depletion led to increased caRNA IAP m5C levels (Extended Data Fig. 2f–i)”
§ RNA m5C oxidation by TET2 regulates chromatin state and leukaemogenesis > caRNA m5C oxidation by TET2
plainstates a cause- Asserted: passes — The authors put it forward as true.
- Checkable: passes — It can be checked against evidence.
- Load-bearing: passes — The paper’s conclusions depend on it.
- Based: passes — The paper gives a reason why it holds.
- It may state two separate claims as one. 44
- Probably not a substantial claim. 33
Create a free account to see these claims.
Create a free account to see these assumptions.
122 more claims
Create a free account to see all 201 claims and to verify the 40 references still open.
Citations
Cites
Moderated estimation of fold change and dispersion for RNA-seq data with DESeq2
Love, M. I., Huber, W., & Anders, S. (2014) · Genome Biology · doi:10.1186/s13059-014-0550-8 · Cited by 95,106
Trimmomatic: a flexible trimmer for Illumina sequence data
Bolger, A. M., Lohse, M., & Usadel, B. (2014) · Bioinformatics · doi:10.1093/bioinformatics/btu170 · Cited by 65,548
Fast gapped-read alignment with Bowtie 2
Langmead, B., & Salzberg, S. L. (2012) · Nature Methods · doi:10.1038/nmeth.1923 · Cited by 56,400
Robinson, M. D., McCarthy, D. J., & Smyth, G. K. (2010) · Bioinformatics · doi:10.1093/bioinformatics/btp616 · Cited by 41,364
featureCounts: an efficient general purpose program for assigning sequence reads to genomic features
Liao, Y., Smyth, G. K., & Shi, W. (2014) · Bioinformatics · doi:10.1093/bioinformatics/btt656 · Cited by 27,219
Ultrafast and memory-efficient alignment of short DNA sequences to the human genome.
Langmead, B., Trapnell, C., Pop, M., & Salzberg, S. L. (2009) · Genome Biology · doi:10.1186/gb-2009-10-3-r25 · Cited by 21,849
HTSeq—a Python framework to work with high-throughput sequencing data
Anders, S., Pyl, P. T., & Huber, W. (2015) · Bioinformatics · doi:10.1093/bioinformatics/btu638 · Cited by 21,464
Model-based Analysis of ChIP-Seq (MACS)
Zhang, Y., Liu, T., Meyer, C. A., Eeckhoute, J., Johnson, D. S., Bernstein, B. E., Nusbaum, C., Myers, R. M., Brown, M., Li, W., et al. (2008) · Genome Biology · doi:10.1186/gb-2008-9-9-r137 · Cited by 18,386
Twelve years of SAMtools and BCFtools
Danecek, P., Bonfield, J., Liddle, J., Marshall, J., Ohan, V., Pollard, M., Whitwham, A., Keane, T., McCarthy, S., Davies, R. M., et al. (2021) · GigaScience · doi:10.1093/gigascience/giab008 · Cited by 16,449
Graph-based genome alignment and genotyping with HISAT2 and HISAT-genotype
Kim, D., Paggi, J. M., Park, C., Bennett, C., & Salzberg, S. L. (2019) · Nature Biotechnology · doi:10.1038/s41587-019-0201-4 · Cited by 15,022
Conversion of 5-Methylcytosine to 5-Hydroxymethylcytosine in Mammalian DNA by MLL Partner TET1
Tahiliani, M., Koh, K. P., Shen, Y., Pastor, W. A., Bandukwala, H., Brudno, Y., Agarwal, S., Iyer, L. M., Liu, D. R., Aravind, L., et al. (2009) · Science · doi:10.1126/science.1170116 · Cited by 5,836
GENCODE reference annotation for the human and mouse genomes
Frankish, A., Diekhans, M., Ferreira, A.-M., Johnson, R., Jungreis, I., Loveland, J. E., Mudge, J. M., Sisu, C., Wright, J. C., Armstrong, J. C., et al. (2018) · Nucleic Acids Research · doi:10.1093/nar/gky955 · Cited by 3,006
Figueroa, M. E., Abdel-Wahab, O., Lu, C., Ward, P. S., Patel, J., Shih, A., Li, Y., Bhagwat, N., Vasanthakumar, A., Fernandez, H. F., et al. (2010) · Cancer Cell · doi:10.1016/j.ccr.2010.11.015 · Cited by 2,766
Self-citationWard, P. S., Patel, J., Wise, D. R., Abdel-Wahab, O., Bennett, B. D., Coller, H. A., Cross, J. R., Fantin, V. R., Hedvat, C. V., Perl, A. E., et al. (2010) · Cancer Cell · doi:10.1016/j.ccr.2010.01.020 · Cited by 2,020
Mutation in TET2 in Myeloid Cancers
Delhommeau, F., Dupont, S., Valle, V. D., James, C., Trannoy, S., Massé, A., Kosmider, O., Le Couedic, J.-P., Robert, F., Alberdi, A., et al. (2009) · New England Journal of Medicine · doi:10.1056/nejmoa0810069 · Cited by 1,776
Role of histone H2A ubiquitination in Polycomb silencing
Wang, H., Wang, L., Erdjument-Bromage, H., Vidal, M., Tempst, P., Jones, R. S., & Zhang, Y. (2004) · Nature · doi:10.1038/nature02985 · Cited by 1,663
Self-citationTet2 loss leads to increased hematopoietic stem cell self-renewal and myeloid transformation
Moran-Crusio, K., Reavie, L., Shih, A., Abdel-Wahab, O., Ndiaye-Lobry, D., Lobry, C., Figueroa, M. E., Vasanthakumar, A., Patel, J., Zhao, X., et al. (2011) · Cancer Cell · doi:10.1016/j.ccr.2011.06.001 · Cited by 1,339
Self-citationThe role of Tet3 DNA dioxygenase in epigenetic reprogramming by oocytes
Gu, T., Guo, F., Yang, H., Wu, H.-P., Xu, G., Liu, W., Xie, Z.-G., Shi, L., He, X., Jin, S., et al. (2011) · Nature · doi:10.1038/nature10443 · Cited by 1,195
5-methylcytosine promotes mRNA export — NSUN2 as the methyltransferase and ALYREF as an m5C reader
Yang, X., Yang, Y., Sun, B.-F., Chen, Y.-S., Xu, J.-W., Lai, W.-Y., Li, A., Wang, X., Bhattarai, D. P., Xiao, W., et al. (2017) · Cell Research · doi:10.1038/cr.2017.55 · Cited by 1,062
Self-citationTETonic shift: biological roles of TET proteins in DNA demethylation and transcription
Pastor, W. A., Aravind, L., & Rao, A. (2013) · Nature Reviews Molecular Cell Biology · doi:10.1038/nrm3589 · Cited by 897 · cited 1×
“TET2 is also unique among TET enzymes in that it is not covalently linked to the zinc-finger CXXC domain protein CXXC4 or CXXC5 12–14 ; the interaction between TET2 and CXXC4/CXXC5 is critical for DNA binding by TET2 15 (Extended Data Fig.”
de Napoles, M., Mermoud, J. E., Wakao, R., Tang, Y. A., Endoh, M., Appanah, R., Nesterova, T. B., Silva, J., Otte, A. P., Vidal, M., et al. (2004) · Developmental Cell · doi:10.1016/j.devcel.2004.10.005 · Cited by 888
Tet2 is required to resolve inflammation by recruiting Hdac2 to specifically repress IL-6
Zhang, Q., Zhao, K., Shen, Q., Han, Y., Gu, Y., Li, X., Zhao, D., Liu, Y., Wang, C., Zhang, X., et al. (2015) · Nature · doi:10.1038/nature15252 · Cited by 807
Histone H2A deubiquitinase activity of the Polycomb repressive complex PR-DUB
Scheuermann, J. C., de Ayala Alonso, A. G., Oktaba, K., Ly-Hartig, N., McGinty, R. K., Fraterman, S., Wilm, M., Muir, T. W., & Müller, J. (2010) · Nature · doi:10.1038/nature08966 · Cited by 792
Liu, J., Dou, X., Chen, C., Chen, C., Liu, C., Xu, M. M., Zhao, S., Shen, B., Gao, Y., Han, D., et al. (2020) · Science · doi:10.1126/science.aay6018 · Cited by 709
Self-citationAcquired mutations in TET2 are common in myelodysplastic syndromes
Langemeijer, S. M. C., Kuiper, R. P., Berends, M., Knops, R., Aslanyan, M. G., Massop, M., Stevens-Linders, E., van Hoogen, P., van Kessel, A. G., Raymakers, R. A. P., et al. (2009) · Nature Genetics · doi:10.1038/ng.391 · Cited by 680
Li, Z., Cai, X., Cai, C.-L., Wang, J., Zhang, W., Petersen, B. E., Yang, F.-C., & Xu, M. (2011) · Blood · doi:10.1182/blood-2010-12-325241 · Cited by 671
Self-citationGlucose-regulated phosphorylation of TET2 by AMPK reveals a pathway linking diabetes to cancer
Wu, D., Hu, D., Chen, H., Shi, G., Fetahu, I. S., Wu, F., Rabidou, K., Fang, R., Tan, L., Xu, S., et al. (2018) · Nature · doi:10.1038/s41586-018-0350-5 · Cited by 477
Self-citationTranscriptome-wide distribution and function of RNA hydroxymethylcytosine
Delatte, B., Wang, F., Ngoc, L. V., Collignon, E., Bonvin, E., Deplus, R., Calonne, E., Hassabi, B., Putmans, P., Awe, S., et al. (2016) · Science · doi:10.1126/science.aac5253 · Cited by 411
Tet-Mediated Formation of 5-Hydroxymethylcytosine in RNA
Fu, L., Guerrero, C. R., Zhong, N., Amato, N. J., Liu, Y., Liu, S., Cai, Q., Ji, D., Jin, S.-G., Niedernhofer, L. J., et al. (2014) · Journal of the American Chemical Society · doi:10.1021/ja505305z · Cited by 404
Self-citationThe RNA m6A reader YTHDC1 silences retrotransposons and guards ES cell identity
Liu, J., Gao, M., He, J., Wu, K., Lin, S., Jin, L., Chen, Y., Liu, H., Shi, J., Wang, X., et al. (2021) · Nature · doi:10.1038/s41586-021-03313-9 · Cited by 374
Self-citationModulation of TET2 expression and 5-methylcytosine oxidation by the CXXC domain protein IDAX
Ko, M., An, J., Bandukwala, H. S., Chavez, L., Äijö, T., Pastor, W. A., Segal, M. F., Li, H., Koh, K. P., Lähdesmäki, H., et al. (2013) · Nature · doi:10.1038/nature12052 · Cited by 373
METTL3 regulates heterochromatin in mouse embryonic stem cells
Xu, W., Li, J., He, C., Wen, J., Ma, H., Rong, B., Diao, J., Wang, L., Wang, J., Wu, F., et al. (2021) · Nature · doi:10.1038/s41586-021-03210-1 · Cited by 367
Self-citationTet1 Regulates Adult Hippocampal Neurogenesis and Cognition
Zhang, R.-R., Cui, Q., Murai, K., Lim, Y. C., Smith, Z. D., Jin, S., Ye, P., Rosa, L., Lee, Y. K., Wu, H.-P., et al. (2013) · Cell stem cell · doi:10.1016/j.stem.2013.05.006 · Cited by 365
Rapid and accurate alignment of nucleotide conversion sequencing reads with HISAT-3NPreprint
Zhang, Y., Park, C., Bennett, C. G., Thornton, M. A., & Kim, D. (2021) · Genome Research · doi:10.1101/gr.275193.120 · Cited by 349
Hon, G. C., Song, C.-X., Du, T., Jin, F., Selvaraj, S., Lee, A. Y., Yen, C.-A., Ye, Z., Mao, S.-Q., Wang, B.-A., et al. (2014) · Molecular Cell · doi:10.1016/j.molcel.2014.08.026 · Cited by 344
Self-citationJankowska, A. M., Szpurka, H., Tiu, R. V., Makishima, H., Afable, M., Huh, J., O'Keefe, C. L., Ganetzky, R., McDevitt, M. A., & Maciejewski, J. P. (2009) · Blood · doi:10.1182/blood-2009-02-205690 · Cited by 331
Lienhard, M., Grimm, C., Morkel, M., Herwig, R., & Chávez, L. (2013) · Bioinformatics · doi:10.1093/bioinformatics/btt650 · Cited by 328
m6A RNA methylation regulates the fate of endogenous retroviruses
Chelmicki, T., Roger, E., Teissandier, A., Dura, M., Bonneville, L., Rucli, S., Dossin, F., Fouassier, C., Lameiras, S., & Bourc’his, D. (2021) · Nature · doi:10.1038/s41586-020-03135-1 · Cited by 307
Cooper, S., Grijzenhout, A., Underwood, E., Ancelin, K., Zhang, T., Nesterova, T. B., Anil-Kirmizitas, B., Bassett, A., Kooistra, S. M., Agger, K., et al. (2016) · Nature Communications · doi:10.1038/ncomms13661 · Cited by 296
FTO mediates LINE1 m 6 A demethylation and chromatin regulation in mESCs and mouse development
Wei, J., Yu, X., Yang, L., Liu, X., Gao, B., Huang, B., Dou, X., Liu, J., Zou, Z., Cui, X.-L., et al. (2022) · Science · doi:10.1126/science.abe9582 · Cited by 294
Self-citationConnections between TET proteins and aberrant DNA modification in cancer
Huang, Y., & Rao, A. (2014) · Trends in Genetics · doi:10.1016/j.tig.2014.07.005 · Cited by 277
ATAC-see reveals the accessible genome by transposase-mediated imaging and sequencing
Chen, X., Shen, Y., Draper, W. E., Buenrostro, J. D., Litzenburger, U. M., Cho, S. W., Satpathy, A. T., Carter, A. C., Ghosh, R. P., East-Seletsky, A., et al. (2016) · Nature Methods · doi:10.1038/nmeth.4031 · Cited by 264
Wuarin, J., & Schibler, U. (1994) · Molecular and Cellular Biology · doi:10.1128/mcb.14.11.7219 · Cited by 244
Tet2 promotes pathogen infection-induced myelopoiesis through mRNA oxidation
Shen, Q., Zhang, Q., Shi, Y., Shi, Q., Jiang, Y., Gu, Y., Li, Z., Li, X., Zhao, K., Wang, C., et al. (2018) · Nature · doi:10.1038/nature25434 · Cited by 243
Guallar, D., Bi, X., Pardavila, J. A., Huang, X., Saenz, C., Shi, X., Zhou, H., Faiola, F., Ding, J., Haruehanroengra, P., et al. (2018) · Nature Genetics · doi:10.1038/s41588-018-0060-9 · Cited by 190
Self-citationm5C modification of mRNA serves a DNA damage code to promote homologous recombination
Chen, H., Yang, H., Zhu, X., Yadav, T., Ouyang, J., Truesdell, S. S., Tan, J., Wang, Y., Duan, M., Wei, L., et al. (2020) · Nature Communications · doi:10.1038/s41467-020-16722-7 · Cited by 179
Self-citationUltrafast bisulfite sequencing detection of 5-methylcytosine in DNA and RNA
Dai, Q., Ye, C., Irkliyenko, I., Wang, Y., Sun, H., Gao, Y., Liu, Y., Beadell, A. V., Perea, J., Goel, A., et al. (2024) · Nature Biotechnology · doi:10.1038/s41587-023-02034-w · Cited by 172
Self-citationDaou, S., Hammond-Martel, I., Mashtalir, N., Barbour, H., Gagnon, J., Iannantuono, N. G., Nkwe, N. S., Motorina, A., Pak, H., Yu, H., et al. (2015) · Journal of Biological Chemistry · doi:10.1074/jbc.m115.661553 · Cited by 146
Paradoxical association of TET loss of function with genome-wide DNA hypomethylation
López-Moyado, I. F., Tsagaratou, A., Yuita, H., Seo, H., Delatte, B., Heinz, S., Benner, C., & Rao, A. (2019) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1903059116 · Cited by 131
The Human Proteins MBD5 and MBD6 Associate with Heterochromatin but They Do Not Bind Methylated DNA
Laget, S., Joulie, M., Le Masson, F., Sasai, N., Christians, E., Pradhan, S., Roberts, R. J., & Defossez, P.-A. (2010) · PLoS ONE · doi:10.1371/journal.pone.0011982 · Cited by 110
TET2-mediated mRNA demethylation regulates leukemia stem cell homing and self-renewal
Li, Y., Xue, M., Deng, X., Dong, L., Nguyen, L. X. T., Ren, L., Han, L., Li, C., Xue, J., Zhao, Z., et al. (2023) · Cell Stem Cell · doi:10.1016/j.stem.2023.07.001 · Cited by 110
Self-citationMBD5 and MBD6 interact with the human PR‐DUB complex through their methyl‐CpG‐binding domain
Baymaz, H. I., Fournier, A., Laget, S., Ji, Z., Jansen, P. W. T. C., Smits, A. H., Ferry, L., Mensinga, A., Poser, I., Sharrocks, A., et al. (2014) · PROTEOMICS · doi:10.1002/pmic.201400013 · Cited by 109
Dou, X., Xiao, Y., Shen, C., Wang, K., Wu, T., Liu, C., Li, Y., Yu, X., Liu, J., Dai, Q., et al. (2023) · Nature Cell Biology · doi:10.1038/s41556-023-01213-w · Cited by 100
Self-citationMutations along a TET2 active site scaffold stall oxidation at 5-hydroxymethylcytosine
Liu, M. Y., Torabifard, H., Crawford, D. J., DeNizio, J. E., Cao, X.-J., Garcia, B. A., Cisneros, G. A., & Kohli, R. M. (2017) · Nature Chemical Biology · doi:10.1038/nchembio.2250 · Cited by 78
Mutation in TET2 in Myeloid Cancers
(2009) · New England Journal of Medicine · doi:10.1056/nejmc091348 · Cited by 66
Zhao, C., Xiu, Y., Ashton, J., Xing, L., Morita, Y., Jordan, C. T., & Boyce, B. F. (2012) · Stem Cells · doi:10.1002/stem.1050 · Cited by 65
Guan, Y., Tiwari, A. D., Phillips, J. G., Hasipek, M., Grabowski, D., Pagliuca, S., Gopal, P., Kerr, C. M., Ademà, V., Radivoyevitch, T., et al. (2020) · Blood Cancer Discovery · doi:10.1158/2643-3230.bcd-20-0173 · Cited by 64
Selective targeting of TET catalytic domain promotes somatic cell reprogramming
Singh, A. K., Zhao, B., Liu, X., Wang, X., Li, H., Qin, H., Wu, X., Ma, Y., Horne, D. A., & Yu, X. (2020) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.1910702117 · Cited by 63
Self-citationWu, R., Sun, C., Chen, X., Yang, R., Luan, Y., Zhao, X., Yu, P., Luo, R., Hou, Y., Tian, R., et al. (2024) · Proceedings of the National Academy of Sciences · doi:10.1073/pnas.2321611121 · Cited by 63
Self-citationHenriksen, J. R., Løkke, C., Hammerø, M., Geerts, D., Versteeg, R., Flægstad, T., & Einvik, C. (2007) · Nucleic Acids Research · doi:10.1093/nar/gkm193 · Cited by 39
Rinf Regulates Pluripotency Network Genes and Tet Enzymes in Embryonic Stem Cells
Ravichandran, M., Lei, R., Tang, Q., Zhao, Y., Lee, J., Ma, L., Chrysanthou, S., Lorton, B. M., Cvekl, A., Shechter, D., et al. (2019) · Cell Reports · doi:10.1016/j.celrep.2019.07.080 · Cited by 23
MBD5 and MBD6 stabilize the BAP1 complex and promote BAP1-dependent cancer
Tsuboyama, N., Szczepanski, A. P., Zhao, Z., & Wang, L. (2022) · Genome Biology · doi:10.1186/s13059-022-02776-x · Cited by 21
Talkhoncheh, M. S., Subramaniam, A., Magnusson, M., Kumar, P., Larsson, J., & Baudet, A. (2018) · Haematologica · doi:10.3324/haematol.2018.188466 · Cited by 9
Promotion of Erythropoietic Differentiation in Hematopoietic Stem Cells by SOCS3 Knock-Down
Liu, Y.-X., Dong, X., Gong, F., Su, N., Li, S.-B., Zhang, H.-T., Liu, J.-L., Xue, J.-H., Ji, S.-P., & Zhang, Z. (2015) · PLOS ONE · doi:10.1371/journal.pone.0135259 · Cited by 5
Self-citationAbou-Jaoude, A., Huang, C.-Y., Flores, J. C., Ravichandran, M., Lei, R., Chrysanthou, S., & Dawlaty, M. M. (2022) · Stem Cell Research · doi:10.1016/j.scr.2022.102770 · Cited by 4
Cited by
Crosstalk between metabolism and epigenetics during macrophage polarization
Zhang, K., & Jagannath, C. (2025) · Epigenetics & Chromatin · doi:10.1186/s13072-025-00575-9 · Cited by 141
RNA modifications in gene regulation: Functions and pathways
Wei, J., & He, C. (2026) · Cell · doi:10.1016/j.cell.2026.01.006 · Cited by 48
Self-citationAdvances in understanding LINE-1 regulation and function in the human genome
Li, X., & Liu, N. (2025) · Trends in Genetics · doi:10.1016/j.tig.2025.04.011 · Cited by 36
Detection, molecular function and mechanisms of m5C in cancer
Zhang, L., Li, Y., Li, L., Yao, F., Cai, M., Ye, D., & Qu, Y. (2025) · Clinical and Translational Medicine · doi:10.1002/ctm2.70239 · Cited by 30
Self-citationThe RNA Revolution in the Central Molecular Biology Dogma Evolution
Haseltine, W. A., & Patarca, R. (2024) · International Journal of Molecular Sciences · doi:10.3390/ijms252312695 · Cited by 29
Metadata
- Authors
- Zou, Z., Dou, X., Li, Y., Zhang, Z., Wang, J., Gao, B., Xiao, Y., Wang, Y., Zhao, L., Sun, C., Liu, Q., Yu, X., Wang, H., Hong, J., Dai, Q., Yang, F.-C., Xu, M., & He, C.
- Affiliations
- Howard Hughes Medical Institute (US)
- The University of Texas at San Antonio Health Science Center (US)
- Corresponding author
- Xu, Mingjiang
- He, Chuan
- ORCID
- Venue
- Nature
- Published
- 2024-10-02
- Volume
- 634
- Issue
- 8035
- Pages
- 986-994
- ISSN
- 0028-0836 (ISSN-L)
- 1476-4687
- PMC
- PMC11499264
- OpenAlex
- W4403063005
- Semantic Scholar
- 81d7e928494c9361d190cda57390e07758803b5f
- Cited by
- 103
- References
- 65
- Citations by year
- 2026: 53 · 2025: 44 · 2024: 5
- FWCI
- 28.59
- Type
- journal article
- Language
- en
- Open access
- hybrid
- doi.org
- Locations
- Nature (publishedVersion, cc-by)
- PubMed Central (publishedVersion, cc-by-nc-nd)
- PubMed (publishedVersion)
- RePEc: Research Papers in Economics (submittedVersion)
- Knowledge@UChicago (University of Chicago) (submittedVersion)
- University of Chicago
- Funders
- National Institutes of Health
- National Heart, Lung, and Blood Institute (R01HL145883, R01HL146664, R01HL174477)
- National Human Genome Research Institute (RM1HG008935)
- National Cancer Institute (R01CA285299)
- Topics
- Health Sciences › Medicine › Hematology › Acute Myeloid Leukemia Research
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › Epigenetics and DNA Methylation
- Life Sciences › Biochemistry, Genetics and Molecular Biology › Molecular Biology › RNA modifications and cancer
- Keywords
- TET2, 5-methylcytosine oxidation, histone deubiquitination, open chromatin, chromatin regulation, leukemogenesis, myeloid neoplasms, hematopoietic stem cells, hematopoiesis, therapeutic target
- MeSH terms
- Cell Self Renewal, Animals, Chromatin, DNA-Binding Proteins, Female, Hematopoiesis, Histones, Humans, Leukemia, Male, Mutation, Oxidation-Reduction, RNA, Transcription, Genetic, Retroelements, 5-Methylcytosine, Cell Proliferation, Dioxygenases, Mice, Ubiquitination, Carcinogenesis
About these checks
Registry, retraction, Cites and statistics results are computed, not judged, with one exception: a printed reference that no index lists is read once by a model before it counts as a citation error. Claims are extracted by a model and kept only when their quote appears verbatim in the text; each cited source is then checked, with a model’s help, for whether it says what the claim relies on. Those verdicts can be wrong — read the claim’s quote and the cited source before relying on one.
A language model drew the claims from the paper on 2026-11-12, under version 3 of the claim definition (model deepseek-v4.1-flash, prompt extract-v3).
A second model labelled each claim on 2026-11-12 (model jev-1.13-20260917, definition revision gold-guideline-v0.2).
Statistics and arithmetic are recomputed, not judged.
Confidence bands are shown only for fields calibrated on our annotated test set. None is calibrated yet, so no band is shown.
What counts as a claim ›How we measure confidence ›How we check this ›
Are you an author, or do you see a problem with this page? Request a review
